Relation between longevity and size—Longevity and the
period of growth—Longevity and the doubling in weight
after birth—Longevity and rate of reproduction—Probable
relation between longevity and the nature of the food
The duration of the life of animals varies within very
wide limits. Some, as for instance, the males of certain
wheel animalculæ (Rotifera) complete their cycle of life
from birth to death in 50 or 60 hours, whilst others, like
some reptiles, live more than 100 years, and quite possibly
may live for two or three centuries.
Enquiry has been made for many years as to whether
there are laws governing these different durations of life.
Even the most casual observation of domesticated animals
has shown that, as a general rule, small animals do not
live so long as large ones; mice, guinea pigs, and rabbits
for instance, have shorter lives than geese, ducks, and
sheep, whilst these again are survived by horses, deer,
and camels. Of all the mammals which have lived under
the protection of man, the elephant is at once the largest,
and the most long-lived.
However, it is not difficult to show that there is no
absolute relation between size and longevity, since parrots,
ravens, and geese live much longer than many mammals,
and than some much larger birds.
As a general rule it may be said that a large animal takes
more time than a small one to reach maturity, and it has
been inferred from this that the length of the periods of
gestation and of growth were in proportion to the longevity.
Buffon28 long ago stated his opinion that the “total
duration of life bore some definite relation to the length
of the period of growth.” Therefore, as the period of
growth is, so to say, inherent in the species, longevity
would have to be regarded as a very stable phenomenon.
Just as any species has acquired a fixed and practically
invariable size, so it would have acquired a definite longevity.
Buffon, therefore, thought that the duration of life
did not depend on habits or mode of life, or on the nature
of food, that, in fact, nothing could change its rigid laws,
except an excess of nourishment.
Taking as his standard the total period of development
of the body, Buffon came to the conclusion that the duration
of life is six or seven times that of the period of
growth. Man, for instance, he said, who takes 14 years
to grow, can live 6 or 7 times that period, that is to say,
90 or 100 years. The horse, which reaches its full size
in 4 years, can live 6 or 7 times that length of time, that
is to say from 25 to 30 years. The stag takes 5 or 6
years to grow, and reckoned in the same way, its longevity
should be 35 to 40 years.
Flourens29 although supporting his principle, thought
that Buffon had been inexact in calculating the period
of growth. In his opinion a better result can be obtained
by taking the limit of growth as that age at which the
epiphyses of the long bones unite with the bones themselves.
Using such a mode of computation, Flourens laid
down that an animal lived 5 times the length of its period
of growth. Man, for instance, takes 20 years to grow, and
he can live for 5 times that space, that is to say, 100 years;
the camel takes 8 to grow, and lives 5 times as long,
i.e., 40 years; the horse, 5 to grow, and lives 25 years.
However, even if we consider only the mammalia, it is
impossible to accept Flourens’ law, without considerable
reserve. Weismann30 has referred to the case of the horse,
which is completely adult at 4, but lives not merely 5
times that period, but 10 or even 12 times. Mice grow
extremely quickly, so that they are able to reproduce at
the age of 4 months. Even if we take 6 months as their
period of growth, their longevity of 5 years is twice as
long as it would be according to the rule of Flourens.
Amongst domesticated animals, the sheep is slow in reaching
maturity; it does not acquire its adult set of teeth until
it is 5 years old, and cannot be regarded as adult until
then. None the less, at the age of 8 or 10 years, it loses
its teeth and begins to grow old, whilst by 14 it is quite
senile.31 The longevity of the sheep, therefore, is not quite
three times its period of growth.
If we turn to other vertebrates, the variations in the
relation of growth and the duration of life are still greater.
Parrots, for instance, the longevity of which is extremely
great, grow very quickly. At the age of 2 years, they
have acquired the adult plumage and are able to reproduce,
whilst the smaller species are in the same condition
at the age of one. Incubation, moreover, is very short,
not more than 25 days, and in some species not three
weeks. None the less, parrots are birds which enjoy a
quite remarkable longevity. The incubation period of
domestic geese is 30 days, and their period of growth is
also short. However, they may reach a great age, cases
of 80 years and of 100 years being on record. In contrast
with these, ostriches, the incubation period of which is
42 to 49 days, and which take 3 years to become adult,
have a relatively short life.
H. Milne-Edwards32 many years ago contended that
there was no importance in the supposed law of relation
between gestation and longevity. He sums up his criticism
as follows: “Although the period of uterine life is longer
in the horse, that animal does not live so long as a human
being; and some birds, the incubation of which only lasts
a few weeks, can live more than a century.”
Bunge33 has recently taken up the study of the relations
between the duration of growth and longevity, and has
suggested a new means of investigation. He has observed
that the period in which the new-born mammal doubles
its weight is a good index of the rapidity of its growth.
He has shown that whilst a human child requires 180
days to reach double its weight at birth, the horse, the
longevity of which is very much less, doubles its weight
in 60 days; a calf takes only 47 days for this; a kid 15
days; a pig 14 days; a cat 9-1/2; and a dog only 9 days.
Although these facts are very interesting, the exceptions
are too great to make it possible to base a law of longevity
upon them. The period of weight-doubling in the horse
is nearly 7 times longer than that in the dog, and yet the
longevity of the horse is not more than 3 times that of
the dog. The goat, which takes much longer than the
dog to double its weight, has a shorter total life.
I observed myself that new-born mice quadruple their
weight in the first 24 hours. The doubling of weight
in their case requires a time 36 times less long than that
of the cat, and yet the cat lives only 5 times as long as
the mouse.
It is fair to say, however, that Bunge himself does not
draw a definite conclusion from these figures and has
published them only to stimulate interest in the subject.
He is against the view of Flourens, and points out that
although the multiple 5 is valid for man, it is not so in
the case of the horse which finishes its growth in 4 years
and yet reaches the age of 40 much less often than human
beings attain that of 100 years.
Although it is impossible to admit the existence of
exact relations between size and the period of growth on
the one side, and longevity on the other, in the mode
which Buffon and Flourens have followed, it is none the
less true that there is something intrinsic in each kind
of animal which sets a definite limit to the length of years
it can attain. The purely physiological conditions which
determine this limit leave room for a considerable amount
of variation in longevity. Duration of life therefore, is
a character which can be influenced by the environment.
Weismann in his well-known essay on the duration of
life, has laid stress on this side of the problem. Longevity,
according to him, although in the last resort depending
on the physiological properties of the cells of which the
organism is composed, can be adapted to the conditions
of existence and influenced by natural selection, like other
characters useful for the existence of the species.
If a species is to remain in existence, its members must
be able to reproduce and the progeny must be able to
reach adult life so that they in their turn may reproduce.
Now, it happens that there are some animals the fecundity
of which is extremely limited. Most birds which are
adapted to aerial life, and the weight of which is therefore
to be kept down, lay very few eggs. This happens in
the case of birds of prey, such as eagles and vultures.
These birds nest only once a year, and generally rear two
or frequently only a single nestling. In such circumstances
the duration of life becomes a factor in the preservation
of the species, more important since eggs and chicks
are subject to many dangers. Eggs are devoured by many
kinds of animals, whilst unseasonable cold may kill the
chicks. If the members of such a species were incapable of
living long, the unfavourable conditions of life would soon
lead to extinction. Those animals which reproduce rapidly
generally have a relatively brief duration of life. Mice, rats,
rabbits, and many other rodents seldom live more than 5 or
10 years, but reproduce with enormous rapidity. It is almost
possible to imagine that there is some sort of intimate link,
possibly physiological, between longevity and low fertility.
It is a current opinion that reproduction wastes the maternal
organism and that mothers of many children grow old
prematurely and seldom reach an advanced age. This
would seem to mean that fecundity was the cause of the
short duration of life. However, we must guard ourselves
against such a theory. Longevity, at least in the case of
vertebrate animals, differs extremely little in the two sexes,
although the cost of the new generation to the adult
organism is very much greater in the case of the female
than of the male parent. None the less, females frequently
reach a great age, especially in the human race where
women reach 100 years, or live beyond that time, much
more often than men.
Low fertility, however, cannot itself be regarded as a
cause of longevity, as there are some very fertile animals
which none the less attain great ages. There are parrots
which lay two or three times a year, producing six to nine
eggs in each clutch. The ducks (Anatidæ) are distinguished
for considerable longevity and very high fertility, each
nest containing rarely less than six and sometimes as many
as sixteen eggs. The common Sheldrake lays from twenty
to thirty eggs. Tame ducks, in some parts of the tropics,
lay an egg daily throughout the season. Wild ducks lay
from seven to fourteen eggs in one nest. Ducks and geese,
none the less, frequently attain considerable ages, ducks
having been known to live for 29 years. Even the common
fowl, which is a notoriously prolific bird, may reach an age
of twenty to thirty years.
It will be said, however, that these birds are exposed to
many enemies during youth. Chickens, ducklings, and
goslings are ready prey for hawks, foxes and small carnivora.
The longevity is possibly to be explained as an
adaptation for the preservation of the species by compensating
for the great destruction of the young. Weismann
explains in this way the longevity of many aquatic birds
and other creatures that are much preyed on. It must be
noted, however, that the longevity cannot depend on the
risks run by the young birds, but must have arisen independently.
If this had not occurred, creatures, the young
of which are destroyed in great numbers, would have ceased
to exist, as many species have disappeared in geological
time. The longevity of prolific animals, the young of
which are destroyed in numbers, must be due to some
cause which is neither fertility nor the destruction of their
offspring. This cause must be sought in the physiological
processes of the organism and can be attributed neither to
the length of the period of growth nor to the size attained
by the adults.
After having discussed various theories of the cause of
the duration of life, M. Oustalet,34 in a most interesting essay
on the longevity of vertebrates, came to the conclusion that
diet was the chief factor. He thinks that there is a
“definite relation between diet and longevity. For the most
part herbivorous animals live longer than carnivorous
forms, probably because the former find their food with
ease and regularity, whilst the latter alternate between
semi-starvation and repletion.” There are certainly many
instances which give support to the view. Elephants and
parrots, for instance, are vegetarian and reach very great
ages. On the other hand, there exist long-living carnivorous
animals. Many observations have made it certain
that owls and eagles reach great ages, and these birds live
on animal food. Ravens, which live on carrion, are also
notorious for the duration of their lives. There is no exact
knowledge as to the ages reached by crocodiles, but
although these live on flesh, it is certain that their longevity
is great.
We must seek elsewhere for the real factors that control
duration of life. Before stating my conclusion, I will
review what is known as to the duration of life of different
animals.
Longevity in the lower animals—Instances of long life in
sea-anemones and other invertebrates—Duration of life of
insects—Duration of life of “cold-blooded” vertebrates—Duration
of life of birds—Duration of life of mammals—Inequality
of the duration of life in males and females—Relations
between longevity and fertility of the organism
It is wonderful to what an extent the duration of life varies
amongst animals, the slightest examination of the facts
showing that very many factors must be involved.
As the higher animals are nearly always larger than
invertebrates, if there be a definite relation between longevity
and size, one would expect to find that vertebrates
live longer than invertebrates. However, this is not the
case. Amongst animals of extremely simple organisation,
there are some which reach a great age. A striking
example of this is found in sea-anemones. These animals
have a very simple structure, without a separate digestive
canal, and with a badly developed, diffused nervous system,
and yet have lived very long in captivity. More than forty
years ago, I remember having seen in the possession of
M. Lloyd, the Director of the Aquarium at Hamburg, an
anemone that he had kept alive for several dozen years in
a glass bowl. Another sea-anemone, belonging to the
species Actinia mesembryanthemum, is known to have
lived 66 years. It was captured in 1828 by Dalyell, a
Scottish zoologist, and was then quite adult, and probably
about 7 years old. It survived its owner for 36 years, and
died in Edinburgh in 1887, the cause of death being unknown.
Although they are thus capable of living so long,
the rate of growth of members of this species is rapid, and
their fertility is very high. According to Dalyell, these
anemones reach the adult condition in 15 months. The
specimen in his possession, in the 20 years from 1828 to
1848 produced 334 larvæ, then after a period of sterility it
gave birth, in one night (1857) to 230 young anemones.
This extraordinary prolificness decreased with age, but even
when it was 58 years old it used to produce from 5 to 20 at
a time. In the seven years from 1872 onwards, it gave birth
to 150 young anemones.35 This animal, which certainly
was not more than the fortieth or the fiftieth of the weight
of an adult rabbit, lived six or seven times as long.
Ashworth and Nelson Annandale have published their
observations on another sea-anemone, of the species Sagartia
troglodytes, which was 50 years old. It differed from
younger examples only in being less prolific.
There are other polyps, such as Flabellum, which do not
live more than 24 years, although we have no knowledge as
to the cause of the different duration of life.
The variation in the length of the life of molluscs and
insects is extremely great. Some species of gasteropods
(Vitrina, Succinea) live only a very few years, whilst
others (Natica heros) can reach thirty years. Some of the
marine bivalves, as for instance, Tridacna gigas, can live
to sixty or a hundred years.36
Insects are animals as variable in their duration of life as
they are in other respects. Some live only a few weeks;
some of the plant-lice, for instance, die in a month. In
the same order of Insects, however, (Hemiptera) there are
species of cicada which live thirteen to seventeen years, that
is to say, much longer than such little Rodents as rats,
mice, and guinea-pigs. The larva of an American species
spends seventeen years buried in the ground in orchards,
where it feeds on the roots of apple trees, and the species is
known as Cicada septemdecim, because of this duration of
life. In the adult stage the insect lives little more than a
month, just time enough to lay the eggs, and bring into
the world the new generation, which in its turn will not
appear above ground until after another period of seventeen
years.
Between these extremes of long and short life, there is
to be found amongst insects almost every gradation of
longevity. Science, in its present state, has failed to find
any law governing these facts. Rules which hold good up
to a certain point in the case of the higher animals break
down in their application to insects. The large grasshoppers
and locusts, for instance, live a much shorter time
than many minute beetles. Queen bees, the fertility of
which is very great, live two or three years and may reach
a fifth year, whilst worker bees, which are infertile, die in
the first year of their existence. Female ants, although
these are small and extremely prolific, reach the age of
seven years.37
We know so little about the physiological processes of
insects, that we cannot as yet make even a guess at the
cause of this great variation in their longevity. It is more
probable that we shall find some explanation in the case of
vertebrates concerning which we know much more.
Analysis of the facts shows that whilst in the evolution
from fish to mammal there has been a great increase in
complexity of organisation, there has at the same time been
a reduction in the duration of life. As a general rule, it
may be laid down that the lower vertebrates live longer
than mammals.
The facts about the longevity of fish are not very numerous,
but it seems clear that these animals reach a great
age. The ancient Romans, who used to keep eels in
aquaria, have noted that these fish would live for more than
sixty years. There is reason to believe that salmon can
live for a century, whilst pike live much longer. There is,
for instance, the much quoted instance of the pike stated
by Gessner to have been captured in 1230 and to have lived
for 267 years afterwards. Carps are regarded as equally
long lived, Buffon setting down their period of life as 150
years. There is a popular idea that the carp in the lakes
at Fontainebleau and Chantilly are several centuries old,
but E. Blanchard throws doubt on the accuracy of this estimate,
inasmuch as during revolutionary times most of the
carp were eaten when the palaces were overrun by the populace.
There is no doubt, however, that the life of carp
may be very long indeed. Not very much is known about
the duration of life in batrachians, but it is certain at least
that some small frogs may live twelve or sixteen years, and
toads as many as thirty-six years.
More is known about the life of reptiles. Crocodiles and
caymans, which are large and which grow very slowly,
attain great ages. In the Paris Museum of Natural History
there are crocodiles which have been kept for more than
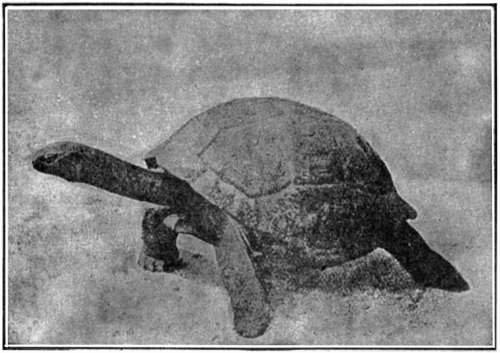
forty years without showing signs of senescence. Turtles,
although they are smaller than crocodiles, live still longer.
A tortoise has lived for eighty years in the garden of the
Governor of Cape Town, and is believed to have reached
the age of two hundred years. Another tortoise, a native
of the Galapagos Islands, is known to be 175 years old,
whilst a specimen in the London Zoological Gardens is 150
years old. A land tortoise (Testudo marginata) has been
kept in Norfolk, England, for a century. I am informed
that in the Archbishop’s palace at Canterbury, there is to
be seen the carapace of a tortoise which was brought to the
Palace in 1623 and which lived there for 107 years.38 Another
tortoise, brought to Fulham by Archbishop Laud, lived in
the Palace for 128 years. I have already referred to a
specimen of Testudo mauritanica, the history of which is
known for 86 years, but which is probably much older.
Very little is known as to the longevity of lizards and
serpents, but it may be inferred from what I have said about
other reptiles that reptiles as a class are able to reach great
ages.
It is an easy inference that the great duration of life in
cold-blooded animals is associated with the slowness of
the physiological processes in these creatures. The circulation,
for instance, is so slow, that the heart of a tortoise
beats only 20 to 25 times in a minute. Weismann has
suggested that one of the factors influencing the duration
of life is the rapidity or slowness of the vital activities, the
times taken by the processes of absorption and nutrition.
On the other hand, the blood is hot and the vital activities
are rapid in birds, and yet birds may attain great ages.
Although in the last chapter I gave a number of examples,
the subject is so important that I propose to go further into
details. The possibility of this is due to an admirable set
of details brought together by Mr. J. H. Gurney.39 In his
list, in which are included more than fifty species of birds,
the lowest figures are from eight and a half to nine years
(Podargus cuvieri, Chelidon urbica), and a duration of life
so short is an exception, a period of from fifteen to twenty
years being more common. Canaries have lived in captivity
from 17 to 20 years, and goldfinches up to 23 years.
Field larks have lived for 24 years, the Lesser Black-backed
Gull 31 years and the Herring Gull 44 years. Birds of
medium size may live for several dozens of years, whether
they live on animal or on vegetable food, whether they are
prolific or lay very few eggs. I will quote only a few
instances. Of forty parrots the minimum and maximum
ages were respectively 15 and 81 years, and the average 43
years. Without accepting the truth of the story mentioned
by Humboldt according to which certain parrots survived
an extinct race of Indians, at least we may be certain that
great ages have sometimes been reached by these birds.
Levaillant mentions a parrot (Psittacus erithaceus) which
lost its memory at the age of 60 years, its sight at 90
years, and which died aged 93 years. Another individual,
probably of the same species, is reported by J. Jennings
to have reached the age of 77. Jones, Layard, and Butler
are the authorities for instances of Sulphur-crested Cockatoos
having reached respectively 30, 72 and 81 years. M.
Abrahams states that an Amazon (Chrysotis amasonica)
lived 102 years. I myself have observed two cases of great
longevity in the same species of parrot. One of these birds
died at the age of 82 years, apparently simply from old
age, whilst the other, which was in my possession for
several years before it died at the age of 70 to 75 years, was
vigorous, showing no signs of senility, but died of pneumonia.
Mr. Gurney found that parrots were not the only birds
capable of reaching a great age. One raven reached 69
years and another 50, an Eagle-owl (Bubo maximus) 68
years, another 53, a condor 52, an imperial eagle 56, a common
heron 60, a wild goose 80, and a common swan 70
years. None of these examples approaches the legendary
three centuries attributed to the swan, but it is evident that
many different kinds of birds may attain great age. I can
add some cases to those of Mr. Gurney. In the Royal Park
at Schönbrunn, near Vienna, a white-headed vulture (Neophron
percnopterus) died aged 118 years, a golden eagle
(Aquila chrysaëtus) aged 104, and another aged 80 (according
to Oustalet). Mr. Pycraft (Country Life, June 25th,
1904) reported that a female eagle, captured in Norway in
1829, had been brought to England and had lived for 75
years. In the last thirty years of its life, it had produced
ninety eggs. The same writer mentions the case of a falcon
having lived to 162 years.
The collection of facts that I have passed in review make
it manifest that birds may have a great duration of life,
but that reptiles surpass them in this respect. Birds certainly
do not reach the very great ages of crocodiles and
tortoises.
Longevity, therefore, is reduced as we ascend in the
scale of vertebrate life. We find a still greater reduction
when we turn from birds to mammals. Some mammals,
it is true, may live as long as birds. Elephants are a
good instance. It used to be thought that these giant
mammals could live three or four centuries, but I can find
no confirmation of the legend, which seems as mythical
as that relating to the life of swans. There are no exact
data as to the ages reached by wild elephants, but it has
been stated that in captivity an elephant rarely but occasionally
has completed its century. In zoological gardens
and in good menageries, where elephants are well cared
for, they seldom live more than 20 to 25 years. Chevrette,
an African elephant presented to the Jardin des Plantes
by Mehemet Ali, in 1825, lived for only 30 years. In the
official list of the Indian Government, which gives the
deaths of elephants, it appears that of 138 examples, only
one lived more than 20 years after it had been purchased
(Brehm’s Mammals).
Flourens, using his own formula, assigned the age of
150 years to elephants as their epiphyses do not fuse with
the long bones until the age of 30. So far, I know of no
fact to support the conclusion, although it seems fairly well
established that occasionally an elephant may reach a
century. It is stated that one elephant was in service
throughout the whole period of more than 140 years in
which Ceylon was occupied by the Dutch. This elephant
was found in the stables in 1656. Natives with special
knowledge of elephants set down their duration of life
as from 80 to 150 years, but say that they begin to grow
old at from 50 to 60 years of age. My general conclusion
from the facts is that the life of these very large mammals
is about the same as that of man who is very much
smaller.
Centenarians, extremely rare amongst elephants, do not
appear to exist in any other kind of mammals except man.
The rhinoceros, another large mammal which is a native
of the same countries as the elephant, does not reach a
great age. According to Oustalet an Indian rhinoceros
died in the menagerie of the Paris Museum at about the
age of 25 years, and showed all the signs of senility.
Another Indian rhinoceros lived for 37 years in the London
Zoological Gardens. Grindon has stated his opinion that
the rhinoceros may live for 70 or 80 years, but this seems
rather an inference from the slowness of growth than a
statement of observed fact.
Horses and cattle are large animals, but do not enjoy
very long lives. The usual duration of life in horses is
from 15 to 30 years. They begin to grow old about 10
years, and in very rare cases may reach 40 or more. A
Welsh pony is said to have reached the age of sixty, but
such a case is excessively rare. Two other extreme cases
are that of a horse belonging to the Bishop of Metz which
died at the age of 50 years, and the charger of Field-Marshal
Lacy which died at 46.
The duration of life of cattle is still shorter. Domestic
cattle show the first sign of age, a yellow discoloration
of the teeth, when five years old. In the sixteenth to
eighteenth year the teeth fall out, or break, and the cow
ceases to give milk, whilst the bull has lost reproductive
power. According to Brehm, cattle live for 25 to 30 years
or more. Although the duration of life is short, cattle
are not prolific. The gestation period of a cow approaches
that of the human race (242-287 days), and there is only
one birth a year. The total period of reproductivity lasts
only a few years.
The sheep, another domesticated Ruminant, has a life
even shorter. According to Grindon, sheep do not live
longer than 12 years as a rule, but may reach 14 years,
which in their case would be extreme age, as they generally
lose their teeth at from 8 to 10 years.
Some Ruminants, such as camels and deer, apparently
live longer than sheep or cattle, but I do not know exact
facts about them.
The short life of domesticated carnivorous animals is
well known. Dogs seldom live more than 16 or 18 years,
and even before that, at an age of from 10 to 12, they
usually show plain signs of senility. Jonatt has mentioned
as an extreme rarity a dog of 22 years of age, and Sir E.
Ray Lankester (Comparative Longevity, p. 60) cites
another instance, in this case the age being 34 years. The
oldest dog that I have been able to procure died at the
age of 22.
It is generally believed that cats do not live so long as
dogs. The average age which they may attain is usually
thought to be 10 or 12 years, but certainly a cat of that
age has not the decrepid appearance of an old dog. Thanks
to the kindness of M. Barrier, the Director of the Ecole
d’Alfort, I have had in my possession a cat 23 years old.
It appeared to be quite vigorous, and died from cancer
in the liver.
Most rodents, particularly the domesticated kinds, are
extremely prolific and very short lived. It is extremely
rare for a rabbit to reach the age of 10 years, whilst 7
years is the utmost limit for a guinea-pig. Mice, so far
as I can ascertain, do not live more than 5 or 6 years.
It is plain from the facts that I have brought together,
that mammals, whether they are large or small, as a rule,
have shorter lives than birds. It is probable, therefore,
that there is something in the structure of mammals which
has brought about a shortening in the duration of their
lives.
Whilst most of the lower vertebrates, and all birds,
reproduce by laying eggs, the vast majority of mammals
are viviparous. As the tax on the parent organism is
greater when the young are produced alive than when
eggs are laid, it might be thought that in this difference
lay the cause of the shorter life of mammals. It is well
known that an animal may be made feeble by too great
fecundity, and it is conceivable that the kind of parasitic
life of the embryos within the body of the mother may
weaken her system.
There are many facts, however, which make it impossible
to accept such a view. The longevity of mammals
is nearly equal in the two sexes, although the tax on the
organism caused by reproduction is much greater in the
case of females than in males. Longevity, however,
cannot be regarded as a character stable in each species
and necessarily identical in the two sexes. The animal
kingdom presents many cases of disparity in this respect,
the difference in longevity in the two sexes being specially
striking in species of insects. Generally, the females live
longer than the males, as, for instance, amongst the Strepsiptera,
where the females have 64 times the duration of
life of the males. On the other hand, amongst butterflies,
there are cases (e.g., Aglia tau) where the males live longer
than the females. In the human race, there is a difference
in the longevity of the sexes, the females having the
advantage.
As in most cases of disparity in the duration of life the
female lives longer than the male, it is plain that the difference
cannot be assigned to the drain on the organism
caused by reproduction, which, of course, is much greater
in females.
Moreover, a closer scrutiny of the facts shows that
although mammals do not live so long as birds, the reproductive
drain is greater in the case of birds.
It is well known that the productivity of an animal is
not necessarily identical with its fecundity. Fish or frogs
which lay thousands of eggs at a time (a pike, for example,
produces 130,000) are obviously more prolific than, for
instance, a sparrow which lays only 18 eggs in a year,
or than a rabbit, which in the same time gives birth to
from 25 to 50. However, to produce this much smaller
quantity of eggs or of young, the sparrow and the rabbit
(I have chosen the most prolific bird and mammal) expend
a much larger quantity of material than the frog or the
fish. The sparrow and the rabbit employ in producing
their progeny a bulk of material greater than the weight
of their body, whilst the enormous quantity of eggs laid
by the frog does not weigh more than one-seventh part of
the body of the frog. It may be laid down, as a general
rule, that although fecundity, that is to say the number
of eggs or of young which are produced, diminishes as
the organism becomes more complex, the productivity on
the other hand increases, expressed in percentage of weight.
The productivity, which is not more than 18 per cent. in
batrachia, reaches 50 per cent. in reptiles, 74 per cent.
in mammals, and 82 per cent. in birds.
It is plain that if reproduction shortens the life of
mammals by weakening the organism, it must be the
productivity, not the fecundity, which is the important
factor. I have just shown that productivity is greater in
birds than in mammals, and in consequence it cannot be
on account of any greater burden of reproduction that
mammals have a shorter life than birds. The shortness
of mammalian life, again, cannot be attributed to the fact
that mammals give birth to young, whilst the long-lived
reptiles and birds produce eggs, because the longevity of
the males, which produce neither young nor eggs, is none
the less practically equal to that of the females of the same
species. The reason of the short life of mammals must
be sought for elsewhere.
Relations between longevity and the structure of the digestive
system—The Cæca in birds—The large intestine of mammals—Function
of the large intestine—The intestinal microbes
and their agency in producing auto-intoxication and auto-infection
in the organism—Passage of microbes through the
intestinal wall
We have seen that the duration of life in mammals is
relatively shorter than that in birds, and in the so-called
“cold-blooded” vertebrates. No indication as to the cause
of this difference can be found in the structure of the organs
of circulation, respiration, or urinary secretion, or in the
nervous or sexual apparatus. The key to the problem is
to be found in the organs of digestion.
In reviewing the anatomical structure of the digestive
apparatus in the vertebrate series, one soon comes to the
striking fact that mammals are the only group in which the
large intestine is much developed. In fish, the large intestine
is the least important part of the digestive tube, being
little wider in calibre than the small intestine. Amongst
batrachia, where it is a relatively wide sack, it has begun
to assume some importance. In several reptiles it is still
larger, and may be provided with a lateral out-growth,
which is to be regarded as a cæcum. In birds, the large
intestine still remains relatively badly developed; it is
short and straight. In most birds, at the point where the
large intestine passes into the small intestine, there is a
pair of cæca, more or less developed. These cæca are
absent in climbing birds, such as the wood-pecker, the
oriole, and many others. They are reduced to a pair of
tiny outgrowths in the eagles, sparrow-hawks, and other
diurnal birds of prey, and in pigeons, and perching birds.
These organs are larger in the nocturnal birds of prey, in
gallinaceous birds, and in ducks, etc.40
In the large running birds, such as ostriches, rheas, and
tinamous, the cæca are relatively largest. Thus, for
instance, in a rhea (Rhea americana) which I dissected, the
cæca were nearly two-thirds as long as the small intestine.
The latter was 1·65 m. in length, whereas one of the cæca
was 1·01 m., and the other 0·95 m. The weight of the
two cæca with their contents was more than 10 per cent.
of the total weight of the bird.
Notwithstanding the exceptions, which are relatively
rare, the large intestine is badly developed in the case
of birds. On the other hand, it reaches its largest size
amongst mammals. In these animals, “only the posterior
portion of the latter, or rectum, which passes into the
pelvic cavity, corresponds to the large intestine of
lower Vertebrates; the remaining, and far larger part,
must be looked upon as a neomorph, and is called the
colon.”41
Gegenbaur,42 another well-known authority on comparative
anatomy, writes as follows on this subject:—“The
hind-gut is longest in the Mammalia, where it forms the
large intestine, and is distinguished as such, from the
mid-gut, or small intestine. Owing to its greater length,
it is arranged in coils, so that the terminal portion only
has the straight course taken by the hind-gut of other
Vertebrata.”
The two series of facts are not to be disputed. On the
one hand mammals are shorter lived than birds and lower
vertebrates, on the other hand the large intestine is much
longer in them than in any other vertebrates. Is there
here any link of causality, binding the two characters, or
is it a mere coincidence?
To answer the question we must turn to the function of
the large intestine in vertebrates. In the lower members
of the group (fish, batrachia, reptiles, birds, etc.), the
large intestine is not more than a mere reservoir for the
waste matter in the food. It takes no share in digestion,
as that is the function of the stomach and the small intestine.
Only the cæcum can be thought to have some
digestive property. In reptiles, the lowest vertebrates in
which the cæcum is present, it is so little differentiated
from the large intestine itself, that it is difficult to assign
to it any specialised function. In very many birds, however,
the cæca are well separated from the main digestive
tube. The food material passes into them in considerable
quantities, and is retained there sufficiently long
for some digestive process to take place. M. Maumus
has found, in the cæca of birds, secretions which can dissolve
albumen and invert sugar cane, but he has been
unable to make out that the cæcal juice has any action
upon fatty matter. Such digestive power, however, is
slight, and when M. Maumus removed the cæca in fowls
and ducks, no evil consequences followed. As in many
birds the cæca are rudimentary and in others absent, it
may be inferred that these organs are useless, and are
in process of degeneration in the class. The cæca can
be regarded as playing an important part in the organism
only in the case of large running birds, where they are
very highly developed, but we have not precise information
as to their digestive function.
The variations in the structure in the large intestine
are greater in mammals than in birds. In some mammals,
the large intestine is a simple prolongation of the small
intestine, similar in calibre and in structure. In these conditions
it may fulfil a definite digestive function. Th.
Eimer43 has determined that in insectivorous bats the
large intestine digests insects like the small intestine.
Such cases, however, are rare. In most mammals the
large intestine is sharply separated from the small intestine
by a valve, and opens directly into the cæcum which
may be very large. In the horse, the cæcum is an enormous
bag, cylindrical and tapering, generally well filled, and
holding on an average 35 litres. It is equally large in
many other herbivorous animals, such as the tapir, the
elephant, and most rodents. In such cases, the food
remains for a considerable time in the organ and without
doubt undergoes some digestive changes. In many other
mammals, particularly carnivorous forms, the cæcum may
be quite absent, whilst in some, as for instance, the cat
and dog, it is very small; in the latter cases its digestive
function must be non-existent or insignificant.44
As for the large intestine itself, apart from the special
cases, such as bats, it cannot fulfil any notable digestive
function. Th. Eimer was unable to find a proof of any
such action in rats and mice, and the very many investigations
that have been made in the case of man seem to
have established the absence of digestive power in the
colon.
Dr. Stragesco,45 in a recent investigation carried out
under the direction of the famous Russian physiologist
Pawloff, established that, in normal conditions, digestion
and assimilation of food are confined almost exclusively to
the small intestine in mammals, and that the large intestine
plays only the smallest part. It is only in certain
diseases of the digestive tract, in which, on account of
increased peristaltic action, the contents of the intestine
with the digestive juices are passed quickly from the small
intestine to the large intestine, that some digestive work is
done in the latter organ.
The large intestine (excluding the cæcum), then, cannot
be regarded as an organ of digestion, although absorption
of the liquids which have been formed in the
small intestine, may take place within its walls. It is
known that in the large intestine the contents of the gut
give up their water and assume the solid form of fæcal
matter. However, whilst the mucous membrane of the
large intestine rapidly absorbs water, it has not a similar
action on other substances.
The question of the extent to which the large intestine
can absorb has been closely investigated, because of its
practical importance. It sometimes happens that invalids
cannot take food by the mouth, so that their life would be
in danger if it were not possible to supply them with food
otherwise. Attempts have been made to inject nutritive
substances through the skin, or, and this is a more usual
procedure, by the rectum. By such means the organism
can be kept alive for a certain time, but the absorbing
power of the large intestine is extremely small. According
to Czerny and Lautschenberger46 the entire colon of
the human being can absorb no more than 6 grammes of
albumen in 24 hours, an amount which, from the point of
view of nutrition, is very small. It was thought that the
large intestine might more rapidly absorb albuminous
material which had been previously digested and transformed
to peptones, but the experiments of Ewald47 showed
that even in that case the absorption was very small.
According to more recent experiments of Heile,48 carried
out upon dogs which had cæcal fistulas, and in the case
of a man who had an artificial aperture in the colon, the
large intestine does not absorb undigested white of egg,
and absorbs water, cane sugar, and glucose only very imperfectly.
The only substances which are rapidly absorbed
through the wall of the colon are the alkaline fluids
from fæcal matter. It is possible, however, to nourish
invalids by rectal injections of certain nutritious substances,
the most important of which is milk.49
The large intestine, which has really very slight digestive
properties and cannot absorb any considerable bulk
of nutriment, is an organ which secretes mucus. The
latter serves to moisten the solid fæcal material, so aiding
in its expulsion.
We must conclude, therefore, that the large intestine,
the organ so highly developed in mammals, is an apparatus
the general function of which is the preparation and elimination
of the waste products of digestion. Why should
such an organ be so much more developed in mammals
than in the other vertebrates?
In answer to the question, I have formed the theory that
the large intestine has been increased in mammals to make
it possible for these animals to run long distances without
having to stand still for defæcation. The organ, then,
would simply have the function of a reservoir of waste
matter.
Batrachia and reptiles lead a very idle life, and can move
slowly, sometimes because they are protected by poison
(toads, salamanders, serpents), sometimes because they
have a very hard shell (turtles), sometimes because they
are extremely powerful (crocodiles). Mammals, on the
other hand, have to move very actively to catch their prey,
or to escape from their enemies. Such activity has
become possible because of the high development of the
limbs, and because the capacity of the large intestine makes
possible the accumulation of waste matter for a considerable
time.
In order to void the contents of the intestines, mammals
have to stand still and assume some particular position.
Each act of this kind is a definite risk in the struggle for
existence. A carnivorous mammal which, in the process
of hunting its prey, had to stop from time to time, would
be inferior to one which could pursue its course without
pausing. So, also, a herbivorous mammal, escaping from
an enemy by flight, would have the better chance of surviving
the less it was necessary for it to stand still.
According to such a view, the extreme development of
the large intestine would supply a real want in the struggle
for existence. M. Yves Delage,50 the well-known biologist,
is unable to accept this hypothesis. He thinks that the
rectal enlargement would fulfil the purpose, and adds that
everyone has seen herbivorous animals pass their excretions
whilst running. The rectum of mammals, however,
cannot serve as a reservoir for waste matter, because as soon
as such matter reaches the rectum it excites the need of
excretion. The waste matter accumulates in the large intestine,
from which it passes into the rectum at intervals.
When it has reached that region, a sensation is caused
which leads to defæcation.
M. Delage is not quite definite when he speaks of
mammals voiding their excretions whilst they are in
motion. A horse, harnessed to a vehicle, may defæcate
whilst it is walking or even running slowly. But these
animals cannot defæcate when in rapid motion, and competent
observers state that horses never do so whilst racing.
In zoological gardens, where animals have room to run
about, they stand still before emptying the rectum. M.
Ch. Debreuil, who keeps antelopes in a very large park
at Melun, has noticed that the excreta are always to be
found in masses and not scattered about as if they had been
discharged by animals in motion. Antelopes, which are
animals that run and leap extremely actively, have to come
to a standstill before discharging their small pellets of
deer-like excreta.
In the struggle for existence, when a mammal is pursuing
its prey or escaping its enemy, there is no question of the
leisurely movement of a horse harnessed to an omnibus or
cab, but the greatest possible activity is necessary. In
such circumstances the possession of an organ within which
the excreta could accumulate would be of real importance.
My theory of the origin of the mammalian large intestine
is intrinsically probable.
Although the capacity of the large intestine may
preserve a mammal in emergencies, it is attended with
disadvantages that may shorten the actual duration of life.
The accumulation of waste matter, retained in the large
intestine for considerable periods, becomes a nidus for
microbes which produce fermentations and putrefaction
harmful to the organism. Although our knowledge of
the subject is far from complete, it is certain that the intestinal
flora contains some microbes which damage health,
either by multiplying in the organism, or by poisoning it
with their secretions. Most of our knowledge on this
matter has come from the study of human patients.
Persons have been known who do not defæcate except
at intervals of several days, and who, none the less, do not
seem to suffer in health. But the opposite result is more
common. The retention of fæcal matter for several days
very often brings harmful consequences. Organisms
which are in a feeble state from some other cause are specially
susceptible to damage of the kind referred to. Infants
are frequently seriously ill as the result of constipation.
Dr. du Pasquier51 describes such cases in the following
words:—“The infant is leaden in hue, with sunken eyes,
dilated pupils, and pinched nostrils. The temperature may
reach nearly 104° Fahr.; the pulse is rapid, feeble, and often
irregular. Restlessness, insomnia, sometimes convulsions,
stiffness of the neck and strabism show that the nervous
system is being poisoned by toxins, and even collapse may
be reached. The foul and dry tongue, the vomiting and
fetid discharges show the disturbance of the digestive tract.
Very often an eruption appears, as described by Hutinel,
chiefly on the back and buttocks, the front of the thighs and
fore-arms.” The illness may lead to death but is generally
cured by simple purging.
Women in pregnancy and child-birth frequently suffer
much as the result of retention of fæcal matter, and
physicians are familiar with the symptoms, which have
been described as follows by M. Bouchet52:—“After
normal parturition, in the course of which the usual antiseptic
precautions have been fully pursued, and where
delivery has been complete and natural, occasionally the
patient is seized with chill and headache. The breath is
fetid and the tongue foul. The temperature, taken in the
axilla, is nearly 101° Fahr. The abdomen is inflated and
painful in the umbilical region. Palpation in the iliac
fossæ reveals lumps or consolidations along the colon.
Thirst is intense, and there is complete anorexy. On questioning,
it is found that there has not been defæcation for
several days. The treatment consists of purgatives,
enemas, and milk diet. In the next few days the bowels
are emptied freely, the abdominal pain ceases, the temperature
becomes lower, appetite is restored, and the patient
recovers.”
Those who suffer from affections of the heart, liver, or
kidneys are specially susceptible to the evil results of retained
fæcal matter. In such patients an error of diet or
constipation may bring about most serious consequences.
Such facts are well known to physicians, and it has been
established that complete emptying of the lower bowels
leads at once to favourable symptoms. From the other
side, it has been shown by experiment that artificial retention
of the fæces by ligature of the rectum puts the body
in a grave condition.
If we collect our knowledge of all the facts, we cannot
doubt but that the cause of the evil is multiplication of
microbes in the contents of the large intestine. When the
fæcal matter is free from microbes, as is the case with the
meconium of the fœtus or new-born infant, it is not a
source of danger to the organism. The waste of cells and
the secretions which are added to the undigested food
cannot do any harm. Amongst the microbes of the gut,
there are some that are inoffensive, but others are known to
have pernicious properties.
The ill-health which follows retention of fæcal matter is
certainly due to the action of some of the microbes of the
gut. There are difficulties, however, in determining the
precise mode of action of these microbes. It is generally
believed that they form poisonous substances which are
absorbed by the walls of the intestine and so pass into the
system. The phrase auto-intoxication as applied to infants,
women in labour, and patients affected with diseases
of the heart, liver, or kidneys, is based on this interpretation
of the morbid processes involved. Attempts have been
made to isolate and study the poisons in question, but there
are many difficulties in the way. To distinguish between the
actions of the poisons and of the microbes themselves, the
latter have been destroyed by heat or by antiseptics, or been
removed by filtration. Such methods, however, may alter
the poisons and so are inconclusive. MM. Charron and
Le Play53 have tried to obtain exact results by heating the
intestinal microbes to a temperature of about 136° Fahr., a
process which probably does not seriously deteriorate the
microbial poisons. Such material, injected into the veins
of rabbits in large quantities, rapidly produced death, or in
smaller quantities, proportionate ill-health.
Kukula54 has tried to produce this toxic action in animals,
employing microbial secretions obtained from cases of intestinal
obstruction. He succeeded in producing serious
symptoms, such as vomiting and curvature of the neck
and back, in fact, precisely the sequence of events familiar
in cases of obstruction of the bowels or other retentions of
fæcal matter.
Some of the products of the intestinal flora are undoubtedly
toxic, such as the benzol derivatives (phenol,
etc.) ammonium and other salts. Many of these toxins
have been insufficiently studied, but it is well known that
certain of them can be absorbed by the wall of the gut and
act as poisons. A well known case is the toxin of botulism
which was isolated and studied by M. van Ermenghem.55
The poison, the product of a microbe which causes serious
intestinal disturbance, is so fatal that a single drop given
to a rabbit produces death after symptoms similar to those
observed in cases of human beings poisoned by stale food.
Butyric acid and the products of albuminous putrefaction
are amongst the most pernicious of the microbial poisons
produced in the large intestine. It is familiar that digestive
disturbance is frequently associated with discharges of
sulphuretted hydrogen and putrid excreta, and there is no
doubt but that the microbes of putrefaction are the cause of
these symptoms.
It has been assumed for long that the retention of fæcal
matter tends to putrefactive changes in the intestines, and
that the evil consequences of constipation are due to this.
Recently, however, bacteriologists have criticised this
accepted view, on account of the small number of microbes
found in the excreta of constipated persons. Strasburger
was the first to establish the fact, and his associate, Schmidt,
showed that putrefaction did not follow when readily putrescible
substances were infected with material taken from
cases of constipation. However, notwithstanding the
exactness of these facts, I cannot accept the inference which
has been drawn from them. The excreta discharged
naturally in cases of constipation do not give a correct
indication of the conditions inside the gut; whilst such
matter contains few microbes, the substance removed after
injection by an enema is extremely rich in bacteria. Moreover,
analysis of the urine, in cases of constipation, shows
an excess of the sulpho-conjugate ethers which are
known to be products of intestinal putrefaction.
Not only is there auto-intoxication from the microbial
poisons absorbed in cases of constipation, but microbes
themselves may pass through the walls of the intestine and
enter the blood. In the maladies that are the result of
constipation some of the symptoms recall those of direct
infection, and it is highly probable that, if special investigations
were made, microbes of intestinal origin would be
found in the blood of the sick children and the pregnant
or parturient women whose symptoms I have described
above.
The question as to the passage of microbes through the
intestinal walls is one of the most controversial of bacteriological
problems, and there is little agreement in the numerous
publications regarding it. None the less, it is far from
impossible to get a general idea of what goes on in an
intestinal tract richly charged with microbes.
Although the intestinal wall in an intact state offers a
substantial obstacle to the passage of bacteria, it is incontestable
that some of these pass through it into the organs
and the blood. Numerous experiments performed on different
kinds of animals (horses, dogs, rabbits, etc.) show
that some of the microbes taken with food traverse the wall
of the alimentary canal and come to occupy the adjacent
lymphatic glands, the lungs, the spleen and the liver,
whilst they are occasionally found in the blood and lymph.
Discussion has taken place as to whether the passage takes
place when the wall of the gut is absolutely intact or only
when it is injured to however small an extent. It would
be extremely difficult to settle the question definitely, but
it is easy to see that it has little practical bearing. It is
known that the wall of the gut is damaged extremely
easily, so that the bluntest sound can hardly be passed into
the stomach without making a wound through which
microbes can pass into the tissues and blood. In the
ordinary course of life, the delicate wall of the gut must
often undergo slight wounding, and the frequent presence
of microbes in the mesenteric ganglia of healthy animals
shows clearly what takes place.56
It is indubitable, therefore, that the intestinal microbes
or their poisons may reach the system generally and bring
harm to it. I infer from the facts that the more a digestive
tract is charged with microbes, the more it is a source of
harm capable of shortening life.
As the large intestine not only is the part of the digestive
tube most richly charged with microbes, but is relatively
more capacious in mammals than in any other vertebrates,
it is a just inference that the duration of life of mammals
has been notably shortened as the result of chronic poisoning
from an abundant intestinal flora.
Relations between longevity and the intestinal flora—Ruminants—The
Horse—Intestinal flora of birds—Intestinal
flora of cursorial birds—Duration of life in cursorial birds—Flying
mammals—Intestinal flora and longevity of bats—Some
exceptions to the rule—Resistance of the lower vertebrates
to certain intestinal microbes
In the actual state of our knowledge it is impossible to
make a final examination of my hypothesis, as there are
many factors about which we are incompletely informed.
Nevertheless, it is possible to confront the hypothesis with
a large number of accurately established facts.
Although the life of most mammals is relatively short,
there are to be found in the group some which live relatively
long, as well as others whose life is short. The
elephant is an example of the long-lived mammals, whilst
ruminants are short-lived forms. In the last chapter, I
stated that sheep and cattle became senile at an early age,
and did not live long. They are striking exceptions to the
rule according to which the duration of life is in direct relation
with the size and length of the period of growth. The
cow, which is much larger than a woman, and the time of
gestation of which is about the same, or a little longer,
acquires its teeth at four years old, and becomes senile at an
early age; it is quite old at between sixteen and seventeen,
an age when a woman is hardly adult; at the age of thirty,
practically the extreme limit for bovine animals, a woman is
in full vigour.
The precocious old age of ruminants, the constitution of
which is well understood, and which are carefully tended,
coincides with an extraordinary richness of the intestinal
flora. Food remains for a long time in the complicated
stomach of these animals, and afterwards the digested
masses remain still longer in the large intestine. According
to Stohmann and Weiske,57 in the case of sheep it is a
week until the remains of a particular meal have finally
left the body of the animal. The excreta of sheep, normally
solid, do not betray any special putrefaction in the intestine,
but if the body is opened there is abundant evidence
of the process. The intestinal contents are richly charged
with microbes and give off a strong odour of putrefaction.
It is not surprising that under these conditions, the life of
sheep should be short.
Another large herbivorous animal, the horse, also dies
young, after a premature old age. Although it does not
ruminate and possesses a simple stomach, the process of
digestion is slow, and enormous masses of nutritive material
accumulate in the huge large intestine. Ellenberger
and Hofmeister58 have shown that food remains in the
alimentary canal for nearly four days. It remains in the
stomach and the small intestine only 24 hours, but about
three times as long in the large intestine. This is remarkably
different from what happens in the case of birds, in
which there is no stagnation during the passage of food
through the digestive canal.
The structure of birds is adapted for flight, the body
being as light as possible, many of the bones and the
cavities of the body containing air-sacs. The absence of a
bladder and of a true large intestine prevents the accumulation
of excreta, these being ejected almost as rapidly as
they are formed. The process of ejection, which takes
place often in birds, is not so inconvenient as in mammals.
The hind limbs are not used in flight, so that they offer
no obstacle to evacuation. Thus birds may discharge their
droppings while flying.
Such structure and habits make it not surprising that
the alimentary canal of many birds contains only a scanty
intestinal flora. Parrots, for instance, which are remarkably
long-lived birds, harbour very few microbes in the
intestine. The small intestine contains almost none, the
rectum so few that the fæcal matter appears to be formed
of mucus, the waste of the food, and only a very few
microbes. M. Michel Cohendy, who has examined the intestinal
flora at the Pasteur Institute, was unable to isolate
more than five different species of microbes living in the
alimentary canal of parrots.
Even in birds of prey which feed upon putrid flesh, the
number of microbes in the intestine is remarkably limited.
I have investigated the case of ravens which I fed on flesh
which was putrid and swarming with microbes. The droppings
contained very few bacteria, and it was specially
remarkable that the intestines had not the slightest smell of
putrefaction. Although the opened body of a herbivorous
mammal, such as a rabbit, gives off a strong smell of putrefaction,
the body of a raven with the digestive tube exposed
has no unpleasant smell. This absence of putrefaction in
the intestine is probably the reason of the great longevity
of such birds as parrots, ravens, and their allies.
It might be said, however, that the long duration of life
in birds is due to the organisation of these animals, rather
than to the scantiness of their intestinal flora. To meet
this objection, it is necessary to turn to the case of cursorial
birds.
There are some birds incapable of flight, the wings of
which are badly developed, but which have strong limbs,
and can run with great rapidity. Ostriches, cassowaries,
rheas, and tinamous, are well known examples of cursorial
birds. They live on the surface of the ground, and their
habits resemble those of mammals. When they are
attacked by enemies, they escape by running so quickly
that some of them (ostriches and rheas) outstrip even a
horse. However, like mammals, they cannot discharge
their secretions when they are running quickly. Tinamous
(Rhynchotus rufescens), which I have observed in captivity,
however quickly they may be running, stop abruptly to
discharge their excretions. M. Debreuil, at my request,
made observations on this matter, and assured me that the
tinamous and rheas (Rhea americana) in his park always
stood still for this purpose. He has noticed that the droppings,
however abundant, were always deposited in heaps.
With regard to ostriches, M. Rivière, director of the experimental
Gardens at Hamma, Algeria, has been kind enough
to give me the following information. “The discharge of
excreta,” he said in a letter in January, 1901, “is less
frequent than in other birds, but the comparatively small
size of the enclosures here makes it impossible for me to
assert that the animal could discharge its droppings if it
were running for a length of time; a priori I should think
that this did not happen. Normally the bird stands still
for defæcation, the tuft of feathers on the tail is lifted up,
and there is a violent contraction of the abdominal muscles
before the sphincters of the cloaca are suddenly opened to
discharge the excrement with violence.”
I believe that the remarkable development of the large
intestine in these running birds has been acquired to obviate
the danger which is caused by the animal having to stop for
defæcation. Although the huge cæca of these birds have
a digestive function, particularly on plants rich in cellulose,
I cannot think that the cæca of cursorial birds have been
developed for digestion. As a matter of fact, some birds
which are not cursorial live on the same kind of food
(herbage, seeds, and insects) and have much smaller
cæca, the cæca indeed, in some, for instance, the pigeons,
being quite rudimentary.
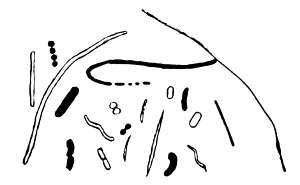
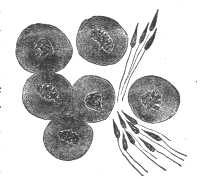
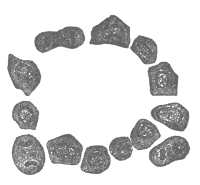
Fig. 14.—Intestinal microbes from the cæca of a Rhea.
It is not surprising that the accumulation of food material
in the large intestine of running birds is associated with
the presence of an extremely rich intestinal flora. Microscopic
examination of the excrement of such birds shows
this at once. Although the intestinal contents and excrement
of many other birds show the presence of very few
microbes, belonging to a small number of species, the same
materials taken from running birds show enormous quantities
of microbes, belonging to a large number of species.
In the cæcum of the rhea (Fig. 14) there are bacterial
threads, spirilla, bacilli, vibrios, and many kinds of cocci.
In the tinamous, the intestinal flora is if possible even
richer. According to the statistical investigations of M.
Michel Cohendy, the quantity of intestinal microbes in
cursorial birds is not less than that found in mammals, even
in man.
If I am correct in the view that I have been explaining,
cursorial birds, on account of their rich intestinal flora,
ought to have a shorter duration of life than that of flying
birds. I will now turn to this side of the question. Amongst
cursorial forms, there are some of the largest living birds,
ostriches being actually the largest living birds, whilst an
extinct running bird, the Aepyornis of Madagascar, was
the largest known bird. According to the rule that large
animals live longer than small animals, ostriches should be
able to reach a great age. The facts, however, are against
this. M. Rivière, who rears ostriches in Algeria, and has
a great experience of them, writes to me as follows: “I
have no confidence in the stories about the longevity of the
ostrich which were told me in the Sahara; they rest on no
facts. My personal observation is not very large, but it is
quite exact. Some of the ostriches which have been hatched
here have lived for 26 years. I do not estimate the duration
of life of this bird at more than 35 years, and only one case
of this age have I seen myself in 20 years. The bird was
a female, a good layer and sitter; she died of old age,
showing all the signs of decrepitude, the skin excoriated
and lumpy, the feathers degenerate and dry. The bird laid
eggs until nearly the end of her life, but at irregular intervals,
and the shells were granular instead of being smooth
and polished.”
In a farm near Nice, where ostriches are reared, there was
recently an old male called “Kruger,” which was supposed
to be 50 years old.59 Countess Stackelberg has been good
enough to try to get information for me about this, and
informs me that although they have not exact knowledge
at the farm, they believe that it must be 50 years old.
M. Rivière thinks this statement very surprising, and has
nothing in his own long experience to confirm it.
The facts which I have been able to get together do not
attribute a long life to other running birds. Gurney mentions
that a cassowary (Casuarius westermanni) lived 26
years in the Zoological Gardens of Rotterdam, and that
three Australian emus (Dromaeus novae-hollandiae) had
lived in the same Gardens for 28, 22, and 20 years. M.
Oustalet (Ornis, 1899, vol. x, p. 62) mentions another
emu of the same species which died in London at the age of
over 23 years. The rhea (Rhea americana), another large
running bird, does not live so long. “Boecking thinks
that its duration of life should be set down at from 14 to 15
years. According to him, many of these birds die of old
age.” (Brehm, Oiseaux, vol. ii, p. 517).
It is striking to compare the short life of cursorial birds,
which nevertheless thrive and reproduce in captivity, with
the remarkable longevity of so many other birds (parrots,
birds of prey) which, although they are much smaller,
have been kept alive for from 80 to 100 years. It would be
difficult to find a more striking argument in favour of the
view that richness of the intestinal flora shortens life. When
birds become adapted to terrestrial life and acquire a huge
large intestine in which microbes can abound, their duration
of life is diminished.
Just as some birds, losing the aerial mode of life, have
come to resemble mammals, so also some mammals have
become flying animals, provided with wings and in some
respects resembling birds. Bats are the most familiar instance.
The large intestine, which is extremely useful to
running animals, not only ceases to be an advantage but is
harmful to flying creatures, insomuch as it increases the
weight of the body uselessly. Bats, accordingly, have no
cæcum whilst the large intestine is changed in structure
and function. Instead of being a capacious tube, serving
as a reservoir for the refuse of the food, the large intestine
of bats has the same diameter as the small intestine. Its
structure is nearly identical. It is provided with glands,
and as I have already mentioned in the last chapter, it
digests the food in the same way as the small intestine.
In fact, the large intestine has become simply a part of the
small intestine, the total length of the gut being reduced.
Bats, therefore, can no longer retain their secretions but
have to empty the intestine almost as often as most birds.
I find that Indian fruit bats (Pteropus medius) discharge
their excreta very often. Microscopic examination shows
that there is an absence of microbes quite unusual in the
case of a mammal. The alimentary canal of bats is nearly
aseptic, containing only a few single bacteria. I have fed
these fruit bats with the same food (carrots) which I have
given to rabbits, guinea pigs, and mice; whilst the bats
accomplished the process of digestion in 1-1/2 hours, and
deposited excreta containing fragments of carrot, the
rodents took very much longer for digestion and large
quantities of waste matter accumulated in the cæca. The
intestinal flora too, although the food in each case was the
same, showed remarkable differences in these animals. It
was almost absent in the bats, whilst in the rabbits, guinea-pigs
and mice it consisted of a mass of microbes of different
species. The excrement of the bats had no unpleasant odour,
and the digestive canal of these bird-like mammals was free
from putrefaction. Fruit bats fed upon fruit discharged
excreta with a pleasant odour of apples and bananas. We
have seen that birds which live a life similar to that of
mammals acquire a rich intestinal flora and do not live so
long as aerial birds. It would be extremely interesting to
ascertain the duration of life of bats, mammals which live
like birds and have a very scanty intestinal flora. I have
been unable to get any exact information as to the duration
of life of the true bats, that is to say, the insectivorous
bats, as all the requests that I have addressed to specialists
have proved fruitless. It appears, however, that it is a
popular belief that bats live long. There is a Flemish
phrase: “as long-lived as a bat,” and a similar phrase is
common in Little Russia.
As for the fruit-eating bats, I have been able to ascertain
that even in captivity, where the conditions are unfavourable
to them, the duration of life is relatively long. I have had
in my own possession a fruit bat (Pteropus medius) which
was bought in Marseilles 14 years ago. It showed no signs
of old age, and the teeth were in perfect condition. It died
of some acute disease accidentally contracted. I know of
another bat of the same species which lived in captivity for
more than 15 years, and I have been informed that60 in the
London Zoological Gardens, a fruit bat has lived for 17
years. If these bats were adult when caught, it would be
necessary to add something to the known figures.
Although I do not know the exact duration of the life of
bats, it is clearly relatively long for mammals no bigger
than guinea-pigs. The difference is remarkable if we compare
it with the life of sheep, dogs and rabbits, mammals
very much larger in size, but possessed of a rich intestinal
flora.
The series of facts that I have been discussing strengthens
my conviction that the intestinal flora is an extremely important
factor in the causation of senility. It must not be
supposed, however, that all the known facts can be explained
equally easily on this hypothesis. The harm done
by microbes cannot always be measured by their abundance
in the alimentary canal. In the first place, it must be
remembered that some microbes are useful; moreover,
microbes, even although their products are very dangerous,
may exist in quantities in an organism, and yet do no harm
if the organism has the power of resisting bacterial poisons.
Thus, for instance, the bacillus of tetanus, which thrives in
the alimentary canal, and which can endanger life if the
wall of the gut is wounded, does not harm a crocodile or a
tortoise, as these animals are extremely resistant to the
poison of tetanus. Dr. Favorsky, by experiments at the
Pasteur Institute, has shown that the poison of botulism
can be absorbed with impunity by some birds, and by tortoises,
although death follows if a very small quantity of it
be introduced into the alimentary canal of a mammal.
The bodies of man and of higher animals are possessed
of a complex mechanism which resists the harmful action of
bacteria and their poisons. The various parts of this
mechanism may act differently, with the result that there is
great variation in the power of resistance. Thus, however
abundant microbes may be in the intestine, they may bring
little harm to an organism that has a high power of destruction
or neutralisation of the toxins, or when these harmful
products are unable to pass through the intestinal wall. It
is in this way that I explain some exceptions to the general
rule, which are exceptions only in appearance. Such a case
is that of the nocturnal birds of prey. Although the diurnal
birds of prey (eagles, vultures, etc.) have very short cæca,
in which the food is never found, owls have very large
cæca, which may be as long as 10 cm. (Eagle-Owl, Bubo
maximus). These long cæca, however, contain debris of
the food only in the enlarged terminal portion, and the
food masses contain a very small number of microbes.
Notwithstanding a great difference in the length of the cæca
between the owls and the eagles, these two groups of birds
do not differ greatly in longevity. But the difference in the
cæca does not imply a corresponding difference in the intestinal
flora which appears to be very scanty in both cases.
It is possible that the elephant is a more real exception to
the rule. Here is a case of a mammal with an enormous
large intestine and a capacious cæcum, and which none the
less is capable of surviving for a century. I have had no
opportunity of investigating the elephant from this point
of view, and have no explanation to suggest.
Monkeys and man differ from most mammals in so far as
they possess a long duration of life, although their large
intestines are very capacious. I have been unable to get
exact information as to the longevity of monkeys, but I
understand that these animals live longer than domesticated
mammals, such as the ox, sheep, dog, and cat. Anthropoid
apes are supposed to be able to reach the age of 50
years. The only other mammal with a longevity similar
to that of the elephant is man.
Longevity of man—Theory of Ebstein on the normal duration
of human life—Instances of human longevity—Circumstances
which may explain the long duration of human life
Man has inherited from his mammalian ancestors his
organisation and qualities. His life is notably shorter
than that of many reptiles, but longer than that of many
birds and most other mammals. None the less he has inherited
a capacious large intestine in which a most abundant
intestinal flora flourishes.
Gestation and the period of growth are long in the human
race, and from the point of view of theoretical considerations,
human longevity should be longer than it generally
is. Haller, a distinguished Swiss physiologist of the 18th
century, thought that man ought to live to 200 years;
Buffon was of the opinion that when a man did not die
from some accident or disease he would reach 90 or 100
years.
According to Flourens, man takes 20 years to grow and
ought to live 5 times 20, that is to say, 100 years.
The actual longevity is much below these figures, which
are based on theory. I have shown, moreover, that even
if the rule based on the theory of growth can be accepted
as generally true, it cannot be applied in every case, as the
factors controlling duration of life are very variable.
Statistics show that the highest human mortality occurs
in the earliest years of life. In the first year after birth
alone, one quarter of the children die. After this period
of maximum mortality, the death-rate slowly falls until
the age of puberty, and then rises again slowly and continuously.
It reaches a second maximum between the ages
of 60 and 75, and then slowly falls again to the extreme
limit of longevity.
Bodio,61 an Italian man of science, holds the view that
the great mortality of infants is a natural adaptation to
prevent too great an increase of the human race. This
view, however, cannot be supported, and rational hygiene
readily brings about a great diminution in the mortality of
children. The cause of mortality is in most cases maladies
of the intestinal canal, produced by erroneous diet, and
with the advance of civilisation, infant mortality has been
very greatly reduced.
I find it impossible to accept the view that the high
mortality between the ages of 70 and 75 indicates a natural
limit of human life. As a result of investigations into
mortality in most of the European countries, Lexis came
to the conclusion that the normal duration of human life
was not more than 75 years. Dr. Ebstein62 accepts this
statistical result and announces that “we now know the
normal limit set by nature to the life of mankind. This
limit is at the age of maximum mortality. If man dies before
then, his death is premature. Everyone does not
reach the normal limit; life ends generally before it, and
only in rare cases after it.”
The fact that many men of from 70 to 75 years old are
well preserved, both physically and intellectually, makes
it impossible to regard that age as the natural limit of
human life. Philosophers such as Plato, poets such as
Goethe and Victor Hugo, artists such as Michael Angelo,
Titian and Franz Hals, produced some of their most
important works when they had passed what Lexis and
Ebstein regard as the limit of life. Moreover, deaths of
people at that age are rarely due to senile debility. In
Paris, for instance, in 1902, of cases of deaths between the
ages of 70 and 74, only 8·5 per cent. were due to old age.63
Infectious diseases, such as pneumonia, tuberculosis, diseases
of the heart and the kidneys, and cerebral
hæmorrhage, caused most of the deaths of these old people.
Such cases of death, however, can often be avoided and
must be regarded as accidental rather than natural.
Confirmation of the view that the natural limit is not at
70 to 75 years is to be found in the fact that so many men
reach a greater age. Centenarians are really not rare. In
France, for instance, nearly one hundred and fifty people
die every year, after having reached the age of 100 or more.
In 1836, in a population of thirty-three millions and a half
(33,540,910), there were 146 centenarians, that is to say, one
in about 220,000 inhabitants. In some other countries,
particularly in Eastern Europe, the number of centenarians
is still greater. In Greece, for instance, there is a centenarian
for each set of 25,641 living persons, that is to say,
nine times as many as in France.64
What age can be reached by the human species? Formerly
it was supposed that individuals might live for
several centuries; to say nothing of Methuselah, whose age
of 969 years, mentioned in the Bible, is the result of a
mistake in calculation, I may mention Nestor, who, according
to Homer, lived for three human ages, that is to say,
300 years, or Dando, the Illyrian, and the King of the
Lacedaemon, who were supposed to have reached ages of five
or six centuries. These ancient records are, of course, quite
incorrect. Much more confidence can be placed in some
facts relating to more modern times, according to which
the extreme old age reached by man was 185 years.
Kentigern, the founder of the Cathedral of Glasgow,
known by the name of St. Mungo, died at the age of 185,
on Jan. 5th, 600.65 Another astonishing case of longevity
is related from Hungary, where an agriculturist, Pierre
Zortay, born in 1539, died in 1724. The Hungarian
records of the 18th century contain other cases of death at
ages between 147 and 172 years.
The case of Drakenberg is still more authentic; he was
born in Norway in 1626 and died in 1772, at the age of
146. He was known as the Old Man of the North. He
had been captured by African pirates and was held by
them for fifteen years, and was engaged as a sailor for
ninety-one years. His romantic history attracted contemporary
attention, and the journals of the time (Gazette de
France, 1764, Gazette d’Utrecht, 1767, etc.)66 contain information
regarding him. The well-known instance of
Thomas Parr appears to rest on good authority. Parr was
a poor Shropshire peasant, who did hard work until he was
130 years old, and who died in London at the age of 152
years and 9 months. The celebrated Harvey examined
the body after death and was unable to discover organic
disease; even the cartilages of the ribs were not ossified and
were elastic as in a young man. The brain, however, was
hard and resisting to the touch, as its blood-vessels were
thickened and dry. Parr was buried in Westminster
Abbey.67
It appears, then, that human beings may reach the age
of 150, but such cases are certainly extremely rare, and
are not known from the records of the last two centuries.
I cannot accept without a good deal of reserve the statements
as to two persons who died in the beginning of
the 19th century at the ages of 142 and 145. On the other
hand, cases of duration of life from 100 to 120 years are
not very rare.
Extreme longevity is not limited to the white races.
According to Prichard,68 negroes have lived respectively
to 115, 160, and 180 years. In the course of the 19th
century there have been observed, in Senegal, eight negroes
ranging from 100 to 121 years old. M. Chemin69 saw
himself in 1898 at Foundiougne an old man, whom the
natives stated to be 108 years of age; although he was
in good health, he had been blind for several years. The
same author, on the authority of the New York Herald
of June 13th, 1895, mentions the case of a coloured woman
in North Carolina, who was more than 140 years old, and
of a man 125 years old.
Women more frequently become centenarians than
men, although the difference is not very great. For instance,
in Greece, in 1885, in a population of nearly two
millions (1,947,760), there were 278 persons aged from
95 to 110 years, of whom 133 were male and 145 female.
In the seven years, from 1833 to 1839 inclusive, according
to Chemin, there were in Paris twenty-six men over the age
of 95, and forty-five women. Such facts, and many others,
support the general proposition that male mortality is
always greater than that of the other sex.
In most cases centenarians are notably healthy and of
strong constitution. There are instances, however, of
abnormal people having reached a great age. A woman,
called Nicoline Marc, died in 1760, at the age of 110.
Since she was two years old, her left arm was crippled.
Her hand was bent under the arm like a hook. She was
a hunch-back, and so bent that she appeared to be no
more than four feet high. A Scotch woman, Elspeth
Wilson, died at the age of 115 years. She was quite a
dwarf, being only a little over two feet high. On the other
hand, although they usually have a very short life, giants
have been known to reach the age of 100.
Haller, in the eighteenth century, remarked that centenarians
often occurred in the same family, as if longevity
were a hereditary quality. It is certainly the case that the
descendants of centenarians frequently reach extreme age.
Thomas Parr, for instance, left a son who died in 1761,
at the age of 127 years, having retained his mental faculties
until death. In M. Chemin’s list of centenarians,
there are eighteen cases of extreme old age having been
reached by their relations. As all innate characters can be
transmitted, the influence of heredity and longevity must
be admitted. At the same time, it is necessary to remember
the important influence of the similarity of conditions
in the case of parents and children. Many cases of tuberculosis
and leprosy, which used to be assigned to heredity,
are now known to be due to infection in the same conditions
of life, and some of the examples of the attaining
of a great age by more than one member of a family may
be explained by the influence of surrounding circumstances.
Very frequently the husband and wife, although
not related by blood, both attain extremely advanced age.
I found 22 cases of this kind in M. Chemin’s list; I will
give a few of them. A widow, Anne Barak, died at the
age of 123, in Moravia; her husband died at the age of
118. In 1896, there was alive in Constantinople, M.
Christaki, a retired army doctor of the age of 110; his
wife was 95 years old. In 1886, M. et Mme. Gallot, aged
respectively 105 years and 4 months, and 105 years and
one month, died within two days of each other at Vaugirard,
54, Rue Cambronne. Lejoncourt mentions a South
American of 143 years old, whose wife had lived to the
age of 117.
It is worth enquiring if there be any relation between
longevity and locality. There are some countries in which
very many of the natives reach old age. It appears that
Eastern Europe (Balkan States, and Russia), although
its civilisation is not high, contains many more centenarians
than Western Europe. I have already mentioned
that Dr. Ornstein had shown the existence of many extremely
old people in Greece. M. Chemin states that
in Servia, Bulgaria and Roumania there were more than
5,000 centenarians (5,545) living in 1896. “Although
these figures appear to be exaggerated,” wrote M. Chemin,
“it is undoubtedly the case that the pure and keen air of
the Balkans, and the pastoral or agricultural life of the
natives, predisposes to old age.” The same author mentions
several localities in France, notable for the numbers
of very old people. In 1898 in the commune of Sournia
(Pyrénées-Orientales) the total population was 600,
amongst which there was one woman of 95 years, a man
of 94, a woman of 89, two men of 85, two of 84, and two of
83, three women of 82, and two men of 80. At St. Blimont
in the Department of the Somme, amongst the 400 inhabitants
alive in 1897, there were six men between the ages of
85 and 93 years and one woman in her 101st year.
It cannot be accepted that it is the keen air which
lengthens the life, because Switzerland, a mountainous
country, is notable for the rarity of centenarians. It is
more likely that some circumstance in the mode of living
influences longevity.
It has been noticed that most centenarians have been
people who were poor, or in humble circumstances, and
whose life has been extremely simple. There are instances
of rich centenarians, such as Sir Moses Montefiore who
died at the age of 101, but such are extremely rare. It may
well be said that great riches do not bring a very long life.
Poverty generally brings with it sobriety, especially in
old age, and it has been often said that most centenarians
have lived an extremely sober life. They have not all
followed the example of the celebrated Cornaro, who
brought himself to subsist on a daily diet of no more
than twelve ounces of solid food, and fourteen ounces of
wine, and who, although his constitution was weak, lived
for about a century. He has left extremely interesting
Memoirs, and retained his intelligence until his death on
the 26th April, 1566 (Lejoncourt, p. 146).
In M. Chemin’s list I have counted twenty-six centenarians,
distinguished by their frugal life. Most of them
did not drink wine, and many of them limited themselves
to bread, milk and vegetables.
Sobriety is certainly favourable to long life, but it is
not necessary, because quite a number of centenarians have
drunk freely. Several of those who are catalogued by
Chemin, drank wine and spirits even to excess. Catherine
Reymond, for instance, who died in 1758 at the age of 107
years, drank much wine, and Politiman, a surgeon who
lived from 1685 to 1825, was in the habit, from his twenty-fifth
year onwards, of getting drunk every night, after
having attended to his practice all day. Gascogne, a butcher
of Trie (Hautes-Pyrénées), died in 1767 at the age of 120,
and had been accustomed to get drunk twice a week. A
most curious example is that of the Irish land-owner
Brawn, who lived to the age of 120, and who had an inscription
put upon his tombstone that he was always
drunk, and when in that condition was so terrible that
even death had been afraid of him. Some districts, even,
are distinguished at once for the longevity of their inhabitants
and for the large local consumption of alcohol.
In 1897, village of Chailly in the Côte-d’Or had no
less than twenty octogenarians amongst 523 inhabitants.
This village is one of the localities in France where most
alcohol is consumed, and the old people are very far from
being distinguished from their younger fellows by any
special sobriety.
In some cases centenarians have been much addicted to
the drinking of coffee. The reader will recall Voltaire’s
reply when his doctor described the grave harm that
comes from abuse of coffee which acts as a real poison.
“Well,” said Voltaire, “I have been poisoning myself for
nearly 80 years.” There are centenarians who have lived
longer than Voltaire, and have drunk still more coffee.
Elisabeth Durieux, a native of Savoy, reached the age of
114. Her principal food was coffee, of which she took daily
as many as forty small cups. She was jovial and a boon
table companion, and used black coffee in quantities that
would have surprised an Arab. Her coffee-pot was always
on the fire, like the tea-pot in an English cottage (Lejoncourt,
p. 84; Chemin, p. 147).
It has been noticed that many centenarians do not smoke,
but this like all other traits is not universal. M. Ross,
who gained a prize for longevity in 1896 at the age of 102,
was an inveterate smoker. In 1897, a widow named
Lazennec, died at La Carrière, in Kérinou, Finistère, at
the age of 104. She lived in a hovel on charity, and she
had smoked a pipe ever since she was quite young.
It is plain that any factor to which long duration of life
has been attributed disappears when many cases are
examined. Naturally a sound constitution and a simple
and sober life are favourable to longevity, but apart from
these, there is something unknown which tends to long
life. The celebrated physiologist of Bonn, Pflüger,70 came
to the conclusion that the chief condition of longevity is
something “intrinsic in the constitution,” something which
cannot be defined exactly, and which must be set down to
inheritance.
In the present state of knowledge, we cannot denote the
chief cause of human longevity, but the proper course
will be to seek it out as we would seek out that of animal
longevity. As human longevity is often local in its character,
and is exhibited by married people who have nothing in
common except their mode of life, we may enquire into the
intestinal flora and the mechanism by which the organism
resists its harmful effect as factors which influence the
duration of life. It is reasonable to suppose that in persons
living in the same district or under the same roof, the intestinal
flora may be similar. The problem can be settled
only by a series of laborious researches which have yet to
be made. At present I can do no more than bring together
a large number of facts regarding the duration of life in
man and in animals, with the hope of suggesting the lines
for future investigation.