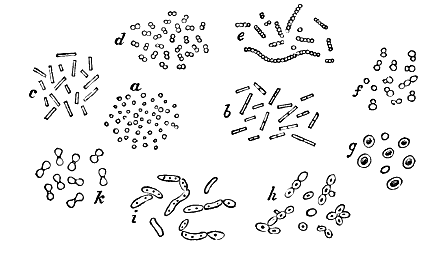
The mode of origin of Bacteria, and, to a less extent,
of Torulæ, has been much discussed of late, and many
different views have been advocated on this subject by
successive writers.
It is of much importance to bear in mind when such
views are under consideration, that a short time since
nothing was positively known concerning the life-history
of these organisms. However strongly, therefore,
certain persons are inclined to rely upon the
analogy which is supposed to obtain between these
doubtful cases, and the multitudes of known cases—in
which it can be shown that organisms are the
offspring of pre-existing organisms—it must always
be borne in mind that in many of the doubtful cases,
where the simplest organisms are concerned, there is
also an analogical argument of almost equal weight
adducible in favour of their de novo origination—after
a fashion, and under the influence of laws
similar to those by which crystals arise. To rely
too exclusively upon an argument from analogy is
always perilous: it is more than usually so, however,
in a case like this, where what is practically
an opposing analogy may be deemed to speak just
as authoritatively in an opposite direction.
There is one consideration, moreover, which deserves
to be pointed out here, and which does not seem to
have occurred to most of those who so firmly pin their
faith to the truth of the motto “omne vivum ex vivo.”
The every-day experience of mankind, supplemented
by the ordinary observations of skilled naturalists, does
pretty fairly entitle us to arrive at a wide generalization,
to the effect that some representatives of every
kind of organism are capable of reproducing similar
organisms. But, whilst this is all that the actual
every-day experience of mankind warrants being said,
and whilst there is in reality the widest possible gulf
between such a generalization and that which is expressed
by the motto “omne vivum ex vivo,” the
latter formula has of late been spoken of as though
it were the one which was in accordance with the daily
experience of mankind, rather than the other, which
gives expression to a generalization of a much narrower
description. This experience, in reality, affords
no evidence which could entitle us to place implicit
belief in the formula “omne vivum ex vivo.”
Whilst we do know something about the ability
which most organisms possess of reproducing similar
organisms, we cannot possibly say, from direct observation,
that every organism which exists has had
a similar mode of origin, because the cases in which
organisms may have originated de novo are the very
cases in which their mode of origin must elude our
actual observation. Such a statement, too, would be
all the more dangerous, in the face of the other
analogy, when it can actually be shown that some
organisms do make their appearance in fluids after
precisely the same fashion as crystals.
Although, therefore, there is a contradiction between
the unwarrantable and ill-begotten formula, “omne
vivum ex vivo,” and the doctrines of what has been
called “Spontaneous Generation”; there is no contradiction
whatever between such doctrines and the
only generalization which we are really warranted
in arriving at, to the effect that some representatives
of every kind of organism are capable of reproducing
similar organisms.
Bacteria, Torulæ, or other living things which may
have been evolved de novo, when so evolved, multiply
and reproduce just as freely as organisms that have
been derived from parents.
The views as to the origin of Bacteria and Torulæ
which are most worthy of attention, may be thus
enumerated:—
a. That they are independent organisms derived by
fission or gemmation from pre-existing Bacteria and
Torulæ.
b. That they represent subordinate stages in the
life-history of other organisms (fungi), from some
portion of which they have derived their origin, and
into which they again tend to develop.
c. That they may have a heterogeneous mode of
origin, owing to the more complete individualization
of minute particles of living matter entering into the
composition of higher organisms, both animal and
vegetal.
d. That they may arise de novo in certain fluids
containing organic matter, independently of pre-existing
living things (Archebiosis).
I shall make some remarks concerning each of these
views, though the evidence I have to adduce mainly
concerns the possibility of the origin of Bacteria and
Torulæ in the way last alluded to, viz., by Archebiosis.
The third mode of origin is what is called Heterogenesis;
whilst the first and second modes are
the representatives of more familiar processes, included
under the head of Homogenesis. Thus, in
accordance with the first view, Bacteria may be
regarded as low organisms having a distinct individuality
of their own and multiplying by a process
of fission—thus affording instances of what I propose
to term direct Homogenesis. Whilst, in accordance
with the second view, Bacteria are supposed to represent
merely one stage in the life-history of higher
organisms, which are therefore reproduced by an indirect
or cyclical process of Homogenesis.
The possible modes of origin of Bacteria and
Torulæ may, therefore, be tabulated as follows:—
Modes of origin
of Bacteria and
Torulæ. |  | 1. Homogenesis. |  | a. Direct. |
| b. Indirect. |
| 2. Heterogenesis. |
| 3. Archebiosis. |
Bacteria and Torulæ being already in existence,
they may, undoubtedly, reproduce organisms similar
to themselves by processes of fission and gemmation—in
the same way that other low protistic
organisms propagate their kind. Although so many
reasons rendered this view probable, it was some
time before I was able actually to confirm it by
personal observations in the case of Bacteria. In the
ordinary microscopical examination of portions of an
infusion containing these organisms, an observer may
watch for hours and never see a single instance of
such fission occurring. His attention is apt to be distracted
by the number of organisms which are constantly
flitting before his view, and he is, moreover,
perhaps apt to pay particular attention to those which
seem by their movements to be most obviously alive.
I have observed the process most plainly when a
few Bacteria have been enclosed in a single drop of
fluid, pressed into a very thin stratum, in a “live-box”
kept at a temperature of about 90° Fahr. by resting
on one of Stricker’s warm-water chambers placed on
the stage of the microscope. Under these conditions,
I have seen a Bacterium of moderate size divide into
two, and each of these into two others somewhat
smaller, in the course of fifteen minutes.
It is still more worthy of remark, that in all cases
(so far as I have been able to observe), this, the most
certain sign of vitality which such organisms are
capable of manifesting, is shown by those which,
from their stillness, might be considered dead. The
Bacteria which are about to divide are generally either
motionless,1 or merely present slight oscillating movements.
The separation is quickly brought about at
the joint, so that the original organism divides into
two equal portions; and these, lying close together,
soon develop a new construction as they grow, through
which a further division may occur.
That the Bacteria which reproduce should be in a
comparatively quiescent condition, seems not difficult
to understand. Such rudimentary organisms do not appear
to possess cilia or other locomotory appendages:
their movements are, therefore, in all probability dependent
upon the mere molecular changes which are
taking place within them, and upon which their life
and nutrition depend. The process of fission must,
however, be considered as the result of a new effort at
equilibrium, which has, perhaps, been necessitated
by molecular changes that have occurred during a
preceding period of growth. The living matter which
is no longer able to exist round a single centre,
re-arranges itself around two centres,—as a result of
which, fission occurs. It seems only natural, therefore,
that whilst this active work of molecular re-arrangement
is going on, those other molecular
movements which occasion the actual locomotion
of the organism from place to place, should be more
or less interfered with.
This is the one and only mode of multiplication of
Bacteria and of Torulæ which is actually known to
occur; and such a limitation is in accordance with the
more general fact, that processes of fission or gemmation
are the only means of reproduction that are known
to occur in the lower kinds of organisms, belonging to
the PROTISTIC kingdom.
However well this process of fission may have
been established, as a frequent mode of reproduction
of Bacteria, such a fact does not lend any support to
the notion that these are necessarily distinct and
independent organisms. Torulæ (of which beer-yeast
is the most familiar example) may similarly undergo
this process of mere vegetative repetition to an
indefinite extent, whilst only some of the products
develop into fungi. The gonidia of lichens may also
reproduce indefinitely in this fashion, and only some
of the products of multiplication may go on to the
production of lichens similar to that from which the
gonidia had been derived.
It is a fact, however, admitted by many, and
which any patient microscopist is capable of verifying
for himself, that some Bacteria do develop into
Leptothrix filaments, and that these are capable of
passing into a dissepimented mycelial structure of
larger size and undoubtedly fungus nature—from
which fructification of various kinds may be produced.
Some Bacteria may therefore develop into some
fungi, just as certainly as some Torulæ may develop
into other fungi, or, just as surely as some multiplying
gonidia may develop into lichens.
In order to prove, however, that the Bacteria which
happen to go through this development into Leptothrix
and thence into fungi, are strictly to be
considered as necessary links in the life-history of
fungi, it would be essential for the person holding
such views, to show that Bacteria could not arise
independently—or at least that no independently
evolved Bacteria could develop through Leptothrix-forms
into a fungus. And, similarly, for the other
kinds of organisms: in order to establish that the
Torula cell is a necessary link in the life-history of
certain fungi, or the gonidial cell a necessary link in
the life-history of lichens, it would be necessary to
show that Torulæ or gonidial cells could not originate
de novo—that no independently evolved Torula or gonidial
cell could develop into a fungus or a lichen.
An easier position to establish would be, that the
Bacterium or the Torula were occasionally links in the
life-history of fungi, or that the gonidial cell was an
occasional link in the life-history of a lichen. This
doctrine would leave the other more difficult problems,—as
to the possible existence of supplementary
modes of origin for such organisms by Heterogenesis
or by Archebiosis—perfectly open questions.
To establish the position that Bacteria are occasional
links in the life-history of fungi, it would be
only necessary to show that some of the Bacteria
which develop into fungi through Leptothrix have
derived their origin from pre-existing fungi. This is
the view which Hallier2 has endeavoured to establish;
it is also the doctrine of M. Polotebnow,3 and one,
moreover, to which Professor Huxley4 inclines. Even
this mode of origin for Bacteria, however, has not been
so decisively established as might be desired. With
regard to Torulæ, we do possess sufficient evidence
tending to show that some of them may arise from
pre-existing fungi, and we are equally certain that
some gonidial cells are thrown off from lichens. The
analogical evidence is, therefore, in favour of the view
that minute particles which are budded off from the
mycelium of certain fungi, may subsequently lead an
independent existence, and multiply in the form of
Bacteria—although many of the cases in which such
buds seem to be given off, may be merely cases in
which co-existing Bacteria have become adherent to
fungus filaments or to Torulæ.5
But, with reference to these supposed cases of budding,
and also to those others in which the contents of
a spore or sporangium break up into what Professor
Hallier calls “micrococci” (which are generally incipient
Bacteria), it would be difficult for us to decide
whether such processes are normal or abnormal.
When we have to do with such organisms, in fact,
there may be the nicest transitions between what is
called Homogenesis, and what, when occurring in
other organisms, we term Heterogenesis. It may be
that the production of such “micrococci” from the
spore or sporangium of the fungus is not an invariable
incident in the life-history of the species, but rather an
occasional result of the influence of unusual conditions,
or of failing vigour on the part of the organism. In
this latter case we should have to do with a process of
Heterogenesis; although, as I have just stated, in
respect to such low and changeable organisms,
scarcely any distinct line of demarcation can be drawn
between Homogenesis and Heterogenesis.
The evidence seems, therefore, against the notion
that Bacteria or Torulæ are ordinary, independent
living things, which merely reproduce their like.
That some Bacteria are produced from pre-existing
Bacteria, just as some Torulæ are derived from pre-existing
Torulæ, may, it is true, be considered as
settled. But, so far as we have yet considered the
subject, there may be just as good evidence to show
that Bacteria and Torulæ are capable of arising de
novo, as there is that some of them are capable of
developing into fungi.
If this were the case, such types could only be
regarded as the most common forms assumed by
new-born specks of living matter; and, by reason of
their origin—which would entail an absence of all
hereditary predisposition—they might be supposed to
be capable of assuming higher developmental forms.
Now, as a matter of fact, worthy of arresting our
attention, we do find that some Bacteria are capable of
growing into Leptothrix, whilst this is able to develop
continuously into a fungus; just as we also know
that some Torulæ are capable of growing into other
fungi.
Should it be established, therefore, that Bacteria
and Torulæ are capable of arising de novo, the facts
concerning their mutability are harmonious enough
with theoretical indications.
But, as I have before indicated, although it is quite
true that some Bacteria develop into fungi, such forms
may constitute no necessary links in the life-history of
other fungi. I have suggested that in those (occasional)
cases in which they do occur as links in the life-history
of fungi, there is room for doubt whether these
Bacteria are to be considered as normal products, or
as abnormal results (heterogeneous offcasts), brought
about by some unusual conditions acting upon the
parent fungus. That is to say, we may be doubtful
whether in such a case their origin ought to be considered
Homogenetic or Heterogenetic. It may be
that many of the lower fungi are such changeable
organisms, and so prone to respond to the various
“conditions” acting upon them (which would be almost
certainly the case if they had been developed from a
Bacterium in two or three days—the Bacterium itself
having been evolved de novo) that no very valid distinction
can here be drawn between Homogenesis and
Heterogenesis. Our whole point of view, in fact, concerning
such fungi as are seen to develop through
Leptothrix forms from Bacteria must be entirely
altered, if it is once conceded that Bacteria may arise
de novo. Such simple Mucedineæ would then have to
be regarded as mere upstart organisms only a few
removes from dead matter, and—in view of the greater
molecular mobility of living matter—capable of being
modified in shape and form even more than the most
changeable crystals under the influence of altering
“conditions.” We should have no longer to do with
the members of a stable species, which had been reproducing
its like through countless geologic ages anterior
to the advent of man upon the earth. Indeed, in
order to reconcile such a possibility with the seemingly
contradictory fact of the known extreme changeability
of these lower forms of life, we hear only vague
hints thrown out about our imperfect knowledge of
the “limits within which species may vary.” As if, in
the face of what we do know concerning hereditary
transmission, this changeability did not make it
almost impossible to conceive that there should have
been an unbroken series of such organisms since that
remote epoch of the earth’s history, when the first
organisms of the kind made their appearance. It does
not seem to me that the presumed permanence of a
very changeable organism is consistent with, or rendered
more explicable by, the supposition that some
representatives of the species have constantly been
undergoing progressive modifications which have been
successively perpetuated by inheritance, in the shape
of distinct specific forms. Why should some be presumed
to have undergone so much change, whilst
others (presenting an equal and an extreme degree of
modifiability, even to the present day) are supposed
to have preserved the same specific form through a
countless series of changing influences?
It has been long known that Bacteria and Torulæ
are frequently to be found within vegetable cells,
taken even from the central parts of plants, whenever
these are in a sickly condition or are actually dying.
They are apt to exist also within epithelial cells taken
from the inside of the mouth; and the frequency and
abundance with which such organisms are met with in
these cells, is almost in direct proportion to the malnutrition
and lack of vital power in the individual who
is the subject of observation. Then, again, in persons
who have died of adynamic diseases, in the course of
twenty-four or thirty-six hours (during warm weather)
Bacteria may be found in abundance within the blood-vessels
of the brain and of other parts, although no
such Bacteria were recognizable in the blood of the
individual during life.
In these cases we must, in order to account for the
presence of the Bacteria and Torulæ, either suppose
that such organisms, in an embryonic state, are almost
universally disseminated throughout the various textures
of higher organisms, both animal and vegetal
(though they are only able to develop and manifest
themselves when the higher organisms, or the parts of
them in which the Bacteria or Torulæ are met with,
are on the eve of death), or else we must imagine
that when the vital activity of any organism, whether
simple or complex, is on the wane, its constituent
particles (being still portions of living matter) are
capable of individualizing themselves, and of growing
into the low organisms in question. Just as the life
of one of the cells of a higher organism may continue
for some time after the death of the organism itself,
so, in accordance with this latter view, may one of the
particles of such a cell be supposed to continue to
live after even cell-life is impossible.
Now, to many persons, the latter seems to be a
much simpler hypothesis than the former, and one,
moreover, which is more in accordance with known
facts. People’s views, however, on this subject are
likely to be much influenced by their notions as to
the possibility of Bacteria arising by a process of
Archebiosis. Although some may be inclined to accept
the doctrine of Heterogenesis, the same persons,
being “vitalists,” may not readily believe in the
doctrine of Archebiosis, because this implies the
vivification of dead matter—the conversion of not-living
elements into a living combination. Those,
however, who do believe in Archebiosis will—if the
necessary evidence be forthcoming—all the more
readily yield their assent to the doctrine of Heterogenesis,
because it is a much less novel thing
to have to believe in the mere transformation of
living matter, than in the possibility of its origin de
novo.
Evidence of a tolerably satisfactory nature, however,
is forthcoming, which may speak independently
in favour of the doctrine of Heterogenesis.
It has been affirmed by Crivelli and Maggi6 that
they have actually seen the particles within granular
epithelial cells (taken from the back of the tongue of
a patient suffering from diabetes) grow and elongate,
so as to give rise to Bacteria, or fuse in longitudinal
series, so as to form a Vibrio.7 And, moreover, as
I have myself ascertained, if one takes healthy-looking
epithelial scales scraped from the inside of
the mouth, which appear to contain nothing but the
finest granules, and places them with a little saliva
in a “live-box” (and this within a damp chamber kept
at a temperature of about 90° Fahr.), in the course
of from 5 to 10 hours, the cells may be found to be
studded throughout with motionless Bacteria. Of
course it may be said that the granules originally
seen in the cells were offcasts from pre-existing
Bacteria8 which had gained access to the cell.
And although, to many, this may seem an extremely
improbable supposition, it is, nevertheless, one which
it would be very difficult to disprove. The improbability
of the notion is increased, moreover,
when we find that Bacteria, and even Torulæ, will
develop just as freely within closed cells taken from
the very centre of a vegetable tuber, as they will in
the midst of the more solid epithelial cell from the
inside of the mouth. If it be urged that in this latter
situation, there is the greatest chance of the cells
being brought into contact with Bacteria, and that
it must be considered possible for imaginary minute
offcasts from these Bacteria to make their own way
into the substance of the epithelial cell, I am quite
willing to grant the desirability of taking such possibilities
into consideration. But, at the same time,
it seems all the less likely that the actual occurrence
of the Bacteria is explicable on these grounds, because
we find them developing just as freely within
the cells freshly cut from the centre of a tuberous
root, or we may find them already developed within
these cells, if the root has begun to decay. To suppose
that actual germs of Bacteria and of Torulæ are
uniformly distributed throughout the tissues of higher
organisms, is to harbour a hypothesis which would
appear to many to be devoid of all probability—more
especially when the heterogenetic mode of origin of
larger and higher organisms is a matter of absolute
certainty.
The evidence on this part of the subject is, I think,
sharply defined and conclusive. Simple experiments
can be had recourse to, which are not admissible in
the discussion of the question as to the origin of Bacteria
and Torulæ by Heterogenesis. There, we wish to
establish the fact that living matter is capable of undergoing
a certain metamorphosis, and consequently,
we must deal with living matter. Here, however, with
the view of establishing the fact that living matter
can arise de novo, if we are able, shortly after beginning
our experiment, to arrive at a reasonable and well-based
assurance that no living thing exists in the hermetically
sealed experimental vessel—if the measures
that we have adopted fully entitle us to believe that
all living things which may have pre-existed therein
have been killed—we may feel pretty sure that any
living organisms which are subsequently found, when
the vessel is broken, must have originated from some
re-arrangements which had taken place amongst the
not-living constituents of the experimental solutions,
whereby life-initiating combinations had been formed.
The possibility of the de novo origination of Bacteria,
Torulæ, and other such organisms, is one which is intimately
associated with the doctrine as to the cause of
fermentation and putrefaction. With regard to the
almost invariable association of such organisms with
some of these processes, almost all are agreed. There
is, moreover, a very frequent association of particular
kinds of organisms with particular kinds of fermentation.
Hence the assumption is an easy and a natural
one to many persons, that the organisms which are
invariably met with in some cases are the causes of
these fermentations,9 although it is quite obvious that
the facts on which this view is based, are equally explicable
on the supposition that the organisms are
concomitant results or products (due to new chemical
combinations) of the fermentative changes. In the one
case the fermentative changes are believed to be initiated
by the influence of living organisms; and those
who regard living things as the only true ferments,
for the most part also believe that living things are
incapable of arising de novo. They think that those
organisms which serve to initiate the changes in question,
have been derived from a multitudinous army
of omnipresent atmospheric germs, which are always
ready, in number and kind suitable for every emergency.
This is the doctrine of M. Pasteur and others.
On the other hand, fermentations and putrefactions
may be regarded as sets of chemical changes, which
are apt to occur in organic and other complex substances—these
changes being due either to the intrinsic
instability of the body which manifests them, or to
molecular movements communicated to it by a still
more unstable body. Baron Liebig says:—“Many
organic compounds are known, which undergo, in presence
of water, alteration and metamorphosis, having a
certain duration, and ultimately terminating in putrefaction;
while other organic substances that are not
liable to such alteration by themselves, nevertheless,
suffer a similar displacement or separation of their molecules,
when brought into contact with the ferments.”
Each substance belonging to the first class, would
be at the same time, therefore, both ferment and fermentable
substance; whilst a small portion of such
substance, when brought into contact with a less unstable
substance, might induce such molecular movements
as to make it undergo a process of fermentation.
With regard to the cause of such induced fermentative
changes, Gerhardt10 says, in explaining Liebig’s views:—“Every
substance which decomposes or enters into
combination is in a state of movement, its molecules
being agitated; but since friction, shock, mechanical
agitation, suffice to provoke the decomposition of many
substances (chlorous acid, chloride of nitrogen, fulminating
silver), there is all the more reason why a
chemical decomposition in which the molecular agitation
is more complete, should produce similar effects
upon certain substances. In addition, bodies are
known which when alone are not decomposed by certain
agents, but which are attacked, when they exist
in contact with other bodies incapable of resisting
the influence of these agents. Thus platinum alone
does not dissolve in nitric acid, but when allied with
silver, it is easily dissolved; pure copper is not dissolved
by sulphuric acid, but it does dissolve in this
when it is allied with zinc, &c. According to M. Liebig
it is the same with ferments and fermentable
substances; sugar, which does not change when it is
quite alone, changes—that is to say ferments—when
it is in contact with a nitrogenous substance undergoing
change, that is, with a ferment.”
Thus, in accordance with this latter view, living
ferments are not needed—mere dead, organic or nitrogenous
matter suffices to initiate the processes in
question.11 Those who hold this opinion may or may
not believe that organisms are capable of arising
de novo;12 though there can be little doubt that a
belief in the truth of such a doctrine does, almost inevitably,
entail a belief in the de novo origination of living
things. No one who has looked into the evidence,
doubts the fact of the association between some of
these processes and the presence of organisms; the only
question is, as to the relation in which they stand to
one another. If organisms are not the causes of those
fermentative changes with which they are invariably
associated, then they are, in all probability, the results
of such changes; and they must certainly have been
produced de novo if it can be shown that fermentation
or putrefaction may take place under the influence of
conditions which make it certain that pre-existing
living organisms could have had nothing to do with
the process.
Now, in order to lend some air of probability to
the former hypothesis, concerning the necessity for the
existence of living ferments, it was incumbent upon its
supporters to endeavour to show that the air did contain
such a multitude of “germs,” or living things, as
were demanded by the requirements of their theory.
Spallanzani and Bonnet had, as far as the imagination
was concerned, done all that was necessary. They
had proclaimed the universal diffusion of “germs” of
all kinds of organisms throughout the atmosphere—which
were ready to develop, whenever suitable
conditions presented themselves. So far, however,
this was but another hypothesis. To establish the
doctrine that fermentation cannot take place without
the agency of living ferments, we cannot receive hypotheses
in evidence: facts are needed. These, no one
attempted to supply in an adequate manner13 anterior
to the investigations of M. Pasteur. Speaking
of his researches, even M. Milne-Edwards says,14 “Previous
to this time, the existence of reproductive particles,
or infusorial germs in the atmosphere was
nothing more than a plausible hypothesis, put forward
in order to explain the origin of such creatures in a
manner conformable with the general laws of reproduction;
but it was only a mere supposition, and no
one had been able actually to see or to handle these
reproductive corpuscles.”
We have to look, therefore, to M. Pasteur’s investigations,
and to others which may have been since
conducted, for all the scientific evidence in support of
what has been called the “Panspermic hypothesis.”
By an ingenious method of filtration, which is fully
described in his memoir,15 M. Pasteur separated from
the air that passed through his apparatus the solid
particles which it contained. This search convinced
him that there were, as he says, “constantly in ordinary
air a variable number of corpuscles whose form
and structure declare them to be organized.” Some
of these, he thinks, resemble the spores of fungi, and
others the ova of ciliated infusoria, though he adds:—“But
as to affirming that this is a spore, much less the
spore of any definite species, and that one is an
egg, and belonging to such an infusorium, I believe
that this is not possible.” He limits himself, in fact,
to the statements, that the corpuscles which he found,
were (in his opinion) evidently organized; that they
resembled in form and appearance the germs of the
lower kinds of organisms; and that, from their
variety in size, they probably belonged to many
different sorts of living things. Even here, therefore,
we have to do with the impressions of M. Pasteur,
rather than with verified statements. All that has
been established by his direct investigation as to the
nature of the solid bodies contained in the atmosphere
is this: that the air contains a number of round or
ovoidal corpuscles, often quite structureless, which
he could not distinguish from the spores of fungi16—some
of which, being about the right size, were round
or ovoidal, and structureless. In addition, however,
it has been shown that the air contains other rounded
corpuscles which are similarly structureless, though
composed of silica or starch. It may therefore be
asked, in the first place, whether the conclusion is
a sufficiently safe one that many of the corpuscles
found by M. Pasteur were spores of fungi; and in the
next place, supposing this to have been established,
whether such spores were living or dead. These
questions would have been answered satisfactorily if
M. Pasteur could state that he had actually watched
the development of such corpuscles, in some suitable
apparatus, into distinct organisms. But any such
development, he distinctly states, he never witnessed.
He says17:—“What would have been the better and
more direct course would have been to follow the
development of these germs with the microscope.
Such was my intention; but the apparatus which I
had devised for this purpose not having been delivered
to me at a convenient time, I was diverted from this
investigation by other work.” The evidence which
he does adduce, in subsequent portions of his memoir,
in order to prove that some of these corpuscles were
really “fertile germs,” is almost valueless, because all
the facts are open to another interpretation, which is
just as much, nay, even more, in accordance with Baron
Liebig’s than with his own doctrine of fermentation.
But another most important consideration presents
itself. M. Pasteur’s researches as to the nature of
the dust contained in the atmosphere enable him to
say nothing concerning the presence of Bacteria,
although he himself admits that these are generally
the first organisms which display themselves in fermentations
or putrefactions, and that in a very large
majority of the cases in which fermentation occurs
in closed vessels they are the only organisms which
make their appearance.18 And yet, notwithstanding
these facts, M. Pasteur says, in reference to the
common form of Bacterium:—“This infusorial animal
is so small that one cannot distinguish its germ, and
still less fix upon the presence of this germ, if it were
known, amongst the organized corpuscles of the dust
which is suspended in the air.”
Here, then, we have a confession from M. Pasteur
himself, that all evidence fails, where it is most wanted,
in support of his hypothesis.
If a large number of fermentations begin with the
presence of Bacteria as the only living things, and if
in a number of cases no other organisms ever occur, it
is useless to adduce as evidence, in proof of the view
that fermentations are always initiated by air-derived
organisms, the fact that certain corpuscles (supposed
to be spores of fungi) are recognizable in the atmosphere—capped
by the distinct statement19 that
Bacteria or their germs are not recognizable. If Bacteria
are not recognizable in the atmosphere, what
scientific evidence is there that the fermentations in
which these alone occur are initiated by Bacteria
derived from the atmosphere, or from certain imaginary
Bacteria germs,20 which we are supposed to be
unable to distinguish? M. Pasteur may, moreover,
be reminded that when he resorts to the supposition
of Bacteria possessing “germs” which are indistinguishable,
he is again resorting to hypothesis rather
than to fact, in order to prove the truth of the
particular doctrine of fermentation which he advocates.
Bacteria are known to reproduce and multiply
only by a process of fission; each of the parts into
which they divide being nothing more than a part of
the original Bacterium, and therefore endowed with
similar properties of resisting heat, desiccation, and
other agencies. Any resort to invisible germs to
account for the multiplication of Bacteria, which are
known to reproduce freely in other ways, is obviously
not permissible, unless such postulation be more or
less necessitated by the occurrence of facts otherwise
inexplicable.
Although, therefore, no direct evidence has been
adduced tending to show that Bacteria are present
in the atmosphere, even if this evidence had been
forthcoming, it would have been necessary, in reference
to M. Pasteur’s hypothesis, for it to be supplemented
by further evidence to the effect that Bacteria were
well capable of resisting such an amount of desiccation
as must have been involved by their presence for an
indefinite time in the atmosphere even of the hottest
and driest regions of the earth. For, organic substances
in solution do not only putrefy in moist
weather or moist climates; they putrefy most rapidly
and surely when the temperature is high, and quite
irrespectively of the amount of moisture contained
in the atmosphere. A property of resisting the
effects of desiccation—the possession of which, by
Bacteria, is so necessary for the truth of M. Pasteur’s
argument—ought to have been shown by scientific
evidence to be a real attribute of such organisms;
though it seems, on the contrary, to have been
assumed to exist, with almost equal readiness by both
parties, in the controversies concerning the possibility
of “spontaneous generation.” This error may be
ascribed to the misguiding influence of a treacherous
analogy. Whilst it may be true that certain seeds
and spores, and also that Rotifers, “Sloths,” and some
Nematoids are capable of resisting the influence of a
prolonged exposure to desiccating influences, it may
well be asked, whether the same fact necessarily holds
good for organisms such as Bacteria, which have no
chitinous or other envelopes to protect them, and
which are merely minute fragments of naked protoplasm.
Having elsewhere21 shown how far presumptions
had stolen a march upon established facts, in
reference to the supposed possession of a similar property
by the Free Nematoids, my eyes were opened
to the reality of this uncertainty with regard to Bacteria.
It is, however, no easy matter definitely to
prove or to disprove the possession of this property
by organisms so minute as Bacteria, and therefore so
difficult to identify. If dried Bacteria are added to a
drop of a suitable solution—similar to that in which
they had been bred—it soon becomes quite impossible
to distinguish those which have been added
from those which arise in the fluid. Taking into consideration
the fate of other simple organisms, however,
it is by no means improbable that they should be
killed even by a short desiccation. I have found, for
instance, that desiccation for half-an-hour in a room
at a temperature of 65° F. suffices to kill all the larger,
naked, lower organisms with which I have experimented—including
long Vibrios, Amœbæ, Monads,
Chlamydomonads, Euglenæ, Desmids, Vorticellæ and
all other Ciliated Infusoria.
But, certain indirect evidence seems to speak
most authoritatively against the supposition that the
air contains any notable quantity of living Bacteria,
or Bacteria germs, whether visible or invisible. I
have always found that a simple solution of ammonic
tartrate, which has been placed—without previous
boiling—in a corked bottle of greater capacity, will
become turbid in two or three days, owing to the
presence of myriads of Bacteria; whilst a similar
solution, previously boiled, may remain for ten days,
three weeks, or more, without showing the least trace
of turbidity, although the open neck of the bottle or
flask in which it is contained, may be covered only by
a loose cap of paper. And yet, at any time, in order to
make this fluid become turbid in from 24 to 48 hours,
all that one has to do is to bring it into contact with
a small glass rod which has just been dipped into a
solution containing living Bacteria.22
If we find that an eminently inoculable fluid will
remain for two or three weeks, or perhaps more,
in contact with the air without becoming turbid,
though it will always become turbid in two or three
days if brought into contact with living Bacteria, what
can we conclude, but that living Bacteria are not very
common in the atmosphere? These most striking
facts can be easily verified by other observers.
Thus we find ourselves, at present, in this position.
After all that has been said and done to prove the
wonderful prevalence of “germs” in the atmosphere,
we are really still in the region of hypothesis—no
further advanced than we were in the time of Bonnet
and of Spallanzani, so far as it concerns the organisms
which are all important—Bacteria. Neither these
nor their germs have been shown to exist in any
recognizable abundance in the atmosphere, and yet
in most fermentations they are the first organisms
which display themselves; whilst in many such
fermentations Bacteria alone occur. Nay more, even
were they present in any great abundance, there is
some reason to believe that the majority of them
would exist as mere dead, organic particles—because
Bacteria are more than likely to be unable to resist
anything like an extreme or prolonged exposure to
desiccating influences.
The first and essential data in support of M. Pasteur’s
hypothesis must, therefore, be regarded as
entirely unproved in respect to Bacteria—which are
the most important of all organisms, in relation to
the cause of fermentation and putrefaction.
Without the aid of elaborate experiments, however,
the evidence which the microscope can supply is
capable of leading us to the conclusion that such
search for atmospheric Bacteria germs, was comparatively
useless. If it can be shown that Bacteria
can arise in a fluid independently of visible germs,
then, obviously, any inquiries as to the nature of the
visible contents of the atmosphere, can have only a
very indirect bearing upon the question as to the
mode of origin of these organisms. And yet by the
aid of the microscope, as I have elsewhere stated,
one can watch the appearance of almost motionless
specks, more or less uniformly diffused through a
motionless film of fluid, and can see them gradually
develop into moving Bacteria or into Torulæ. So that,
where no visible germs previously existed, visible particles
of living matter develop, and more or less rapidly
grow into distinct Bacteria. This may be best seen in
a drop of a fresh and very strong turnip infusion, which
has been filtered several times through the finest paper.
The drop, placed in a live-box, should be flattened
into a thin film by the application of the cover.
Thus protected, evaporation takes place very
slowly, and with the live-box resting on one of
Stricker’s hot-water plates, at a temperature of 85° to
90° F., and the latter upon the stage of the microscope,
one can easily select a portion of the field in
which either no particles or only a countable number
exist. If, therefore, around and between any mere
granules which may pre-exist, or in a clear space, one
gradually sees in the course of two or perhaps three
hours, a multitude of almost motionless specks (at first
about 1/100000″ in diameter) in positions where no such
specks previously existed; and if these specks may
be seen gradually to increase in size and develop
into Bacteria and Torulæ, then, at all events, we are
able to say that these organisms can be developed
without pre-existing visible germs, and we have
just the same amount of actual evidence for believing
that they have been formed de novo, as we should
have for believing that crystals had been formed de
novo, if we had seen them appearing under our eyes in
the same manner. Whether they really arise after the
fashion of crystals, without the aid of pre-existing
though invisible germs, is a matter which can only be
settled inferentially, by a subsequent resort to strict
methods of experimentation.
Seeing however, that we are able, with the aid of
the microscope alone, to demonstrate that Bacteria
and Torulæ can develop in situations where no visible
germs had previously existed, it is useless, as I have
said before—so far as the question of their mode of
origin is concerned—to search the atmosphere to ascertain
what visible germs it may contain. If some Bacteria
and Torulæ arise from germs at all, it must be
from germs which are invisible to us. The finding of
visible germs in the atmosphere can, therefore, only
have an indirect bearing upon the solution of the problem.
Since it can be shown that some visible spores
and ova exist in the atmosphere, this affords a certain
amount of warrant for the supposition that invisible,
living, reproductive particles may also exist—more
especially if the existence of an amount of organic
matter, which is ordinarily invisible, can be revealed
in the air, by the agency of the electric beam, or by
any other means.
Nothing can be more illegitimate, however, in the
way of inference, than the assumption at once indulged
in by Prof. Tyndall and others (who might have been
expected, by their previous scientific work, to have
learned more caution) that this impalpable organic dust
was largely composed of impalpable germs. Yet, without
a shadow of proof, without even an attempt to
prove it, the air was for a time represented to be a
mere stirabout, thick with invisible germs. The
briefest reflection, however, upon the probabilities of
the case, should have sufficed to suggest a totally different
interpretation. The surface of the earth is
clothed with living things of all kinds, animal and
vegetal, which are not only continually throwing off
organic particles and fragments during their life, but
are constantly undergoing processes of decay and molecular
disintegration after their death. The actual reproductive
elements of these living things are extremely
small in bulk, when compared with the other
parts which are not reproductive, and although Bacteria
and Torulæ do exist abundantly, and do materially help
to bring about some of the decay in question, yet their
bulk, also, is extremely small in comparison with the
amount of organic matter itself that is continually
undergoing disintegration of a dry kind, in which
Bacteria and Torulæ take no part. When, moreover,
it is considered that in the neighbourhood of populous
cities (the air of which alone exhibits this very large
quantity of impalpable, mixed with palpable, organic
dust), there is constantly going on a wear and tear of
the textile fabrics and of the organic products of
various kinds which are daily subservient to the wants
of man; and that the chimneys of manufactories and
dwelling-houses are also continually emitting clouds
of smoke thick with imperfectly consumed organic
particles, some idea may be gained of the manifold
sources whence the organic particles and fragments
found in the atmosphere may emanate, and also as to
what proportion of them is likely to be composed of
living or dead reproductive elements, or “germs.”
Thus, then, so far as the two rival doctrines of fermentation
are concerned, the investigation of the
nature of the solid particles contained in the atmosphere
has revealed facts which are thoroughly in
harmony with all the requirements of Liebig’s physical
theory, though it has almost utterly failed to give
anything like a scientific basis to the vital theory of
Pasteur. So far from being able to show that living
Bacteria (which are the first and oftentimes the only
organisms concerned in many processes of fermentation
and putrefaction) are universally diffused through
the air, Pasteur admits that these cannot be detected,
and that their “germs” are not recognizable.
If, therefore, M. Pasteur still maintains the truth of
his theory, it should be distinctly understood that it
rests originally, not upon established facts, but upon
a mere hypothesis—the hypothesis that the air teems
with multitudes of invisible Bacteria germs. He is
driven to such a doctrine, not only by his own confessions
concerning Bacteria, but also by the microscopical
evidence to which I have referred.
So that in explaining the results of any experiments
made with the view of throwing light upon the
cause of fermentation or putrefaction, it is especially
necessary to bear in mind two considerations:—
I. That dust filtered from the atmosphere cannot
be proved to include living Bacteria; though it is
known to contain a multitude of organic particles
which may be capable in the presence of water, in accordance
with Liebig’s hypothesis, of acting as ferments.
II. It must also be recollected that, in the opinion
of many, Life represents a higher function which is
displayed by certain kinds of organic matter; and that
this higher function may be deteriorated or rendered
non-existent by an amount of heat which might not
be adequate to decompose the organic matter itself.
It is all the more necessary to call attention to
these two considerations, because M. Pasteur invariably
speaks as though it had been established that
the air contains multitudes of living Bacteria, when,
really, he had only proved that the air contains a
number of corpuscles resembling spores of fungi, &c.
And, as I have already intimated, the existence of
spores of fungi in the atmosphere, however well
established, is of little or no importance as an explanation
of the cause of a very large number of
fermentations. Their presence is even of still less importance,
owing to the fact of the co-existence with
these fungus-spores, of multitudes of organic fragments,
which—in accordance with the views of Liebig,
Gerhardt, and other chemists—are capable of acting
as ferments. To this latter consideration M. Pasteur
never even alludes when he speaks (loc. cit. p. 40) of his
“ensemencements,” and of other experiments which
are equally, or even more, capable of being interpreted
in accordance with Liebig’s views than with his own.
Bearing these considerations in mind, we shall be in
a better position to enquire into the real interpretation
that may be given to many of M. Pasteur’s results,
and into the question as to how far the facts which he
records are favourable to his own, or to the adverse
doctrine concerning the causes of fermentation.
In the memoir so often alluded to on “The Organized
Corpuscles which exist in the Atmosphere,” M. Pasteur
adduced various kinds of evidence, tending,
as he thought, to show that the first Bacteria which
make their appearance in putrefying or fermenting solutions,
have been derived from living Bacteria or their
“germs,” which pre-existed in the atmosphere.
Some of the experiments by which he endeavoured
to substantiate this position were of a very
simple nature. Their narration attracted much attention
at the time, as it was supposed that by their
means M. Pasteur had—as he professed—conclusively
shown the erroneousness of the views of those
who believed in what was called “spontaneous generation.”
These experiments were soon repeated by
other observers, who, using different fluids, obtained
quite opposite results. Thus it became obvious to
impartial critics, that whilst the means adopted by
M. Pasteur might be adequate to check the processes
of fermentation or putrefaction in certain fluids, they
were quite powerless to effect this when many other
fluids were employed.
These particular experiments, however, still seem
to exercise a very great influence on the minds of many
in this country, who are either unaware of, or disbelieve
in, the possibility of obtaining opposite results.
The chapter in which M. Pasteur detailed these
experiments is thus entitled:—“Another very simple
method of demonstrating that all the organized products
of Infusions (previously heated) owe their origin to the
corpuscles which exist suspended in the Atmosphere.”
Whilst claiming to have already rigorously established
the validity of this conclusion by the experiments
described in previous chapters, M. Pasteur adds:—“If
there remained the least doubt on this subject, in the
mind of the reader, it would be dissipated by the experiments
of which I am now about to speak.” (p. 66.)
Sweetened yeast-water, urine, infusions of pear and
of beetroot, were placed in flasks with long necks,
variously drawn out and bent. The flasks were subsequently
treated as follows. M. Pasteur says:—“I
then raise the liquid to the boiling-point for several
minutes until steam issues abundantly from the extremity
of the drawn-out neck of the flask, which is
permitted to remain open. I then allow the flask to
cool. But, singular fact—and one well calculated to
astonish every one acquainted with the delicacy of the
experiments relating to what is called ‘spontaneous
generation’—the liquid of this flask will remain indefinitely
without alteration. The flask may be handled
without any fear, it may be transported from place to
place, allowed to experience all the seasonal variations
of temperature, and its liquid does not undergo the
slightest alteration, whilst it preserves its odour and its
taste.” If, however, the neck of one of these flasks be
broken off close to the flask itself, then, according to
M. Pasteur, the previously unaltered fluid will, in a
day or two, undergo the ordinary changes, and swarm
with Bacteria and Mucedineæ.
“The great interest of this method is,” M. Pasteur
adds, “that it completes, unanswerably, the proof that
the origin of life in infusions which have been raised
to the boiling point, is solely due to the solid particles23
which are suspended in the air.” He believes that any
living things pre-existing in the fluid itself would be
destroyed by the high temperature to which it had been
raised; and that those contained in the air of the flask
would also be destroyed, if not expelled, by the process
of ebullition. Believing that the air is the source of
germs from which Life is first developed in infusions,
he thinks that what rapidly enters at first, on the
cessation of ebullition, has its germs destroyed by
contact with the almost boiling liquid; whilst the air
which enters subsequently, and more slowly, is supposed
to deposit its germs in the various flexures of
the tubes, so that none are able to reach the fluid
itself. Infusions, thus protected, do not undergo putrefaction,
says M. Pasteur, because the access of pre-existing
living things is necessary for the initiation of
this change, and such access is prevented by the tortuous
and bent neck of the flask.
Others say that some fluids submitted to the conditions
mentioned, will undergo putrefactive changes,
and that, therefore, these experiments of M. Pasteur
are utterly incapable of settling the general question
as to the cause of fermentation and putrefaction, and
also that concerning the origin of Life. Although
acknowledging a certain difficulty in explaining the
results which are sometimes attained by this method,
some of us would rather confess this than confidently
offer explanations—as M. Pasteur did—which may in
a short time be stultified by the results of other experiments
with different fluids.
Having previously shown24 that living things could
appear and multiply in such a flask as M. Pasteur
describes—in any flask, in fact,—which had been hermetically
sealed during the ebullition of a suitable fluid
within; this was deemed to be a result so contradictory
to the explanations of M. Pasteur, that it appeared
needless to add my testimony, as I could have done,
to that of M. Victor Meunier and others, as to the
different results obtainable by operating, in M. Pasteur’s
fashion, with different fluids. It seemed to me
that if organisms were to be procured in flasks from
which air had been altogether expelled, it was useless
still to urge the preservative virtues of any process of
filtration of air—with the object of showing that living
things in infusions derived their origin from atmospheric
germs. Obviously, if there were no atmosphere,
there could be no atmospheric germs present; and if
living things were, nevertheless, developed under these
exclusive circumstances, how could M. Pasteur or his
disciples still expect to convince others that the first
living things in infusions always proceeded from pre-existing
atmospheric germs—even although it could
be shown, that in many cases, when these were filtered
off by flasks with narrow and tortuous necks, no
living things were developed in such fluids. Granting
to the full the truth of such facts, they could do
nothing to establish the doctrine of the origin of infusorial
life from pre-existing atmospheric germs, so long
as it could also be shown that living things might be
developed in boiled solutions to which air, instead of
being filtered, was never allowed to enter at all.
It is not, therefore, because I think that some of the
experiments which will subsequently be related afford
any stronger or more direct support to my own conclusions,
but because I think they may do this indirectly—by
shaking the faith of many in some of the
reasonings of M. Pasteur—that I am induced to give
an account of them.25
What has been hitherto said, also applies to the more
recent statements concerning the efficacy of cotton-wool
as an agent for filtering germs from the atmosphere.
Prof. Huxley says he has never seen putrefaction or
fermentation occur after certain organic fluids have
been boiled for ten or fifteen minutes, if a good plug
of cotton-wool has been inserted into the neck of the
flask in which they are contained whilst ebullition is
going on, and has, subsequently, been allowed to remain
in the same situation. Using other or perhaps stronger
fluids, however, I have found that such a method of
proceeding is by no means adequate to stop the growth
and development of organisms. And, also, even if it
had been always efficacious—the reason adduced
could not hold good, in the face of my other experiments,
which had shown that a development of life
might go on in cases where the air, which had been
similarly driven out, was subsequently, in place of
being filtered, prevented from gaining access to the
fluid.
If germs derived from the air are the sole causes of
putrefaction, then, surely, deprivation from air ought
to be just as efficacious as any process of filtration of
air—more especially when the filtration or the deprivation
have a common starting point. And the mode
of procedure, in both cases, is precisely the same up to
a certain point. A fluid is boiled for a short time
in order to kill the germs which may be within the
flask, and to expel its previously contained air. At
a certain stage of the ebullition, this may be arrested,
if we have to do with a bent-neck flask, or one
whose neck is plugged with cotton-wool, and no
change, it is said, will subsequently take place in the
contained fluid, because the air which enters is, by
either of these means, filtered from its germs. But
if, whilst ebullition continued, the neck of the flask
had been hermetically sealed—so as altogether to
prevent the re-ingress of air—and if the fluid, thus
contained in vacuo, would nevertheless undergo fermentation,
obviously the former explanation must be
altogether shelved.
In the face of M. Pasteur’s explanations, and those of
Professor Huxley, these frequent positive results with
fluids contained in vacuo are absolutely contradictory.
There may naturally arise, therefore, a very grave doubt
as to the validity of the explanation adduced by M. Pasteur,
and adopted by Professor Huxley and others.
All these experiments to which I have been alluding
are based upon the supposition (assented to by Pasteur
and Huxley) that Bacteria which pre-existed in
the solution would certainly be destroyed by its being
raised for a few minutes to a temperature of 212° F.
This conclusion is, I believe, perfectly correct,26 and in
support thereof I will adduce the following additional
information.
After stating elsewhere27, that Vibriones are partly
broken up or disintegrated by an exposure for a few
minutes to a temperature of 212° F. in an infusion
which is being boiled, and also that, in all probability,
the life of Bacteria would be destroyed by such a
treatment, I made the following remarks:—“With
reference to these organisms, however, one caution is
necessary to be borne in mind by the experimenter.
The movements of monads and Bacteria may be, and
frequently are, of two kinds. The one variety does
not differ in the least from the mere molecular or
Brownian movement, which may be witnessed in
similarly minute, not-living particles immersed in
fluids. Whilst the other seems to be purely vital—that
is, dependent upon their properties as living
things. These vital movements are altogether different
from the mere dancing oscillations which not-living
particles display, as may be seen when the
monad or Bacterium darts about over comparatively
large areas, so as frequently to disappear from the
field. After an infusion has been exposed for a second
or two to the boiling temperature, these vital movements
no longer occur, though almost all the monads
and Bacteria may be seen to display the Brownian
movement in a well-marked degree. They seem to
be reduced by the shortest exposure to a temperature
of 100° C. to the condition of mere not-living particles,
and then they become subjected to the unimpaired
influence of the physical conditions which
determine these movements.” I now have various
facts to add in confirmation of these conclusions, and
in extension of our knowledge concerning the vital
resistance to heat of Bacteria and Torulæ.
It would be a most important step if we could
ascertain some means by which these primary movements
of living Bacteria might be distinguished from
the secondary, or communicated, movements of not-living
particles. In many cases, organisms that are
truly living may only exhibit very languid movements,
which, as movements, are quite indistinguishable from
those that the same Bacteria may display when they
are really dead. Because the movements, therefore,
are of this doubtful character, persons are apt, unfairly,
to argue that the Bacteria which present them, are no
more living than are the minute particles of carbon
obtained from the flame of a lamp, which may exhibit
similar movements. This, however, is a point of view
which becomes obviously misleading if too much stress
is laid upon it; and it is more especially so in this
case, when those Bacteria which display the most
characteristic sign of vitality—viz., “spontaneous”
division or reproduction—do, at the time, almost
always exhibit only the same languid movements.
Mobility is, in fact, not an essential characteristic of
living Bacteria, whilst the occurrence of the act of reproduction
is the most indubitable sign of their life. It
should be remembered, therefore, that any Bacteria
which are almost motionless, or which exhibit mere
Brownian movements, may be living, whilst those
which spontaneously divide and reproduce, are certainly
alive—whatever may be the kind of movement
they present.
In any particular case, however, can we decide
whether Bacteria, that have been submitted to a given
temperature, and which exhibit movements resembling
those known as Brownian, are really dead or
living? If the movements are primary, or dependent
upon the inherent molecular activity of the organism
itself, they ought, it might be argued, to continue
when the molecules of the fluid are at rest; if, on the
other hand, they are mere secondary or communicated
movements, impressed upon the organisms as they
would be upon any other similarly minute particles,
by the molecular oscillations of the fluid in which they
are contained, then the movements ought to grow less,
and gradually cease, as the fluid approaches a state of
molecular rest—if this be attainable. Following out
this idea, some months ago, I first tested the correctness
of the assumption by experimenting with fluids
containing various kinds of not-living particles; such
as carbon-particles from the flame of a lamp, or freshly
precipitated baric sulphate. However perfect may
have been the Brownian movements when portions of
these fluids were first examined beneath a covering-glass,
they always gradually diminished, after the
specimen had been mounted by surrounding the
covering-glass with some cement or varnish. Thus
prepared, no evaporation could take place from the
thin film of fluid, and after one, three, four, or more
hours—the slide remaining undisturbed—most of
the particles had subsided, and were found to have
come to a state of rest. In order still further to test
these views, I took an infusion of turnip, containing
a multitude of Bacteria whose movements were
of the languid description, and divided it into two
portions. One of these portions was boiled for about
a minute, whilst the other was not interfered with.
Then, after the boiled solution had been cooled, a
drop was taken from each and placed at some little
distance from one another on the same glass slip;
covering-glasses half an inch in diameter were laid
on, and the superfluous fluid beneath each was removed
by a piece of blotting-paper. When only
the thinnest film of fluid was left, the covering-glasses
were surrounded by a thick, quickly-drying
cement.28 Examined with the microscope immediately
afterwards, it was generally found that the Bacteria
which had been boiled presented a shrunken and
shrivelled aspect—whilst some of them were more
or less disintegrated—though, as far as movement
was concerned, there was little to distinguish that
which they manifested, from that of their plumper-looking
relatives which had not been boiled.
If the specimens were examined again after twenty-four
or more hours, there was still very little difference
perceptible between them, as regards their movements.
And the same was the case when the specimens
were examined after a lapse of some days or
weeks. One important difference does, however, soon
become obvious. The Bacteria which have not been
boiled, undergo a most unmistakeable increase within
their imprisoned habitat; whilst those which have been
boiled, do not increase. The two films may be almost
colourless at first (if the Bacteria are not very abundant),
but after a few days, that composed of unboiled fluid
begins to show an obvious and increasing cloudiness,
which is never manifested by the other. Microscopical
examination shows that this cloudiness is due to
a proportionate increase in the number of Bacteria.
Is the continuance of the movements of the organisms
which had been boiled attributable to their
extreme lightness, and to the slight difference between
their specific gravity and that of the fluid in which
they are immersed? I soon became convinced that
this was one, if not the chief reason, when I found
that Bacteria which had been submitted to very much
higher temperatures, behaved in precisely the same
manner as those which had been merely boiled, and
also that other particles which—though obviously
dead—had a similar specific lightness, also continued
to exhibit their Brownian movements for days and
weeks. This was the case more especially with the
minute fat particles in a mounted specimen of boiled
milk,29 and also with very minute particles which were
gradually precipitated30 from a hay infusion that had
been heated to 302° F. for four hours. Trials with many
different substances, indeed, after a time convinced me
that the most rapid cessation of Brownian movements
in stationary films,31 occurred where the particles were
heavy or large; and that the duration of the movement
was more and more prolonged, as the particles
experimented with, were lighter or more minute.
So that, when we have to do with Bacteria, the minute
oil globules of milk, or with other similarly light particles,
the movements continue for an indefinite time,
and are, in part, mere exponents of the molecular
unrest of the fluid. They are always capable of being
increased or renewed by the incidence of heat or other
disturbing agencies.
In respect of the movements which they may exhibit,
therefore, really living, though languid, Bacteria,
cannot always be discriminated from dead Bacteria.
Both may only display mere Brownian movements.
It becomes obvious, then, that in doubtful cases we
ought not to rely very strongly upon the character of
their movements, as evidence of the death of Bacteria—although
these may frequently be of so extensive
a nature as to render it not at all doubtful whether
the Bacteria which display them are living. In the
experiments which I am about to relate, we shall be
able to pronounce that the Bacteria are living or dead,
by reference to the continuance or cessation of their
most essentially vital characteristic. If Bacteria fail
to multiply in a suitable fluid, and under suitable conditions,
we have the best proof that can be obtained
of their death.
Having made many experiments with solutions of
ammonic tartrate and sodic phosphate, I have almost
invariably observed that such solutions—when exposed
to the air without having been boiled—become turbid
in the course of a few days owing to the presence of
myriads of Bacteria and Vibriones, with some Torulæ.
These organisms seem to appear and multiply in such
a solution almost as readily as they do in an organic
infusion. On the other hand, having frequently boiled
such solutions, and closed the flasks during ebullition,
I have invariably found, on subsequent examination
of these fluids, that whatever else may have been met
with, Bacteria and Vibriones were always absent. The
difference was most notable, and it seemed only intelligible
on the supposition that any living Bacteria or
dead ferments which may have pre-existed in the
solution, were deprived of their virtues by the preliminary
boiling. These experiments also seemed to
show that such solutions, after having been boiled, and
shut up in hermetically-sealed flasks, from which all
air had been expelled, were quite incapable of giving
birth to Bacteria. The unboiled fluid, exposed to the
air, might have become turbid, because it was able to
nourish any living Bacteria which it may have contained,
or because it was capable of evolving these de
novo, under the influence of dead ferments whose activity
had not been destroyed by heat. Hence we have
a fluid which is eminently suitable for testing the vital
resistance of Bacteria,—one which, although quite
capable of nourishing and favouring their reproduction,
does not appear capable of evolving them, when,
after previous ebullition, it is enclosed in a hermetically
sealed flask from which all air has been
expelled. Three flasks were half-filled with this solution.32
The neck of the first (a) was allowed to remain
open, and no addition was made to the fluid. To the
second (b), after it had been boiled and had become
cool, was added half a minim of a similar saline solution,
which had been previously exposed to the air,
and which was quite turbid with Bacteria, Vibriones
and Torulæ. From this flask—after its inoculation
with the living organisms—the air was exhausted
by means of an air-pump, and its neck was hermetically
sealed during the ebullition of the fluid, without
the flask and its contents having been exposed to a
heat of more than 90° F. The third flask (c) was
similarly inoculated with living Bacteria, although its
contents were boiled for ten minutes (at 212° F.), and
its neck was hermetically sealed during ebullition. The
results were as follows:—the solution in the first flask
(a), became turbid in four or five days; the solution
in the second (b), became turbid after thirty-six hours;
whilst that in the third flask (c), remained perfectly
clear. This latter flask was opened on the twelfth
day, whilst its contents were still clear, and on microscopical
examination of the fluid no living Bacteria
were to be found. This particular experiment was
repeated three times with similarly negative results,
although on two occasions the fluid was only boiled
for one minute instead of ten.
It seemed, moreover, that by having recourse to experiments
of the same kind, the exact degree of heat,
which is fatal to Bacteria and Torulæ might be ascertained.
I accordingly endeavoured to determine
this point. Portions of the same saline solution,
after having been boiled33 and allowed to cool,
were similarly inoculated with a drop34 of very
turbid fluid, containing hundreds of living Bacteria,
Vibriones, and Torulæ. A drying apparatus was fixed
to an air-pump, and the flask containing the inoculated
fluid was securely connected with the former by
means of a piece of tight india-rubber tubing,35 after
its neck had been drawn out and narrowed, at about
two inches from the extremity. The flask containing
the inoculated fluid was then allowed to dip into a
beaker holding water at 122° F., in which a thermometer
was immersed. The temperature of the fluid was maintained
at this point for fifteen minutes,36 by means of a
spirit lamp beneath the beaker. The air was then
exhausted from the flask by means of the pump, till
the fluid began to boil; ebullition was allowed to continue
for a minute or two, so as to expel as much air
as possible from the flask, and then, during its continuance,
the narrowed neck of the flask was hermetically
sealed by means of a spirit-lamp flame and a blowpipe.
Other flasks were similarly prepared, except
that they were exposed to successively higher degrees
of heat—the fluid being boiled off, in different cases,
at temperatures of 131°, 140°, 149°, 158°, and 167° F.
All the flasks being similarly inoculated with living
Bacteria, Vibriones, and Torulæ, and similarly sealed
during ebullition, they differed from one another only
in respect to the degree of heat to which they had
been submitted. Their bulbs were subsequently placed
in a water bath, which during both day and night was
maintained at a temperature of from 85° to 95° F.
The results have been as follows:—The flasks whose
contents had been heated to 122° and 131° F. respectively,
began to exhibit a bluish tinge in the
contained fluid after the first or second day; and
after two or three more days, the fluid in each became
quite turbid and opaque, owing to the presence and
multiplication of myriads of Bacteria, Vibriones and
Torulæ; the fluids in the flasks, however, which had
been exposed to the higher temperature of 140°, 149°,
158°, and 167° F., showed not the slightest trace of
turbidity, and no diminution in the clearness of the
fluid while they were kept under observation—that
is, for a period of twelve or fourteen days. One kind
of conclusion only is to be drawn from these experiments,
the conditions of which were in every way
similar, except as regards the degree of heat to which
the inoculated fluids were subjected—seeing that the
organisms were contained in a fluid, which had been
proved to be eminently suitable for their growth and
multiplication.37 If inoculated fluids which have been
raised to 122° and 131° F. for ten minutes, are found
in the course of a few days to become turbid, then,
obviously, the organisms cannot have been killed
by such exposure; whilst, if similar fluids, similarly
inoculated, which have been raised to temperatures
of 140°, 149°, 158°, and 167° F. remain sterile, such
sterility can only be explained by the supposition
that the organisms have been killed by exposure to
these temperatures.
Some of these experiments have been repeated
several times with the same results. On three occasions,
I have found the fluid speedily become turbid,
which had only been exposed to 131° F. for ten
minutes, whilst on three other occasions I have found
the inoculated fluid remain clear, after it had been
exposed to a heat of 140° F. for ten minutes.38
In experimenting upon rather higher organisms,
with which there is little difficulty in ascertaining, by
microscopical examination, whether they are living or
dead, I have found that an exposure even to the lower
temperature of 131° F. for five minutes, always suffices
to destroy all signs of life in Vibrios, Amœbæ, Monads,
Chlamydomonads, Euglenæ, Desmids, Vorticellæ,
and all other Ciliated Infusoria which were observed,
as well as in free Nematoids, Rotifers, and
other organisms contained in the fluids which had
been heated.
These results are quite in harmony with the
observations and experiments of M. Pouchet and
of Professor Wyman, as to the capability of resisting
heat displayed by Vibriones and all kinds of ciliated
infusoria. According to the former,39 the majority
of ciliated infusoria are killed at, or even below, the
temperature of 122° F., whilst large Vibriones are all
killed at a temperature of 131° F.40 According to the
observations of Professor Wyman, the motions of all
ciliated infusoria are stopped at less than 130° F.,
whilst Vibriones, taken from the most various sources,
also seemed to be killed at temperatures between
130°–136.4° F. Similarly, we find Baron Liebig quite
recently making the following remarks concerning
a species of Torula:—“A temperature of 60° C.
[140° F.] kills the yeast cells; after exposure to this
temperature in water, they no longer undergo fermentation,
and do not cause fermentation in a sugar
solution. . . . In like manner, active fermentation in
a saccharine liquid is stopped when the liquid is
heated to 60° C., and it does not recommence again
on cooling the liquid.”
That the organisms in question—being minute naked
portions of living matter—should be killed by exposure
to the influence of a fluid at these temperatures will
perhaps not seem very improbable to those who have
attempted to keep their fingers for any length of time
in water heated to a similar extent. With watch in
hand I immersed my fingers in one of the experimental
beakers containing water at 131° F., and found that, in
spite of my desires, they were hastily withdrawn, after
an exposure of less than five-and-twenty seconds.
Wishing to ascertain what difference there would
be if the inoculated fluids were exposed for a very
long time, instead of for ten minutes only, to certain
temperatures, I prepared three flasks in the same
manner—each containing some of the previously
boiled solution, which, when cold, had been inoculated
with living Bacteria, Vibriones, and Torulæ. These
flasks and their contents were then submitted to the
influence of the following conditions:—One of them
was heated for a few minutes in a beaker containing
water at 113° F., and then by means of the air-pump
a partial vacuum was procured, till the fluid began to
boil. After the remainder of the air had been expelled
by the ebullition of the fluid, the neck of the flask was
hermetically sealed, and the flask itself was subsequently
immersed in the water of the beaker, which
was kept for four hours at a temperature between 113°
and 118 1/2° F.41 The two other flasks similarly prepared
were kept at a temperature of 118 1/2°–127 1/2° F. for
four hours. In two days, the fluid in the first flask
became slightly turbid, whilst in two days more the
turbidity was most marked. The fluid in the two
other flasks which had been exposed to the temperature
of 118 1/2°–127 1/2° F. for four hours, remained quite
clear and unaltered during the twelve days in which
they were kept in the warm bath under observation.
These experiments seem to show, therefore, that the
prolongation of the period of exposure to four hours,
suffices to lower the vital resistance to heat of Bacteria
and Torulæ by 14 1/2°–18° F.
Such experiments would seem to be most important
and crucial in their nature. They may be
considered to settle the question as to the vital
resistance of these particular Bacteria, whilst other
evidence points conclusively in the direction that
all Bacteria, whencesoever they have been derived,
possess essentially similar vital endowments42. Seeing
also that the solutions have been inoculated with a drop
of a fluid in which Bacteria, Vibriones, and Torulæ
are multiplying rapidly, we must suppose that they
are multiplying in their accustomed manner, as much
by the known method of fission, as by any unknown
and assumed method of reproduction. In such a
fluid, at all events, there would be all the kinds of
reproductive elements common to Bacteria, whether
visible or invisible, and these would have been alike
subjected to the influence of the same temperature.
These experiments seem to show, therefore, that even
if Bacteria do multiply by means of invisible gemmules
as well as by the known process of fission, such
invisible particles possess no higher power of resisting
the destructive influence of heat than the parent
Bacteria themselves possess. This result is, moreover,
as I venture to think, in accordance with what
might have been anticipated à priori. Bacteria seem
to be composed of homogeneous living matter, and
any gemmule, however minute, could only be a
portion of such living matter, endowed with similar
properties.
Having thus satisfied ourselves as to the truth of
the conclusion that Bacteria are killed when the fluid
containing them is boiled (at 212° F.), we are in a position
to proceed with the inquiry as to the evidence
which exists in respect to the statements made by
M. Pasteur, Professor Huxley, and others, that fermentable
fluids which have been boiled, will not undergo
fermentation, either in vessels whose necks have been
many times bent, or in those into whose necks a
plug of cotton-wool has been inserted during the
ebullition of their contained fluid. Organisms are
not found in such cases, they say, because the
“germs” from which the low organisms of infusions
are usually produced, are arrested either in the
flexures of the tube or in the cotton-wool. As I have
before stated, however, it is obvious that if this
explanation be the correct one, the preservation
should be equally well marked in all cases—quite
irrespectively of the amount of albumenoid or other
nitrogenous material which may be contained in the
fluid. Any exceptions to the rule should at once
suggest doubts as to the validity of the explanation.
It was shown43 in 1865 by M. Victor Meunier that
some fluids were preserved after having been boiled in
a vessel of this kind, whilst others, submitted to the
same treatment, speedily became turbid from the presence
of Bacteria and other organisms.44 By these
experiments he ascertained that strong infusions did
frequently change, whilst weak ones might be preserved;
and that even a strong infusion might be
prevented from undergoing change if the period of
ebullition were sufficiently prolonged.
The fluids most frequently employed by M. Pasteur
were yeast-water, the same sweetened by sugar, urine,
infusion of beetroot, and infusion of pear.
Taking urine as a fair example of such a fluid, I
have found that the statements of M. Pasteur and of
Professor Lister are perfectly correct. This fluid may
generally remain for an indefinite period in such vessels45
without becoming turbid, or undergoing any
apparent change. The same is generally found to
be the case with an infusion of turnip, and occasionally
an infusion of hay may be similarly prevented
from undergoing fermentation. On the other hand, if
the turnip-solution be neutralized by the addition of
a little ammonic carbonate, or liquor potassæ; or,
better still, if even half a grain of new cheese be added
to the infusion before it is boiled, then I have found
that the fluid speedily becomes turbid, owing to the
appearance of multitudes of Bacteria. In an infusion
to which a fragment of cheese had been added, I have
seen a pellicle form in three days, which, on microscopical
examination, proved to be composed of an
aggregation of Bacteria, Vibriones, and Leptothrix filaments.
A mixture of albuminous urine and turnip-infusion
has also rapidly become turbid in a vessel of
this kind owing to the appearance of multitudes of
Bacteria, and so has a mixture containing one-third
of healthy urine with two-thirds of infusion of turnip.
Other infusions have been boiled for ten minutes in a
vessel with a horizontal neck two feet long, into which,
during ebullition, a good plug of cotton-wool had been
carefully pushed down for a depth of twelve or fourteen
inches, and cautiously increased in quantity during
the continuance of the ebullition; whilst immediately
after the withdrawal of the heat, the plug was pressed
closer, and all the outer unoccupied portion of the
tube was rapidly filled up in the same manner.
Preserved in such a vessel, a specimen of urine
remained unchanged; a hay-infusion also underwent
no apparent alteration; whilst a very strong infusion
of turnip became turbid in five days, and ultimately
showed a large quantity of deposit.46
Thus the rules laid down by Pasteur and others
are not universal, and therefore, as I have previously
pointed out, the explanation which he adduced of the
preservation of those particular fluids which remained
unchanged is at once rendered doubtful. More especially
is there room for doubt on this subject when, as
I have found, the result of the experiment can be,
within certain limits, predicated beforehand, according
to the nature of the fluid employed. If all organisms
proceed from pre-existing germs, and these can be
filtered from the air by a certain mechanical contrivance,
then, if it be alleged that it is on account of
such filtration that certain boiled fluids do not change,
all fluids placed under these conditions ought, on this
theory, to be similarly preserved. Exceptional cases
cannot be accounted for on this hypothesis. To
others, however, who say that organisms are capable
of arising de novo, and that fermentation can be
initiated without the agency of living things, the
above facts appear quite natural. The more complex
the nitrogenous or protein materials contained in a
solution, the more is it fitted to undergo fermentative
changes, which may be accompanied by the de
novo origination of living things. Therefore the above
results are just as compatible with the notions of
M. Liebig and his school, as they are antagonistic
to those of M. Pasteur. Certain fluids, it is found, do
not undergo change; whilst other fluids, of a more
complex description, will ferment under the influence
of similar conditions. Prolonged ebullition also, by
breaking up some of the more unstable compounds
of a solution (those which most easily initiate these
changes) will retard or prevent its fermentation.
The complete untenability of M. Pasteur’s explanations
are, however, best revealed by having recourse to
a series of comparative experiments, in which portions
of the same fluid are boiled for an equal length of time
in vessels of different kinds, and are then subsequently
submitted, in a water-bath, to the influence of the
same temperature.
I have made many experiments of this kind with
different solutions, some of which I will now record.
Owing to the different behaviour of the same fluids
under different conditions, we are enabled to draw
some most important conclusions; and owing to the
different behaviour of different fluids under these
respective conditions, our attention is strongly drawn
to other facts which ought considerably to influence
our judgment as to the relative merits of the two
doctrines concerning the cause of fermentation and
putrefaction.