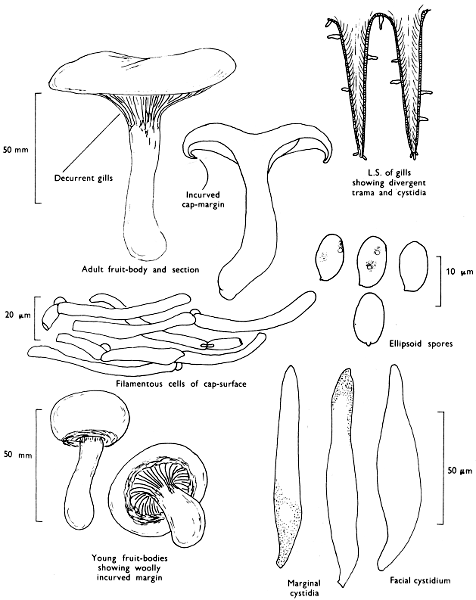
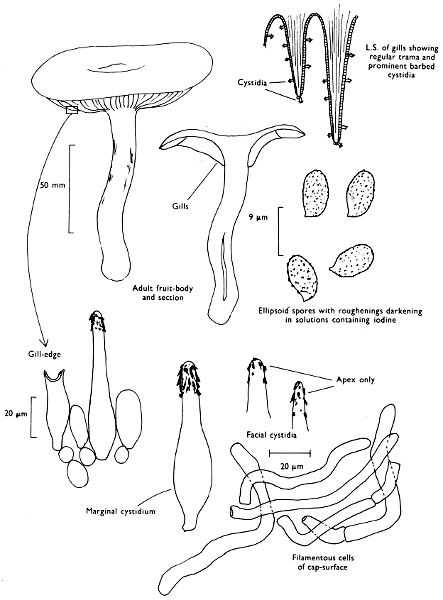
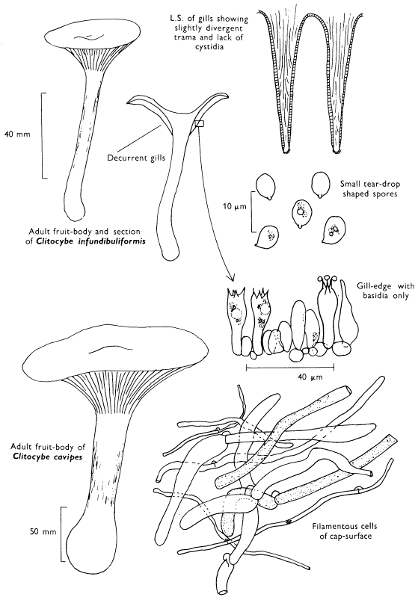
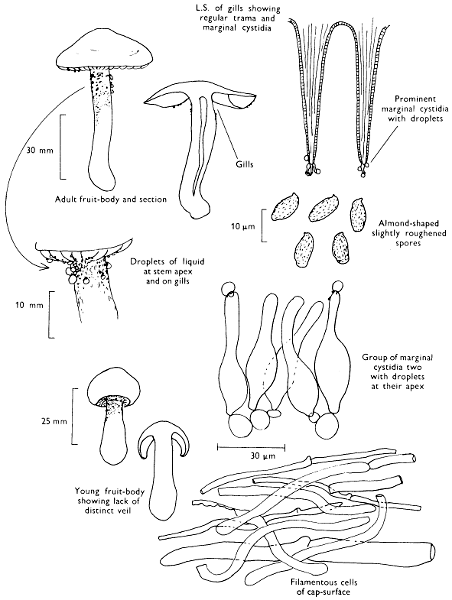
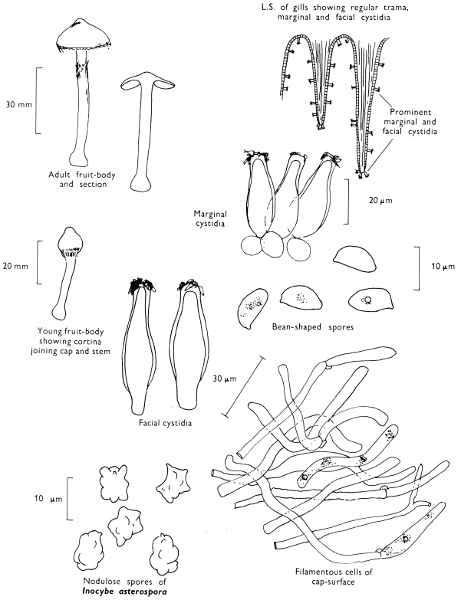
- 1. Spores distinctly coloured in mass and coloured individually under the microscope
2
- Spores not, or faintly, coloured in mass and hyaline under the microscope
25
- 2. Spores blackish or some shade of brown
8
- Spores pinkish
3
- 3. Stem laterally attached to the cap or absent
Claudopus (and some species of Clitopilus)
- Stem centrally attached to the cap
4
- 4. Stem with a cup-like structure enveloping the base
Volvariella
- Stem lacking any special structure at its base
5
- 5. Gills not attached to the stem (free), or with part attached to and descending down the stem (decurrent)
6
- Gills attached to the stem but not descending down the stem
7
- 6. Gills remote to free from the stem
Pluteus
- Gills distinctly attached and descending down the stem
Clitopilus (see also Eccilia p. 102)
- 7. Gills broadly attached to the stem (adnate)
Entoloma
- Gills narrowly attached to the stem (adnexed)
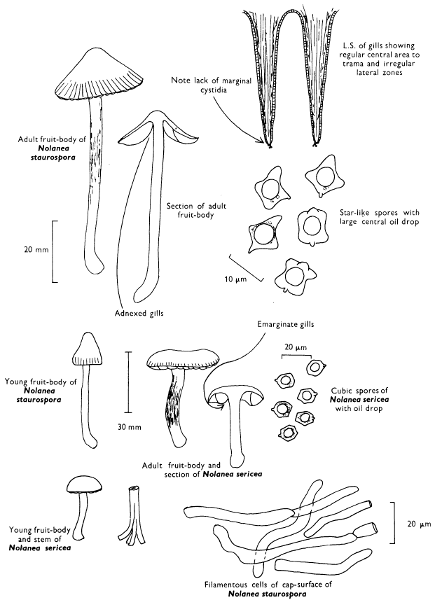
Leptonia & Nolanea
- 8. Stem laterally attached to the cap
Crepidotus
- Stem centrally attached to the cap
9
- 9. Spore-print some shade of brown
10
- Spore-print blackish to purplish black
18
- 10. Spore-print bright rust-brown
11
- Spore-print dull clay-brown or ochraceous
16
- 11. Stem with the veil girdling the stem (ring), or cobweb-like (cortina)
12
- Stem without the veil girdling the stem or when present then easily lost
13
- 12. Stem with distinct ring or ring-zone
Pholiota & related genera
- Stem with cobweb-like veil or faint filamentous ring-zone
Cortinarius & Gymnopilus
- 13. Gills attached to the stem but not descending down the stem (adnexed to adnate)
14
- Gills free of the stem, or distinctly attached to and running down the stem (decurrent),
and then often joined together at the apex of the stem or at their base
15
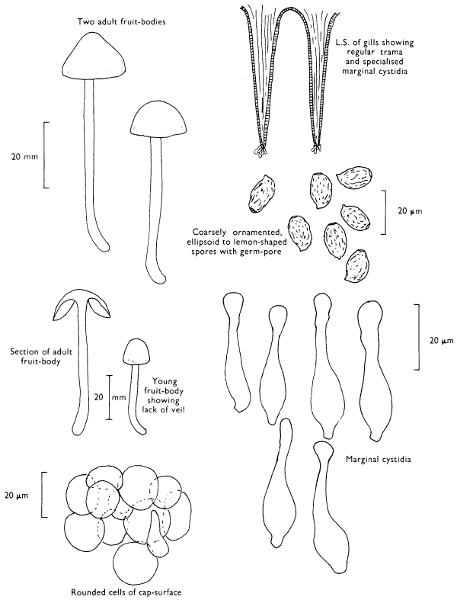
- 14. Cap-surface composed of rounded cells
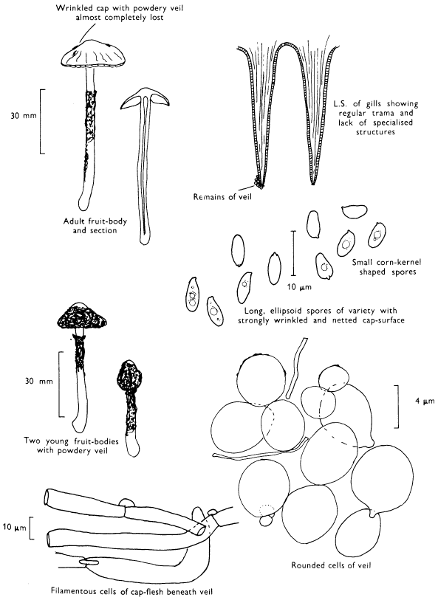
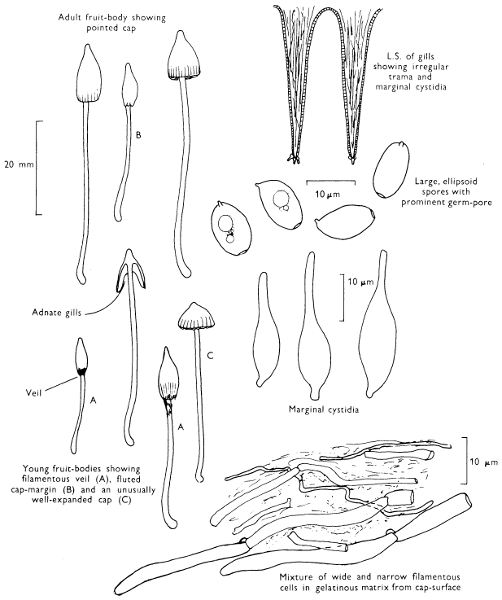
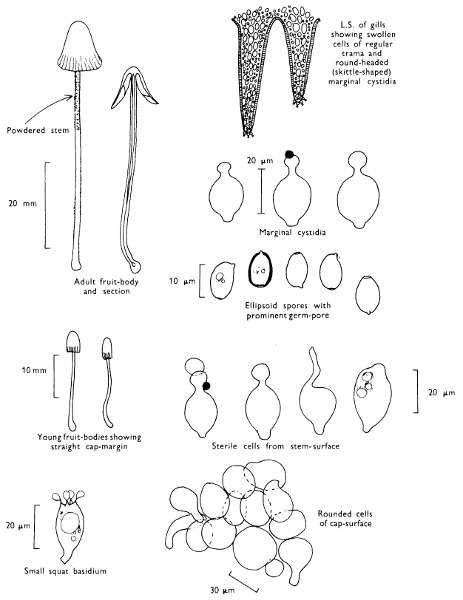
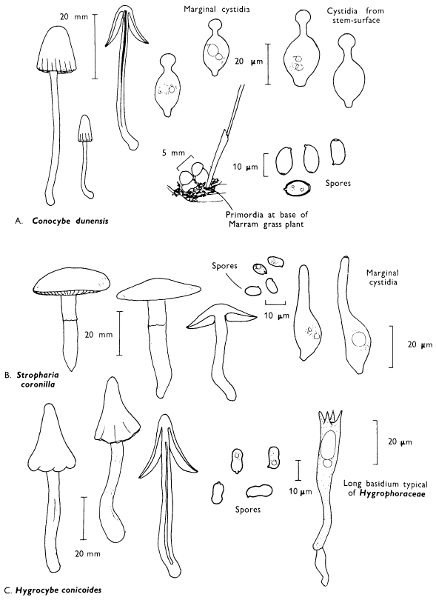
Conocybe
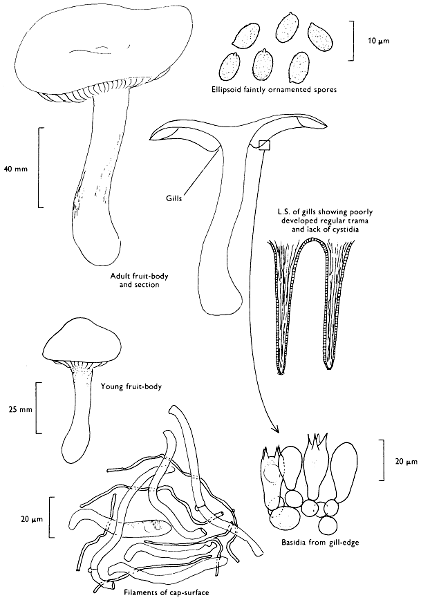
- Cap-surface composed of filamentous cells
Galerina
- 15. Gills free of the stem and the whole fruit-body very fragile
Bolbitius
- Gills attached to and running down the stem (decurrent),
easily separable from the cap-tissue and frequently veined at apex of stem
Paxillus
- 16. Cap scaly, fibrillose and roughened
Inocybe
- Cap smooth, greasy or viscid
17
- 17. Cap-surface composed of rounded cells
Agrocybe
- Cap-surface composed of filamentous cells
Naucoria & Hebeloma
- 18. Gills or complete fruit-body becoming liquefied
Coprinus
- Neither the gills nor fruit-body collapsing into a slurry of cells
19
- 19. Gills free to remote from the stem or attached and descending down the stem (decurrent)
20
- Gills attached in some way to the stem but not descending down the stem (adnate to adnexed)
21
- 20. Gills decurrent; stem possessing a cobweb-like veil
Gomphidius and Chroogomphus
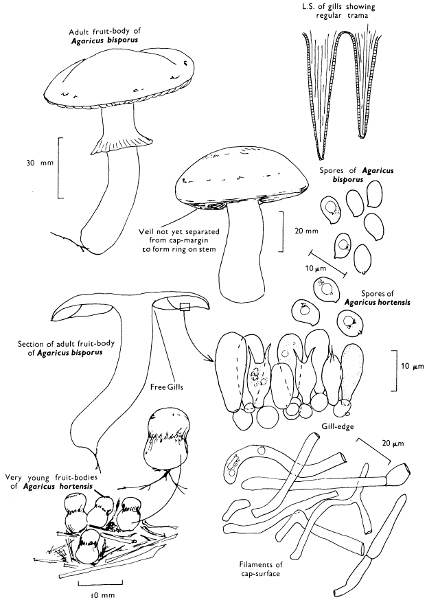
- Gills remote or free; stem possessing a usually persistent ring
Agaricus
- 21. Gills distinctly spotted or distinctly mottled; stem stiff but breaking with a snap when bent;
growing on dung or in richly manured areas
Panaeolus
- Gills not spotted or distinctly mottled; stem cartilaginous or not, and fruit-body growing on dung or not
22
- 22. Gills broadly attached to the stem (adnate) and with a veil girdling the stem
Stropharia
- Gills narrowly attached to the stem (adnexed) or with concave dentation near the stem (sinuate),
or if adnate then lacking a ring
23
- 23. Gills with concave indentation near the stem (sinuate) and cap and stem with a
cobweb-like veil
Hypholoma
- Gills attached to the stem but lacking a distinct concave indentation near the stem
24
- 24. Stem stiff but breaking with a snap when bent; edge of cap incurved at first and cap-surface
composed of filamentous cells
Psilocybe
- Stem fragile; edge of cap straight even when young and cap-surface composed of rounded cells
Psathyrella
- 25. Fruit-body fleshy and readily decaying, often firm but never tough
26
- Fruit-body tough and not easily decaying
47
- 26. Parasitic on other agarics
Nyctalis
- Not parasitic on other agarics
27
- 27. Spore-bearing layer on fold-like often forked gills or simply on irregularities
28
- Spore-bearing layer (hymenium), on distinct well-formed gills
29
- 28. Spore-bearing layer on fold-like gills
Cantharellus
- Spore-bearing layer on surface of irregularities
Craterellus
- 29. Cap easily separable from the stem
30
- Cap not easily separable from the stem
31
- 30. Stem with girdling veil (ring) and/or with a persistent cup-like structure at the base (volva);
cap usually with warts or scales distributed on its surface
Amanita
- Stem with a ring but lacking a volva; cap surface powdery, hairy or scaly
Lepiota & related genera
- 31. Cap, stem and gills brittle; stem never stiff and either exuding a milk-like juice or not;
spores with spines or warts which stain blue-black in solutions containing iodine
32
- Cap, stem and gills soft or if stem stiff then snapping when bent; gills never brittle
33
- 32. Fruit-body exuding a milk-like fluid
Lactarius
- Fruit-body not exuding milk-like fluid
Russula
- 33. Gills thick, watery and lustrous (waxy) or with a bloom as if powdered with talc; often brightly coloured
34
- Gills not waxy and rarely over 1·5 mm thick
36
- 34. Gills rather watery and lustrous (waxy); spores smooth
35
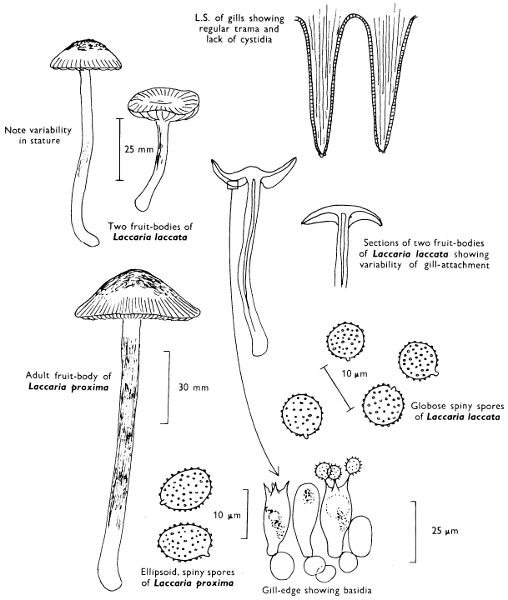
- Gills rigid not watery, with powdery bloom; spores with distinct spines
Laccaria
- 35. Fruit-body with a distinct veil and growing in woods; cap often viscid or pale
coloured
Hygrophorus
- Fruit-body lacking a veil and usually growing in fields; cap usually brightly coloured and sometimes viscid
Hygrocybe
- 36. Stem with girdling veil (ring) and/or stem not attached to the centre of the cap (eccentric)
37
- Stem central and lacking a ring
38
- 37. Stem central and possessing a ring
Armillaria
- Stem not centrally attached to the cap
members of the ‘Pleurotaceae’ (p. 74)
- 38. Stem fibrous
39
- Stem stiff only in the outer layers
42
- 39. Gills with a concave indentation near the stem (sinuate)
40
- Gills attached to and descending down the stem (decurrent)
41
- 40. Spores with warts which darken in solutions containing iodine
Melanoleuca
- Spores not so colouring in solutions containing iodine
Tricholoma & related genera
- 41. Spores with warts which darken in solutions containing iodine
Leucopaxillus
- Spores not so colouring in solutions containing iodine
Tricholoma & related genera
- 42. Gills thick and with rather blunt edges
Cantharellula & Hygrophoropsis
- Gills thin and with distinct and sharp edges
43
- 43. Gills attached to and descending down the stem (decurrent); cap often depressed at the centre and
sterile cells absent from the gills and the surface of the cap
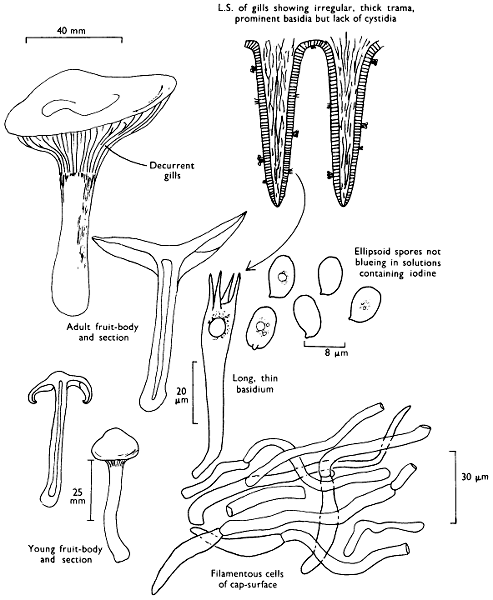
Clitocybe & Omphalina
- Gills attached to the stem but not descending down the stem (adnate to adnexed) or if descending
then distinct sterile cells on the gills, cap and stem
44
- 44. Cap-edge straight and usually striate when young; cap thin and somewhat conical and gills descending
down the stem or not
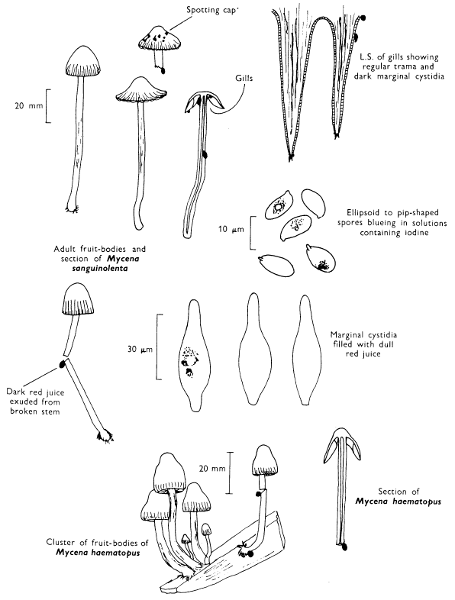
Mycena & related genera
- Cap-edge incurved, non-striate and cap rather fleshy; gills not descending down the stem
45
- 45. Stem dark and woolly at least in the lower half and the cap viscid; fruit-bodies growing in clusters on tree-trunks
Flammulina
- Stem not dark and woolly
46
- 46. Cap viscid and stem usually rooting; fruit-body growing directly on wood or attached to
wood by long strands or cords of mycelium (rhizomorphs)
Oudemansiella
- If cap viscid then fruit-body neither attached to wood by cords of mycelium nor stem with a rooting base
Collybia & related genera
- 47. Stem central and gills often interconnected by veins; cap can be dried and later revived, purely by moistening
Marasmius & related genera
- Stem not attached to the centre of the cap and fruit-body although persistent not easily
revived to natural shape after once being dried
48
- 48. Spore-print blue-black with solutions containing iodine
49
- Spore-print yellowish in solutions containing iodine
50
- 49. Gills toothed or notched along the edges
Lentinellus
- Gills even along their edges and not toothed
Panellus
- 50. Gills appearing as if split down their middles
Schizophyllum
- Gills not splitting
51
- 51. Gills notched or toothed along their edges
Lentinus
- Gills even along their edges and not toothed
Panus
- 52. Spore print yellowish, purplish, black or pink
53
- Spore-print some shade of brown, but without purplish flush
56
- 53. Spore-print yellowish or pinkish
54
- Spore-print purplish brown or blackish
55
- 54. Spore-print yellowish
Gyroporus
- Spore-print pinkish
Tylopilus
- 55. Spore-print purplish brown
Porphyrellus
- Spore-print blackish and spores ornamented
Strobilomyces
- 56. Cap glutinous and stem with or without girdling veil (ring); within the tubes the sterile cells
(cystidia) cluster together
Suillus
- Cap at most viscid and then only in wet weather and sterile cells within the tubes individually placed
57
- 57. Stem-surface covered with distinct black or dark brown or white then darkening scales; spore-print
clay-brown with or without a flush of cinnamon-pinkish brown
Leccinum
- Stem-surface covered completely or in part with a network or pattern of faint lines or pale yellow
or red-rust but never black dots; spore-print olivaceous buff
Boletus & related genera
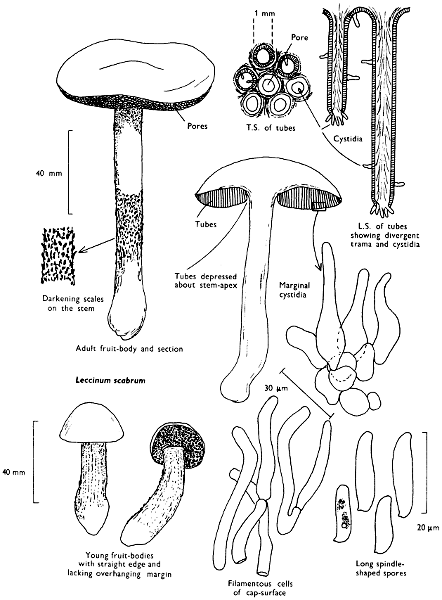
Leccinum scabrum (Fries) S. F. Gray
Birch rough stalks or Brown birch-bolete.
Cap: width 45-150 mm. Stem: length 70-200 mm; width 20-30 mm.
Description: Plate 1.
Cap: convex and becoming only slightly expanded at maturity, pale
brown, tan or buff, soft, surface dry, but in wet weather becoming
quite tacky, smooth or streaky-wrinkled and cap-margin not overhanging
the tubes.
Stem: white, buff or greyish, roughened by scurfy scales which are
minute, pale and arranged in irregular lines at the stem-apex, and
enlarged and dark brown to blackish towards the base.
Tubes: depressed about the stem, white becoming yellowish brown
at maturity, with small, white pores which become buff at maturity
and bruise distinctly yellow-brown or pale pinkish brown when
touched.
Flesh: watery, very soft in the cap lacking distinctive smell and either
not changing on exposure to the air or only faintly becoming pinkish
or pale peach-colour.
Spore-print: brown with flush of pinkish brown when freshly prepared.
Spores: very long, spindle-shaped, smooth, pale honey-coloured under
the microscope and more than 14 µm in length (14-20 µm long ×
5-6 µm broad).
Marginal cystidia: numerous and flask-shaped. Facial cystidia: sparse,
similar to marginal cystidia.
Habitat & Distribution: Found in copses and woods containing birch
trees, or even accompanying solitary birches.
General Information: This fungus is recognised by the pale brown cap,
the white, unchanging or hardly changing flesh and the cap-margin
not overhanging the tubes. There are several closely related fungi
which also grow with birch trees but they need some experience in
order to distinguish them. This fungus was formerly placed in the
genus Boletus, indeed it will be found in many books under this
name. Species of Leccinum are edible and considered delicacies in
continental Europe. The majority can be separated from the other
fleshy fungi with pores beneath the cap, i.e. boletes, by the black
to brown scaly stem and rather long, elongate spores. The scales
on the stem give rise to the common name ‘Rough stalks’ which is
applied to this whole group of fungi.
Illustrations: F 39C; Hvass 253; LH 122; NB 1556; WD 891.
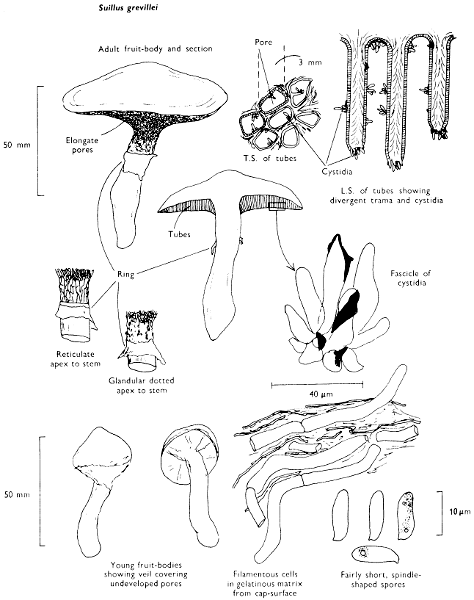
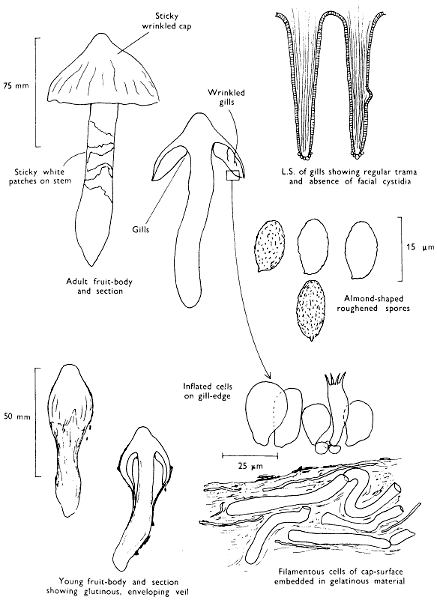
Suillus grevillei (Klotzsch) Singer
Larch-bolete
Cap: width 30-100 mm. Stem: width 15-20 mm; length 50-70 mm.
Description: Plate 2.
Cap: convex or umbonate at first, later expanding and then becoming
plano-convex, golden-yellow or rich orange-brown, very slimy
because of the presence of a pale yellow sticky fluid.
Stem: apex reddish and dotted or ornamented with a fine network,
cream-coloured about the centre because of the presence of a ring
which soon collapses, ultimately appearing only as a pale yellow
zone; below the ring the stem is yellowish or rusty brown, particularly
when roughly handled.
Tubes: adnate to decurrent, deep yellow but becoming flushed wine-coloured
on exposure to the air, with angular and small sulphur-yellow
pores which become pale pinkish brown to lilaceous or
pale wine-coloured when handled.
Flesh: with no distinctive smell, pale yellow immediately flushing
lilaceous when exposed to the air, but finally becoming dingy red-brown,
sometimes blue or green in the stem-base.
Spore-print: brown with distinct yellowish tint when freshly prepared.
Spores: long, ellipsoid, smooth and pale honey when under the microscope,
less than 12 µm in length (8-11 µm long × 3-4 µm broad).
Marginal cystidia: in bundles and encrusted with amorphous brown,
oily material. Facial cystidia: similar in shape and morphology to
marginal cystidia.
Habitat & Distribution: Found on the ground accompanying larch
trees either singly or more often in rings or troops.
General Information: This fungus is easily recognised by the poorly
developed ring, overall golden-yellow colour and pale yellow viscidness
on the cap which comes off on to the fingers when the fruit-body
is handled. There are several closely related fungi which also
grow with coniferous trees, e.g. Suillus luteus Fries, ‘Slippery jack’,
but many need experience in order to identify them. All these fungi
were formerly placed in the genus Boletus, because of the fleshy
fruit-body with pores beneath the cap. The larch-bolete receives its
common name from the close relationship of the fungus with the
larch. On drying S. luteus and S. grevillei may strongly resemble
one another but the former can be distinguished when fresh by the
chocolate brown, sepia, or purplish brown cap and the large whitish,
lilac-tinted ring.
Species of Suillus are edible and rank highly in continental cook-books,
although they have disagreeably gelatinous-slimy caps, a
character, in fact, which helps to separate them from other fleshy
pore-fungi.
Illustrations: F 41a; Hvass 257; ML 187; NB 1044; WD 842.
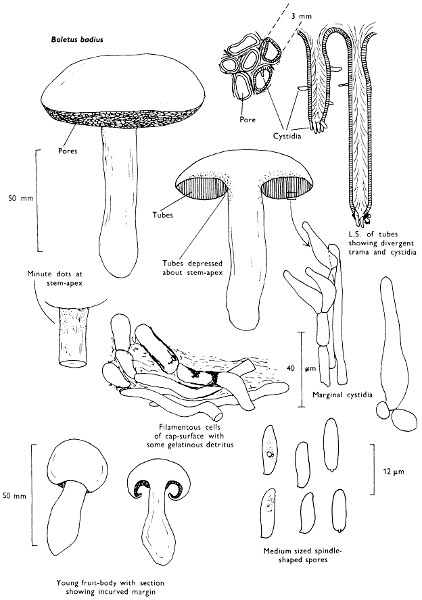
Boletus badius Fries
Bay-coloured bolete
Cap: width 70-130 mm. Stem: width 34-37 mm; length 110-125 mm.
(36-40 mm at base).
Description: Plate 3.
Cap: hemispherical, minutely velvety, but soon becoming smooth and
distinctly viscid in wet weather, red-brown flushed with date-brown
and darkening even more with age and in moist weather to become
bay-brown.
Stem: similarly coloured to the cap but paler particularly at the apex,
smooth or with faint, longitudinal furrows which are often powdered
with minute, dark brown dots.
Tubes: adnate or depressed about the stem, lemon-yellow but immediately
blue-green when exposed to the air and with angular, rather
large similarly coloured, pores which equally rapidly turn blue-green
when touched.
Flesh: strongly smelling earthy, pale yellow but becoming pinkish in
centre of the cap, and blue in the stem and above the tubes when
exposed to the air, but finally becoming dirty yellow throughout.
Spore-print: brown with a distinct olivaceous flush.
Spores: long, spindle-shaped, smooth, honey-coloured under the
microscope and greater than 12 µm in length (13-15 µm long ×
5 µm broad).
Marginal cystidia: numerous, flask-shaped and slightly yellowish.
Facial cystidia: scattered and infrequent and similar to marginal
cystidia in shape.
Habitat & Distribution: Found in woods, especially accompanying pine
trees, but often found fruiting on the site of former coniferous trees,
even years after the trunks or the stumps have been removed.
General Information: This fungus is recognised by the rounded, red-brown
cap, coupled with the pale yellow flesh and greenish yellow
tubes, both of which become greenish blue when exposed to the air.
There are several species in the genus Boletus which stain blue at
the slightest touch or when the flesh is exposed to the air, e.g.
B. erythropus (Fries) Secretan, a common bolete with a dark olivaceous
cap, orange pores and red-dotted stem.
The flesh of some species of Boletus, e.g. B. edulis Fries, however,
remains unchanged or at most becomes flushed slightly pinkish.
Although many people say they recognise B. edulis, the ‘Penny-bun’
bolete—a name derived from the colour of the cap, there is some
doubt as to whether the true B. edulis is common in Britain as we
are led to believe. B. edulis and its relatives are highly recommended
as edible (see p. 35). B. badius is also edible, but it is ill-advised to
eat any bolete which turns blue when cut open.
Illustrations: B. badius—F 38c; Hvass 248 (not very good); LH 191;
NB 1095; WD 851. B. edulis: F 42a; Hvass 246; LH 191; NB 1433.
General notes on Boletes
There are nearly seventy boletes recorded for the British Isles and
evidence of others which have as yet not been fully documented. As a
group they are characterised by being fleshy, possessing a central stem
and producing their spores within the tubes, and not on gills as in the
common mushroom. It is the first character by which the boletes
differ so markedly from the other pored fungi, such as the ‘Scaly
Polypore’ (see p. 140).
The boletes have long been classified in the genus Boletus, but
instead of referring all the pored, fleshy fungi to a single large genus
several genera are now recognised. The separation of these genera is
based on differences in colour of the spore-print and differences in the
anatomy of the tubes, cap and stem, etc., e.g. members of the genus
Suillus have colourless or pale coloured dots on the stem exuding a
resin-like liquid in wet weather, which is clear and glistening in some
species but turbid and whitish in others, gradually darkening and
hardening so that the stem is ultimately covered in dark brown or
reddish smears or spots; members of the genus Leccinum on the other
hand never exude liquid and have coarse or fine roughenings on the
stem which are usually dark, but may commence white and ultimately
darken depending on the species; many species of Boletus possess a
very distinct raised network all over the stem, whilst others have it
present only in part, or have minute, often brightly coloured, dots
replacing it.
Within this single, yet not particularly large, group of fungi, several
biological phenomena are demonstrable. There is good evidence that
the majority of British boletes are mycorrhizal; several species are
known to be associated only with one species of tree or group of closely
related tree-species. Thus Suillus grevillei and S. aeruginascens (Secretan)
Singer grow in association with larch trees; S. luteus and Boletus
badius in contrast grow in association with pine trees; Leccinum
scabrum with birch trees; L. aurantiacum (Fries) S. F. Gray, with
poplar trees and L. quercinum (Pilát) Green & Watling, with oak trees.
Boletus edulis can be separated into several distinct subspecies which
are associated with different trees; the two commonest subspecies are
those associated with birch and with beech trees. It is well known that
although present in this country during the warmer periods of the
Ice-Age, larch neither survived the intense cold of the last advance of
the ice nor migrated back into Britain after the ice had melted. Thus
all larches which we see in Britain have been planted by man. There
is little doubt that mycelia of many fungi were introduced along with
these plants very probably including the mycelium of the larch-bolete.
A similar pattern can be seen with other introduced trees, although not
to such a marked degree, e.g. spruce trees. The beech tree, however,
is native to the south of England, unlike the larch returning to this
country after the ice had melted; it has been planted extensively
outside its former range in northern areas of the British Isles taking
with it its associated fungi. There is some evidence that some stocks
of beech and fungi have been introduced from continental Europe in
comparatively recent times.
A parallel, yet inexplicable association is found between the bolete
Suillus bovinus (Fries) O. Kuntze and its close relative Gomphidius
roseus (Fries) Karsten where the mycelium of two fungi are found intertwined
forming a close association! Parasitism although rare is also
found amongst the boletes, and an uncommon parasitism at that—a
fungus on a fungus; for example in Britain although infrequent Boletus
parasiticus Fries grows attached and ultimately replaces the spore-tissue
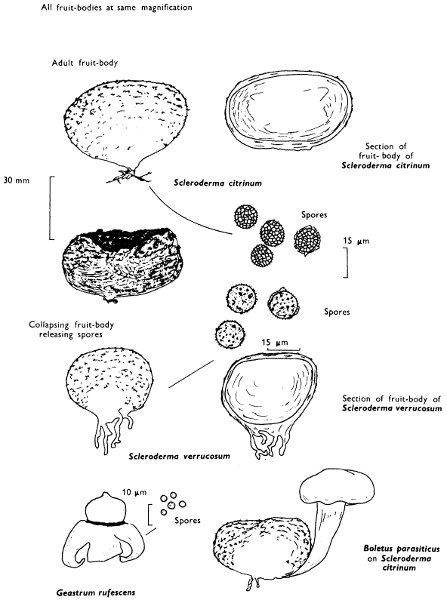
of the common earth-ball (Scleroderma, see p. 192).
Those fungi which grow on dead and decaying substrates are called
saprophytes and although the greater number of higher fungi would
be included in this class of organisms the character is infrequent
amongst the boletes. One British example of this type of fungus is
the rare Boletus sphaerocephalus Barla which grows on woody debris.
Chemists have long been interested in boletes, for as noted above the
flesh of some species when exposed to the atmosphere turns vivid
colours, a feature often incorporated into the Latin name, e.g. Boletus
purpureus Persoon, from the purple colours produced whenever the
fruit-body is handled. The reaction appears to be an oxidation where
in the presence of an enzyme and oxygen a pigmented substance or
substances are produced. What the significance of these colour-changes
is in nature is as yet unknown; however, what is interesting is that
many of the chemicals involved are unique and have only recently
been analysed completely; they are related to the quinones.
There is little doubt that it is this rapid and intense blueing of the
flesh of many boletes that has lead to a belief that they are poisonous.
It is uncertain whether there are any truly toxic species of Boletus
but several have unpleasant smells and tastes which make them very
unattractive. Boletus edulis is the important ingredient, however, which
gives the distinctive taste to so-called dried mushroom soup. Thousands
of fruit-bodies are collected annually in the forests of Europe to
be later dried and processed for incorporation into soup. Boletes
appear to form an important part of the diet of several rodents and
deer and in Scandinavia in the diet of reindeer.
Probably one of the most obscure of our British boletes is Strobilomyces
floccopus (Fries) Karsten, the ‘Old Man of the Woods’. It has a
black, white and grey woolly, scaly cap and stem, and the flesh distinctly
reddens when exposed to the air. The spores are almost spherical,
purple-black in colour and covered in a coarse network when seen
under the microscope. All these characters readily separate Strobilomyces
from all other European boletes; however, in Australasia, members
of this and related genera form a very important part of the flora.
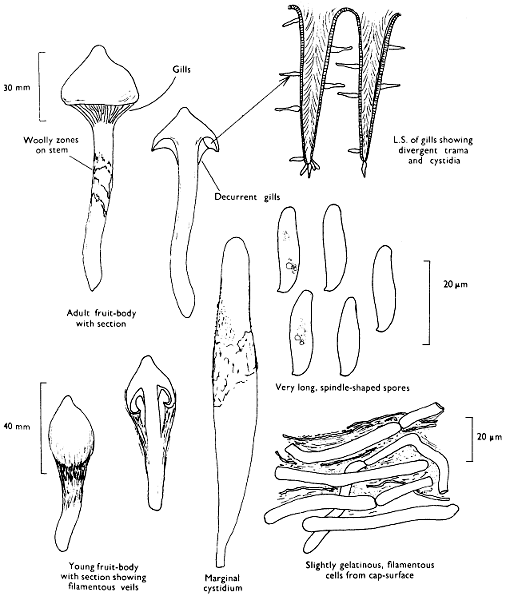
Chroogomphus rutilus (Fries) O. K. Miller
Pine spike-cap
Cap: width 30-150 mm. Stem: width 10-18 mm; length 60-120 mm.
Description:
Cap: convex with a pronounced often sharp umbo, wine-coloured,
flushed with bronze-colour at centre and yellow or ochre at
margin, viscid but soon drying and then becoming paler and quite
shiny.
Stem: yellowish orange, apricot-coloured or peach-coloured, streaked
with dull wine-colour, spindle-shaped or narrowed gradually to the
apex from a more or less pointed base.
Gills: arcuate-decurrent, distant, at first greyish sepia then dingy
purplish with paler margin, but finally entirely dark purplish brown.
Flesh: lacking distinctive smell and reddish yellow or pale tan in the
cap, rich apricot- or peach-colour towards the stem-base.
Spore-print: purplish black.
Spores: very long, spindle-shaped, smooth, olivaceous purple and
greater than 20 µm in length (20-23 × 6-7 µm).
Marginal cystidia: cylindrical to lance-shaped and up to 100 × 15 µm.
Facial cystidia: similar to marginal cystidia.
Habitat & Distribution: Found in pine woods, usually solitary or in
small groups. Fairly common throughout the British Isles and
characteristic of Scots Pine woods.
General Information: This fungus can be distinguished by the purplish
or wine-coloured cap and the gills being pigmented from youth.
There is only one other British species of this genus, i.e. C. corallinus
Miller & Watling.
Chroogomphus is separated from Gomphidius by the flesh having
an intense blue-black reaction when placed in solutions containing
iodine, and the gills being coloured from their youth. In many
books Chroogomphus is placed in synonymy with the genus Gomphidius.
However, Gomphidius glutinosus (Fries) Fries, G. roseus (Fries)
Karsten and G. maculatus Fries all have whitish gills when immature
which gradually darken, and their flesh simply turns orange-brown
in solutions of iodine. G. glutinosus is uniformly grey in colour and
is most frequently found under spruce and other introduced conifers:
G. roseus has a pale-pinkish coloured cap and white stem, and grows
with pine; G. maculatus grows under larch and is flushed lilaceous
at first but becomes strongly spotted with brown when handled.
Illustrations: Hvass 192; LH 213; WD 833.
Paxillus involutus (Fries) Karsten
Brown roll-rim
Cap: width 50-120 mm. Stem: width 8-15 mm; height 30-75 mm.
Description:
Cap: at first convex with a strongly inrolled, downy margin, but then
expanded and later frequently depressed towards the centre, clay-coloured,
ochre or yellow-rust, slightly velvety but becoming smooth
or sticky particularly in wet weather and readily bruising red-brown
when fresh.
Stem: central or slightly eccentric, thickened upwards, fibrillose-silky,
similarly coloured to the cap but typically streaked with red-brown
particularly with age.
Gills: ochre or yellow-brown then rust and finally darker brown,
decurrent, crowded, often branched and united about the apex of
the stem; easily peeled from the flesh with the fingers and rapidly
becoming red-brown on handling.
Flesh: thick, soft and with slightly astringent smell and yellowish to
brownish but becoming red-brown after exposure to the air.
Spore-print: rust-brown.
Spores: medium-sized, ellipsoid, smooth, deep yellow-brown and
rarely greater than 10 µm in length (8-10 × 5-6 µm).
Marginal cystidia: numerous lance-shaped or spindle-shaped.
Facial cystidia: scattered and similar in shape to marginal cystidia.
Habitat & Distribution: Found on heaths and in mixed woods, particularly
where birch has or is now growing, or even accompanying
solitary birch trees.
General Information: This fungus is easily recognisable by the strongly
inrolled, woolly margin of the cap and yellow-brown gills which
are easily separable from the cap-flesh. P. rubicundulus P. D. Orton
is similar but grows under alder and has yellow gills unchanging when
handled and dark scales on the cap. P. atrotomentosus (Fries) Fries
and P. panuoides (Fries) Fries both grow on coniferous wood and
have smaller spores; the former is recognised by the dark brown to
almost black shaggy stem and the latter by the shell-shaped cap
devoid almost completely of a stem.
Illustrations: F 41c; Hvass 189; LH 185; NB 1158; WD 702.
Cortinarius pseudosalor J. Lange
Cap: width 60-125 mm. Stem: width 15-25 mm; length up to 180 mm.
Description:
Cap: bell-shaped or bluntly conical only slightly expanding with
maturity, smooth or wrinkled at centre but often furrowed at the
margin, slimy, brown with a distinct olive flush when in fresh
condition and becoming ochraceous brown and shiny when dry.
Stem: usually swollen to some degree about the middle, slimy particularly
towards the base, whitish throughout when young except
for a faint amethyst or violaceous flush in the lower part; as the
slime dries the stem becomes shiny and the outer surface breaks
up into fibrillose scales or scaly, irregular ring-zones.
Flesh: lacking distinct smell, white with ochraceous flush in the cap,
white in the stem, thick and soft in the cap but fibrous in the stem.
Gills: adnate, broad, rather thick, frequently veined and distant,
ochraceous brown and finally deep rust-brown.
Spore-print: rust-colour.
Spores: long, slightly almond-shaped in side view, finely warted
throughout and not less than 12 µm in length (13-14 × 7-8 µm).
Marginal cystidia: ellipsoid or club-shaped, hardly different from the
surrounding undeveloped basidia.
Facial cystidia: absent.
Habitat & Distribution: Found on the ground in copses and woods
especially those containing beech.
General Information: Recognised by the conical, grooved cap and the
slimy spindle-shaped stem with a distinct violaceous flush; this
fungus is often misnamed C. elatior Fries but this is a much less
common fungus. There are several closely related fungi, but these
grow with other tree-species and need much more experience to
distinguish one from the other. C. pinicola P. D. Orton is one such
species growing in the litter under Pinus sylvestris, Scots Pine; this
species is fairly common in the remnant pine woods of Northern
Scotland. The large size, sticky or glutinous cap and stem indicate
that this fungus belongs to Cortinarius, subgenus Myxacium.
Illustrations: Hvass 145; LH 162; NB 119; WD 601.
General notes on Cortinarii
The genus Cortinarius is the largest genus of agarics in the British Isles,
indeed in Europe and North America—perhaps in the world. It includes
some of our most beautiful agarics, yet it is one of the least
satisfying to the mycologist because of the difficulties experienced in
identifying collections—partly because many species are so seldom
seen.
Cortinarius contains just under two hundred and fifty recognisable
British species, although recent research has shown that many more
are yet to be described from this country as new to science. Except for
some very characteristic species the individual members within the
genus Cortinarius are often very difficult to separate one from the other;
however, Cortinarius is one of our least difficult genera to recognise in
the field owing to the presence when mature of rust-coloured gills
and a cobwebby veil which extends from the margin of the cap to the
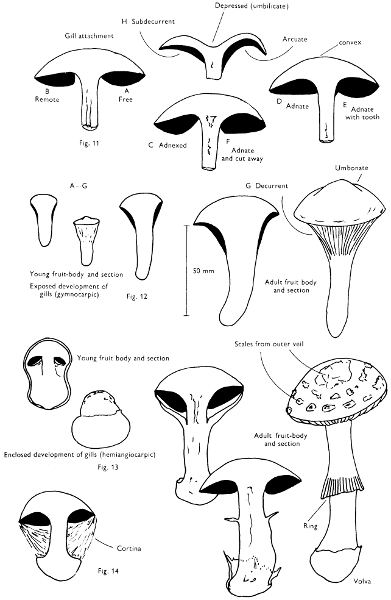
stem. This structure is termed a cortina (Fig. 14) and in young specimens
covers the gills with delicate filaments. As the cap expands the cottony
or cobwebby filaments are stretched and either disappear entirely or
may collapse to form a ring-like zone of filaments on the stem. In
some species a second completely enveloping veil is also found, and this
veil is viscid in one distinct group of which C. pseudosalor already
described is a member. The gills in the genus are variable in colour
when young although constant for a single species; they may be
lilaceous purple, orange, brown, red, yellow-ochraceous or tan, but
ultimately in all members at maturity they become rust-colour. The
spores under the microscope are richly coloured, yellow to red-brown
and are frequently strongly warted; in mass they are rust-brown
and this character coupled with the presence of the cobweb-like veil
characterises the genus.
Within the genus Cortinarius there is a wide range of characters
varying from species with distinctly sticky caps and stems, some with
sticky caps and dry stems to those with both dry caps and stems. A
few species are very large and fleshy whilst others are quite slender and
many of the latter rapidly change colour on drying out and are then
said to be hygrophanous. However, although there is such a large
spectrum of characters in a single genus the species all have in common
the cortina and rust-coloured gills, the latter often appearing as if
powdered with rusty dust.
Utilising the characters mentioned above this very large genus can
be split into the following six sections, called by the mycologist subgenera:
- Large to medium sized fleshy agarics with viscid caps and stems—Myxacium
- Large, fleshy agarics with viscid or tacky caps when fresh but dry
stems—Phlegmacium
- Large to medium sized agarics with dry, scaly or humid caps and
dry stems which if orange tawny are robust—Cortinarius
- Medium, rarely large, agarics with dry, silky to innately fibrillose
caps, slender stems and frequently with at least part of the fruit-body
yellow, orange or reddish—Dermocybe
- Medium to small agarics with silky fibrillose, non-hygrophanous
caps which may become tacky in wet weather and then usually
with robust, clavate-bulbous stems—Sericeocybe
- Small, less frequently medium or large agarics, all with distinctly
hygrophanous caps—Hydrocybe.
In several continental books some or all of these divisions are recognised
as distinct genera in their own right. The subgenus Telamonia
which occurs in many texts was formerly thought to differ from
Hydrocybe in the presence of a universal veil; the universal veil is a
second veil which completely envelopes the fruit-body when it is
young and is in addition to the cortina. However, the modern treatment
would seem to suggest that the presence of the universal veil is not of
the utmost importance and so the two subgenera are incorporated into
one. The name Hydrocybe reflects the character of changing colour
as it dries out because of the loss of water. Within each subgenus
the species are distinguished by the colour of the young gills and of
the cap, the veil colour and texture, and microscopic characters of the
spores, particularly their size.
The majority of species of Cortinarius are mycorrhizal and like the
boletes possess very specific relationships with tree species. Thus some
are typical of coniferous woodland and others typical of deciduous
woodland in general, whilst others typify woods of a particular tree,
e.g. beech, oak, birch, pine, larch. Some species are characteristic of
woods on limestone or chalky soils (calcareous) whilst others are
characteristic of woods on sandy, heathy acidic soils. For example,
Cortinarius armillatus (Fries) Fries which is found in damp woods and
possesses one or more cinnabar-red or scarlet zones on the stem and
red fibrils at the stem-base appears to be connected with birch. Several
species are associated with native trees whilst others have undoubtedly
been introduced from abroad. They are very important in the economy
of the woodland ecosystem.
One of the most beautiful and easily distinguished of our British
species is Cortinarius violaceus (Fries) Fries which has uniformly deep
violet-coloured stem and cap and coloured cystidia on the gill-margin,
a character unusual in Cortinarius.
No species are known to be truly poisonous and many species are
known to be edible, but many are too small to be of any value. Some of
the larger species are regarded as good to eat, but frequently are too
scarce. Thus the necessity for experience to recognise the different
species, coupled with their often unpleasant tastes make them an
unimportant group of agarics for eating.
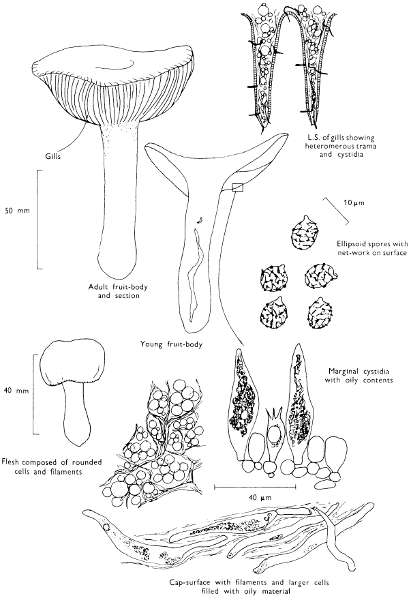
Russula ochroleuca (Secretan) Fries
Common yellow russula
Cap: width 50-100 mm. Stem: width 20-35 mm; length 50-100 mm.
Description: Plate 7.
Cap: yellow-ochre or dull yellow becoming paler with age, or flushed
faintly greyish green, convex but soon expanding and becoming
flat or depressed in the centre, smooth, or granular when young and
slightly tacky in wet weather, faintly striate at the margin.
Stem: white at first then flushed slightly greyish, smooth or wrinkled,
firm at first but quickly becoming soft and fragile.
Flesh: brittle, firm at first then soft, white, yellow under cap-centre.
Gills: white at first then flushed pale cream-colour, brittle, adnexed
to free, rather distant.
Spore-print: faintly cream when freshly prepared.
Spores: medium-sized, hyaline, broadly ellipsoid or subglobose to
almost globose, coarsely ornamented with prominent warts which
stain blue-black when mounted in solutions containing iodine and
which are faintly interconnected by low ridges, about 8 × 7 µm in
size (9-10 × 7-8 µm).
Marginal cystidia: prominent, lance- to spindle-shaped and often filled
with oily material.
Facial cystidia: similar in shape to marginal cystidia and projecting
some distance from the gill-face.
Habitat & Distribution: Commonly found in mixed woods from summer
until late autumn.
General Information: Easily recognised by the ochre-yellow cap, very
pale cream-coloured spore-print and greying stem. Two other
yellow-capped species of Russula are commonly found. R. claroflava
Grove with yellow spore-print and blackening fruit-body which grows
with birches in boggy places, and R. lutea (Fries) S. F. Gray which is
much smaller, having a cap up to 50 mm and very deep egg-yellow
gills and spore-print; it grows in deciduous woods.
Illustrations: F 22a; Hvass 226; LH 119; NB 1371; WD 491.
General notes on the genus Russula
A large genus with nearly one hundred distinct species in the British
Isles and several others yet unrecognised or undocumented. This genus
is composed generally of large toadstools often beautifully coloured,
indeed the majority have brightly coloured caps in reds, purples,
yellows or greens depending on the species although a few are predominantly
white bruising reddish brown or grey to some degree.
Such large and distinctive fungi one would think would be the
easiest members of our flora to identify, unfortunately they are not.
They form a group quite isolated in their relations, the only close
relatives being members of the genus Lactarius, to be dealt with later
(see p. 50). The flesh of members of both Lactarius and Russula
contains groups of rounded cells, a feature unique amongst agarics
and explains why in Russula the fruit-bodies, cap and gills and sometimes
the stem are brittle and easily break if crushed between the
fingers. The fruit-body does not exude a milky liquid when the flesh
is broken.
The spore-print varies, depending on the species involved, from white
to deep ochre and individual spores are covered in a coarse ornamentation
which is composed of isolated warts or warts interconnected by
raised lines, or mixtures of both. The ornamentation stains deep blue-black
when the spores are mounted in solutions containing iodine and
the pattern which is produced appears in many cases to be of a specific
character.
The majority of the species, if not all north-temperate species are
mycorrhizal and the familiar host-tree fungus relationship can be
recognised:—
R. claroflava Grove, with birch in boggy places, R. emetica (Fries)
S. F. Gray with pine in wet places, R. betularum Hora with birch in
grassy copses and R. sardonia Fries with pines. Brief notes are here
included giving the basic characters of eight common species, but it
must be appreciated the identification of many species within this
genus is difficult.
R. atropurpurea (Krombholz) Britz.
Blackish purple russula
Cap: width 50-100 mm. Stem: width 14-25 mm; length 60-80 mm.
Cap: deep reddish purple but becoming spotted with either cream-colour
or white blotches.
Stem: white but becoming flushed greyish or stained brownish with age.
Gills: white then very pale yellow.
Flesh: white in cap and stem.
Spore-print: white.
On the ground in mixed woods and copses, particularly those containing
oak.
Russula cyanoxantha (Secretan) Fries
Cap: width 50-150 mm. Stem: width 10-30 mm; length 50-100 mm.
Cap: lilac, bluish to purple often with green tints.
Stem: pure white.
Gills: pure white.
Flesh: white.
Spore-print: white.
Common in deciduous woods, especially beech-woods.
R. emetica (Fries) S. F. Gray
Emetic russula
Cap: width 50-100 mm. Stem: width 8-15 mm; length 25-70 mm.
Cap: bright scarlet fading with age to become spotted pinkish, slightly
viscid when moist.
Stem: spongy, fragile.
Flesh: white.
Gills: pure white.
Spore-print: pure white.
In pine woods usually in boggy areas.
R. fellea (Fries) Fries
Geranium-scented russula
Cap: width 40-75 mm. Stem: width 10-20 mm; length 30-75 mm.
Cap: tacky when fresh, straw-coloured or pale tawny brown.
Stem: similarly coloured to the cap.
Gills and flesh: pale straw-colour and smelling of House Geraniums
(i.e. Pelargoniums).
Spore-print: cream-coloured.
Common under beech.
R. foetens (Fries) Fries
Foetid russula
Cap: width 70-170 mm. Stem: width 15-30 mm; length 50-90 mm.
Cap: slimy, dingy yellow to tawny, margin strongly furrowed and
ornamented with raised bumps.
Stem: whitish then flushed or spotted with rust-brown.
Gills: straw-coloured, often spotted brown with age and beaded with
watery droplets when growing under moist conditions.
Flesh: white to cream, brittle and with foetid-oily smell.
Spore-print: pale cream-colour.
Common in deciduous woods.
R. mairei Singer
Cap: width 30-75 mm. Stem: width 7-15 mm; length 35-70 mm.
Cap: scarlet red but developing creamy areas with age, dry.
Stem and gills: white but with a distinct although faint greenish grey
flush, the former fairly firm.
Flesh: white.
Spore-print: pure white.
Commonly accompanying beech, even individual trees in gardens.
R. nigricans (Mérat) Fries
Blackening russula
Cap: width 75-200 mm. Stem: width 15-35 mm; length 25-75 mm.
Cap: cream-coloured then flushed sooty brown, finally black as if
scorched by proximity to bonfire.
Stem: white then dark brown.
Gills: pale ochre reddening when bruised, thick and very distant.
Flesh: white slowly dull red on cutting then brown and finally changing
soot-colour after some time.
Spore-print: white.
Common in deciduous woods.
R. xerampelina (Secretan) Fries
Cap: width 50-140 mm. Stem: width 15-30 mm; length 40-60 mm.
Cap: deep blood-red or brownish red.
Stem: white with a flush of red towards the base.
Gills: cream then ochraceous.
Flesh: white staining brownish and smelling strongly of fish- or crab-paste,
and staining dark green when a crystal of green iron sulphate
is rubbed into it.
Spore-print: deep cream-colour.
Common in mixed woods; a very variable fungus with many colour-forms,
but easily recognised by the green reaction with ferrous
sulphate.
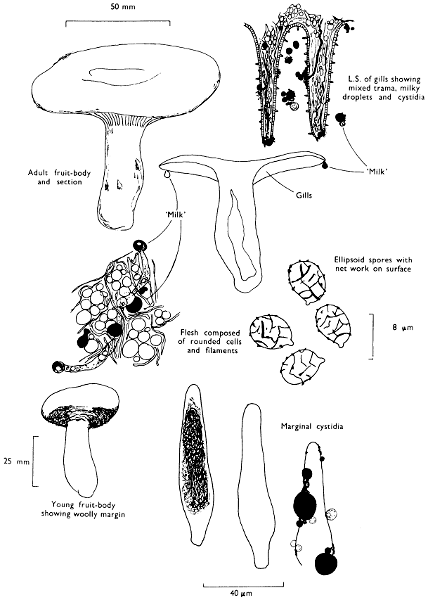
Lactarius turpis (Weinm.) Fries
Ugly milk-cap
Cap: width 60-200 mm. Stem: width 10-25 mm; length 40-75 mm.
Description:
Cap: firm, convex usually with a central depression at maturity, dark
olive-brown or dark greyish olive with a yellow-tawny, woolly margin
when young which soon disappears, and the whole cap becomes
sticky with age and turns deep purple when a drop of household
ammonia is placed on it.
Stem: short, stout, similarly coloured to the cap except for the distinctly
ochraceous apex, slimy and pitted.
Gills: crowded, cream-coloured to pale straw-coloured, but soon
spotted with dirty brown, particularly when bruised.
Flesh: white or greyish ochre exuding a milk-like liquid which lacks
a distinct smell and is white and unchanging when exposed to the air.
Spore-print: pale pinkish buff.
Spores: subglobose or ellipsoid and covered in a network of strongly
developed, raised lines interconnected by finer ones, both of which
stain blue-black in solutions containing iodine, generally 8 × 6 µm
in size (7-8 × 6-7 µm).
Marginal cystidia: lance- or spindle-shaped and filled with oily contents.
Facial cystidia: similar to marginal cystidia.
Habitat & Distribution: Common in woods and copses, or on heaths
especially in boggy places but always where birch is growing.
General Information: Easily recognised by the dull colours and purple
reaction with alkali; there is no British species with which L. turpis
can be mistaken. The purple reaction is similar to that found in the
familiar school laboratory reagent litmus, for the compound found
in L. turpis turns purple in alkali and reddens in acidic solutions. First
discovered by Harley in 1893 this reaction marked the beginning
of a whole series of chemical studies on the agarics which has led
to the discovery of many unique compounds.
Illustrations: Hvass 214 (but too green); LH 213; NB 1133; WD 381.
General notes on the genus Lactarius
There is little doubt that the genus Russula and the genus Lactarius
are closely related; in fact they stand aside from the other agarics in
the very important character mentioned on page 46. In Europe the
easiest distinction between the two genera is that members of the
genus Lactarius exude a milk-like juice which may be white or variously
coloured depending on the species involved (e.g. purple in L. uvidus
(Fries) Fries, yellow in L. chrysorheus Fries). The cap, stem and
frequently the gills are brittle and when broken liberate the milk-like
liquid; when the fruit-body is dry, however, the presence of this liquid
may be difficult to demonstrate. The spores have a blue-black ornamentation
under the microscope when mounted in iodine, and although
when in mass the colours are not as varied as those found in the genus
Russula there is every likelihood that they will play an important role
in the classification of the group in the future. The colour of the
spore-print has been rather neglected, although the genus includes
some rather unusual fungi.
The odours of many species are very distinct and vary from the smell
of coconut and spice to those of various flowers; an odour commonly
met with is termed ‘oily rancid resembling butter which has become
mouldy’; in early books it was described as being the smell of bed-bugs!
The majority of the species are undoubtedly mycorrhizal: thus L.
torminosus is found with birch, L. deliciosus and L. rufus with conifers
and L. quietus with oak. Brief notes are given on additional species:—
L. camphoratus (Fries) Fries
Curry-centred milk-cap
Cap: width 20-50 mm. Stem: length 20-50 mm; width 4-6 mm.
Cap and stem: red-brown.
Gills: reddish brown.
Flesh: reddish buff with an aromatic odour resembling spices which
becomes very strong when dried and exudes a pale thin milk-like
liquid.
Common in conifer woods and plantations.
L. deliciosus (Fries) S. F. Gray
Saffron milk-cap
Cap: width 50-120 mm. Stem: length 20-60 mm; width 15-25 mm.
Cap: viscid, dirty greyish ochre with flush of tawny but soon becoming
greenish with age.
Stem: dirty buff or greyish ochre, spotted with green particularly with
age or on handling.
Gills: orange-yellow bruising deep orange but becoming green with
time.
Flesh: pinkish to apricot-coloured but becoming green with age and
exuding a rich orange-red fluid which gradually becomes greyish
green.
Frequent in conifer woods and plantations.
L. glyciosmus (Fries) Fries
Coconut-scented milk-cap
Cap: width 20-50 mm. Stem: length 30-50 mm; width 5-8 mm.
Cap: usually with a central ‘bump’, greyish lilac, dull and minutely
scaly or velvety.
Stem: white to pale yellowish.
Gills: pale yellowish to flesh-coloured then flushed lilaceous.
Flesh: pale yellowish or flushed lilaceous, smelling strongly of desiccated
coconut and exuding a white unchanging milk-like liquid.
In woods and on heaths, particularly where birch is growing.
L. quietus (Fries) Fries
Oak milk-cap
Cap: width 30-80 mm. Stem: length 40-80 mm; width 10-15 mm.
Cap and stem: milky cocoa-coloured, zoned with reddish brown.
Gills: pale ochraceous then flushed red-brown.
Flesh: similar to gills, smelling strongly of rancid oil, and exuding a
white, thin milk-like liquid which becomes very, very faintly yellow
on exposure to the air.
Common wherever oak is growing.
L. rufus (Fries) Fries
Rufous milk-cap
Cap: width 50-90 mm. Stem: length 50-90 mm; width 10-15 mm.
Cap: dark red-brown with a distinct, usually sharp ‘bump’ in centre.
Stem: pale red-brown throughout or whitish at base.
Gills: pale reddish brown and exuding a white, unchanging milk-like
fluid.
In pine woods and less frequently with birches on acid heaths.
L. torminosus (Fries) S. F. Gray
Woolly milk-cap
Cap: width 40-150 mm. Stem: length 60-100 mm; width 15-30 mm.
Cap: pale strawberry-pink or pale salmon colour, distinctly zoned,
slimy when wet at centre and strongly shaggy fibrillose at margin.
Stem and gills: pale strawberry colour.
Flesh: tinged salmon-pink and exuding a white unchangeable milk-like
liquid.
Frequent where birches grow.
Amanita muscaria (Fries) Hooker
Fly agaric
Cap: width 100-175 mm. Stem: width 30-40 mm; length 150-275 mm.
Description:
Cap: bright scarlet to orange-red with scattered whitish or yellowish
fragments of veil particularly towards the centre and hanging down
from the margin, viscid when moist, striate at margin with age.
Stem: white, striate above the soft easily torn, although prominent,
ring which is white above and yellow below; stem-base swollen and
ornamented with patches of yellowish or white veil-fragments which
form concentric rings or ridges of tissue.
Gills: white, free, crowded, fairly thick, minutely toothed at their edge.
Flesh: soft, lacking distinctive smell, or at times slightly earthy and
white, yellowish below cap-centre.
Spore-print: white.
Spores: long, hyaline under the microscope, ellipsoid, smooth about
10 × 7 µm in size (10-13 × 7-8 µm).
Marginal cystidia: composed of chains of swollen, hyaline cells.
Facial cystidia: absent.
Habitat & Distribution: Found in birch-woods, less frequently collected
in the vicinity of conifers; wide-spread and fairly common, but it is
erratic in its appearance giving the impression of being absent from
a locality until one season it suddenly fruits in profusion.
General Information: An easily recognised fungus because of its striking
colour. It is also very familiar and well-known because it appears so
often on Christmas cards, and features commonly in illustrations in
children’s story-books. The fungus contains a poison which formerly
was used to kill flies—hence the common name of ‘Fly agaric’ and
the scientific name from the latin name for the house-fly. The red
skin of the cap, where the major amount of the poison resides, was
cut up with a little milk and sugar or honey; flies attracted to this
sweet concoction inadvertently ate the poison and later perished.
This fungus has a very well documented and long history and appears
in the legends of many countries. It is featured in Greek mythology,
Slavic and Scandinavian folk-lore and indeed appears in the pre-history
of Indian tribes of N.E. Asia. It has even been connected
with the formation of certain sects within the early Christian church.
Illustrations: F. frontispiece; Hvass 1; LH 117; NB 1131; WD 21.
Notes on the genus Amanita
The genus Amanita contains many important mycorrhizal fungi
including the ‘Blusher’, A. rubescens (Fries) S. F. Gray, the ‘Tawny
grisette’, A. fulva Secretan, and the ‘False death-cap’, A. citrina
S. F. Gray. The first grows on heaths and in woods with a variety of
trees; A. fulva frequently grows with birch and A. citrina with several
leafy trees although its var. alba (Gillet) E. J. Gilbert appears to be
confined to beech woods. However, there is some evidence that many
members of the genus in drier more southern countries than Britain,
are non-mycorrhizal. In fact the genus as a whole may be southern-temperate
in its distribution. In the British Isles the number of species
of Amanita recorded decreases as one goes north, or the frequency of
single species except for a few widespread forms falls off northwards.
In a few cases a more familiar southern species is replaced in similar
habitats by another species, e.g. A. phalloides (Fries) Secretan is replaced
by A. virosa Secretan the ‘Destroying angel’ in Scotland, and A.
citrina frequently in the north by A. porphyria (Fries) Secretan.
Species of Amanita are usually large conspicuous fungi and the genus
contains some of our best known agarics. One, A. muscaria (Fries)
Hooker has already been mentioned, but the genus also includes the
‘Death-cap’ A. phalloides and ‘Caesar’s mushroom’ A. caesarea (Fries)
Schweinitz, a fungus not found in this country but considered to be
superior in edibility to all other fungi; thus edible and deadly poisonous
species are found closely related and this simply emphasises how
important it is not to eat the agarics one finds in the woods and
fields except when accompanied by a ‘real’ expert. Deaths or near
fatalities in Europe and North America are recorded annually due to
the eating of fungi belonging to this genus.
The poisonous qualities of the fungi in this genus—only a very
small amount of poison is often sufficient to produce fatal results—has
led to a close connection between these fungi and black magic and
the supernatural. This connection is even more emphasised when it is
learnt that some have an intoxicating effect. Hence the long history
mentioned earlier.
Members of the genus Amanita are characterised by their anatomy
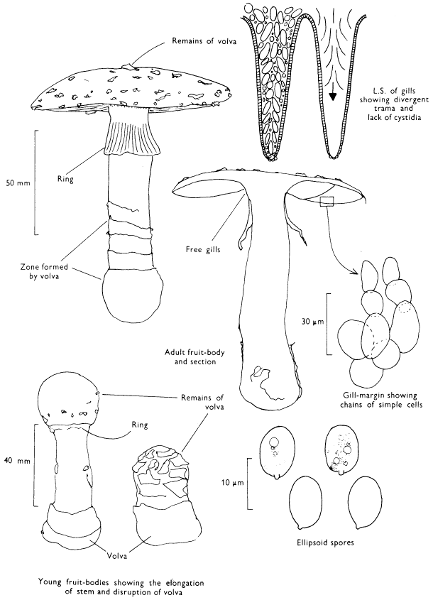
and certain macroscopic features; the former is illustrated under
A. muscaria, i.e. the divergent gill-trama. The main macroscopic
character of note is the presence of a volva at the base of the stem
and it is the details of this volva which helps to distinguish different
species. A. phalloides has a distinct, loose, membranous sheath, in A.
citrina the volva is reduced to a narrow rim around the bulbous stem
and in A. rubescens and A. muscaria the volva is simply a series of concentric
zones of woolly scales. All the four species noted above possess
a ring, but A. fulva the ‘Tawny grisette’ and A. vaginata (Fries)
Vittadini the ‘Grisette’ only possess a volva; this has lead to the use
of the generic name Amanitopsis in many books, now no longer considered
necessary.
The veil in Amanita is probably the most highly developed amongst
our common agarics and from Appendix iv it can be seen how the
scaly cap and stem originate and how the volva differs from the ring.
The volva and cap-scales constitute what has been called the universal
veil and the ring which stretches from the cap margin to the stem has
been termed the partial veil.
The spores of species of Amanita are large and their shape and
chemical reactions help to distinguish the different species within the
genus. One of the most interesting features, however, is that the spore-mass,
although usually described as white, in many species is not white
but flushed greenish grey, etc. The slight subtleties in colour of the
spore-print assist in classification.
The following notes may be instructive in conjunction with the
information above (for common names see above).
(i) Possessing a ring on the stem:—
A. citrina S. F. Gray
Cap: width 55-80 mm. Stem: width 18-22 mm; length 70-80 mm.
A lemon-yellow or whitish capped agaric with bulbous stem-base,
white patches of volva on cap and white stem with flesh strongly
smelling of new potatoes.
Spores: almost globose and measuring 9-10 × 7-8 µm.
A. excelsa (Fries) Kummer
Cap: width 75-140 mm. Stem: width 20-28 mm; length 85-120 mm.
A greyish or brownish capped agaric with clavate stem-base, grey
patches of volva on the cap and white concentrically scaly stem
with flesh unchanged on exposure to the air.
Spores: broadly ellipsoid and measuring 9-10 × 8-9 µm.
A. rubescens (Fries) S. F. Gray
Cap: width 70-120 mm. Stem: width 12-25 mm; length 65-100 mm.
A reddish fawn or pinkish buff capped agaric with swollen stem-base,
pinkish or flesh-coloured patches of volva on cap and reddish concentrically
scaly stem with flesh becoming reddish when exposed to
the air.
Spores: ellipsoid and measuring 9-10 × 5-6 µm.
A. pantherina (Fries) Secretan
‘Panther’
Cap: width 48-95 mm. Stem: width 12-20 mm; length 65-100 mm.
An olive-brown or smoky brown capped agaric with only slightly
swollen stem-base, white patches of volva on the cap and white
concentrically scaly stem with unchanging flesh.
Spores: ellipsoid and measuring 8-12 × 7 µm.
A. phalloides (Fries) Secretan
Cap: width 70-85 mm. Stem: width 12-20 mm; length 85-120 mm.
A greenish or yellow-olive capped agaric with stem sheathed in membranous
volva, white patches of volva on cap and smooth, white
stem with white flesh.
Spores: broadly ellipsoid and measuring 10-12 × 7 µm.
(ii) Lacking ring on stem:—
A. fulva Secretan
Cap: width 40-60 mm. Stem: width 10-15 mm; length 100-150 mm.
A thin, tawny-brown agaric with stem sheathed in membranous volva
and pale tawny, slightly scaly stem.
Spores: globose and 10-12 µm in diameter.
A. vaginata (Fries) Vittadini
Differs from A. fulva in the cap being metallic grey or silvery in colour.
Armillaria mellea (Fries) Kummer
Honey-fungus
Cap: width 50-150 mm. Stem: width 10-12 mm; length 75-150 mm.
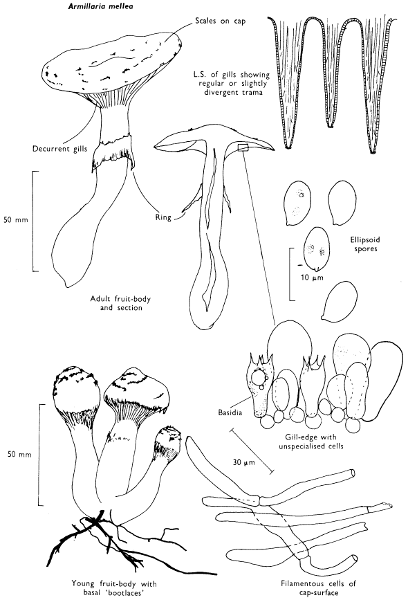
Description: Plate 10.
Cap: at first convex then more or less flattened or slightly depressed,
very variable in colour, yellowish, olive, buff, sand-coloured or some
shade of brown, at first covered in small, brownish or ochraceous
scales which give the young cap a velvety aspect, but gradually the
scales disappear with age except at the cap-centre; margin striate
and usually paler than centre of the cap.
Stem: equal or swollen at base, often several grouped together, white
at apex above a whitish, rather thick, ring which is flushed with
olive-yellow or red-brown at its margin; stem-base fibrillose,
whitish but finally red-brown at maturity.
Gills: adnate or slightly decurrent, whitish then flushed flesh colour
and developing brownish spots with age or in cold, wet weather.
Flesh: with rather strong and unpleasant smell, white or flushed
pinkish in the cap, brown and stringy in the stem.
Spore-print: very pale cream colour.
Spores: medium-sized, hyaline, ellipsoid, less than 10 µm in length
(8-9 × 5-6 µm).
Marginal cystidia: variable, hyaline, cylindric and not well-differentiated.
Facial cystidia: absent.
Habitat & Distribution: This fungus grows in troops or is found joined
at the base to form clusters. It is always attached to old trees, trunks,
stumps and buried wood, either directly or by its vegetative stage
which darkens and aggregates to form strands resembling boot-laces
which are called rhizomorphs.
General Information: This rather variable, and therefore often perplexing,
fungus causes a destructive rot of trees and can travel long distances
through the soil with the use of its rhizomorphs. It commonly
grows on several species of broad-leaved trees, but can also colonise
conifer trees. It also attacks garden shrubs, such as privet-hedges,
and is particularly destructive to Rhododendrons causing a wilt of the
whole shrub and subsequent death; it has also been recorded as
attacking potatoes. The actively growing mycelium which can often
be found growing under the bark of infected trees, exhibits a luminosity
if freshly exposed and placed in a darkened room. The rhizomorphs
of A. mellea are highly specialised structures composed of
mycelial threads some of which have become rather more differentiated
than is normally found in the vegetative stage of other agarics.
Illustrations: F 27a; Hvass 26; LH 93; NB 1411; WD 43.
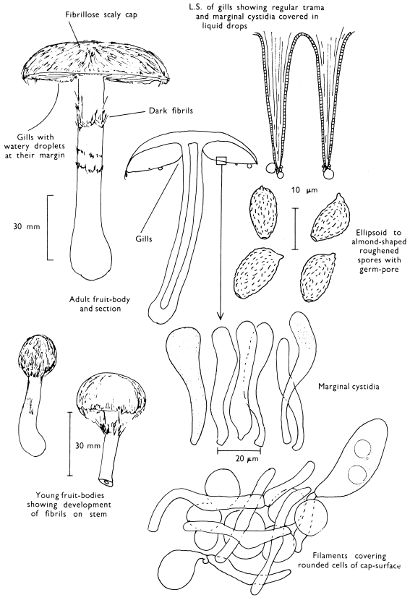
Pholiota squarrosa (Fries) Kummer
Shaggy Pholiota
Cap: width 50-120 mm. Stem: width 17-25 mm; length 95-125 mm.
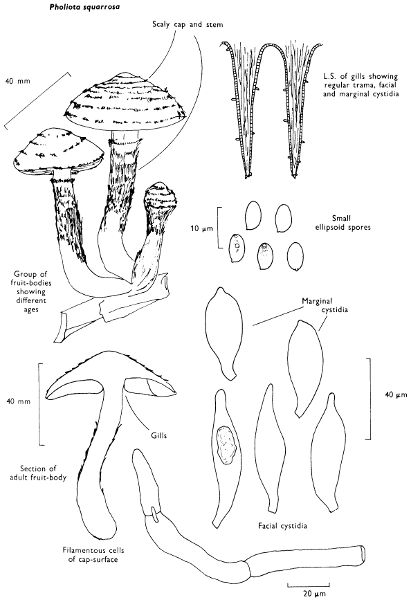
Description: Plate 11.
Cap: convex, but expanding and becoming flattened with a slight
central umbo, ochre-yellow to yellowish rust-colour and covered
with dark brown recurved scales which are particularly dense at
the centre.
Stem: variable in length and thickness depending on how it is attached
to the substrate, whether in a deep crack or wound, or in a depression,
and how many specimens are in the cluster; its colour is similar to
that of the cap, exhibits a small, dark brown fibrillose, torn ring or
ring-zone and is ornamented with recurved red-brown scales below
that ring.
Gills: broadly adnate with a decurrent tooth and crowded, yellowish
at first then rust-coloured.
Flesh: with strong, pleasant but pungent smell, yellowish brown, soft
in the cap, fibrous in the stem.
Spore-print: rich rust-brown.
Spores: medium-sized, pale brown under the microscope, smooth,
ellipsoid, and 6-8 × 4 µm in size.
Marginal cystidia: spindle-shaped, hyaline, numerous.
Facial cystidia: flask-shaped with a small apical appendage and becoming
rich yellow when immersed in solutions containing ammonia.
Habitat & Distribution: Common in clusters in woods, gardens or
parks, on wood or at the base of the trunks of broad-leaved trees in
summer and autumn.
General Information: Although rather a common easily recognisable
and aesthetically pleasing fungus growing in its characteristic clusters
at the base of trees, it is a weak parasite entering the living tissue
after invading decayed areas of the tree. This is the reason why
when branches are broken off trees by wind, snow or storms, they
should be carefully trimmed to remove ragged edges and the
wound treated with a protective tar to stop the entry of rain, cold
and fungus spores. Other more destructive fungi may enter a tree
through such wounds; P. squarrosa frequently attacks mountain ash
or rowan.
It is recognised by the dry scaly cap and stem which helps to
distinguish it from the sticky capped P. aurivella (Fries) Kummer
with similar habitat preferences but wider spores (6-9 × 4-5 µm).
P. adiposa (Fries) Kummer is found on beech trees and it, too, has a
viscid cap, but the spores are 5-6 × 3-4 µm in dimensions.
Illustrations: Hvass 134; LH 149; WD 542.
Hypholoma fasciculare (Fries) Kummer
Sulphur-tuft
Cap: width 20-50 mm. Stem: width 6-13 mm; length 40-100 mm.
Description:
Cap: sulphur-yellow, flushed with sand-colour or red-brown at centre
then ochraceous yellow throughout, convex at first with margin
incurved and clothed with fibrillose remnants of a yellow-olive veil,
but then becoming flattened and losing evidence of that veil.
Stem: equal or flexuous, usually with several joined at base, similarly
coloured to the cap, fibrillose streaky or with some fibrils from the
veil stretching from the cap to the stem in young specimens.
Gills: sinuate and crowded, at first sulphur-yellow then olive-green,
but finally with a flush of purple-brown.
Flesh: with rather strong and unpleasant smell, yellow throughout.
Spore-print: purple-brown.
Spores: medium-sized, ellipsoid or ovoid, smooth, purple-brown and
less than 10 µm in length (6-8 × 4 µm).
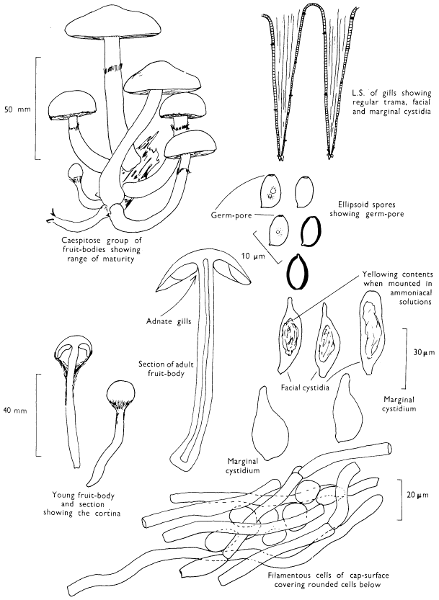
Marginal cystidia: flasked-shaped, short, cylindric and hyaline.
Facial cystidia: more swollen than marginal cystidia and with silvery
contents which yellow in solutions containing ammonia.
Habitat & Distribution: The sulphur-tuft grows in dense clusters on
and around old stumps of broad-leaved trees, and can be found
throughout the year; it also grows on conifers, but less frequently.
General Information: It may be recognised by the greenish tint of the
immature gills and of the young cap. H. capnoides (Fries) Kummer
grows on the wood of coniferous trees and has a much more ochraceous
brown cap and stem than the sulphur-tuft and slightly larger
spores—7-8 × 4-5 µm. H. sublateritium (Fries) Quélet grows on
hardwoods but is bigger than H. fasciculare and has a brick-coloured
cap and very sturdy stem (spores 6-7 × 3-4 µm).
Illustrations: F 37b; Hvass 176; LH 147; NB 1415; WD 762.
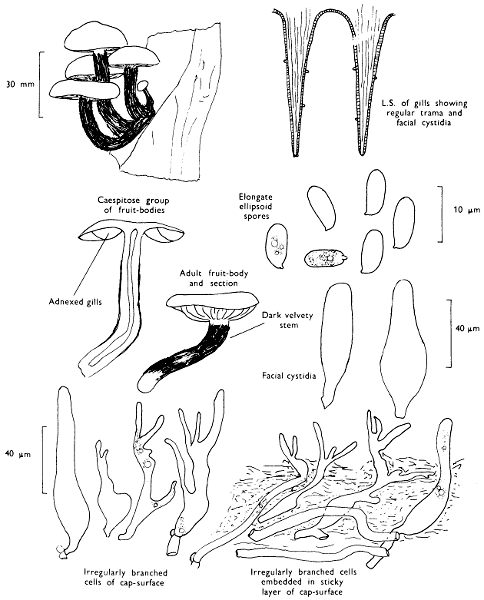
Flammulina velutipes (Fries) Karsten
Velvet-shank
Cap: width 20-80 mm. Stem: width 5-10 mm; length 35-60 mm.
Description:
Cap: bright sand-colour or slightly red-brown at centre, convex at
first then flattened with age, smooth, slimy because of the presence
of a sticky elastic skin, rather rubbery to the touch.
Stem: cylindrical or slightly swollen towards the base, dark brown and
densely hairy or velvety, tough and rubbery to handle.
Gills: adnexed, very unequal and somewhat distant, pale yellow, gradually
becoming buff as the spores mature.
Flesh: with rather pleasant smell, yellowish, watery and soft.
Spore-print: white.
Spores: medium-sized, hyaline, ellipsoid and about 8 × 3-4 µm in
Size (7-9 × 3-4 µm).
Marginal cystidia: hyaline, elongate, broadly flask-shaped.
Facial cystidia: similar to marginal cystidia.
Habitat & Distribution: Found in clusters on old stumps, fallen trunks
and on the wounded parts of standing trees.
General Information: This fungus can be recognised by the clustered
habit, the viscid, bright tawny cap and the dark velvety stem. This
is one of the few agarics which occurs regularly late in the season,
even appearing in the winter, although it can be seen growing in
its familiar groups at almost any time of the year. This fungus holds
a rather isolated position in classification and was once placed in the
genus Collybia. It may be found in several books under this last
genus.
Illustrations: F 18b; Hvass 80; LH 109; NB 1413; WD 214.
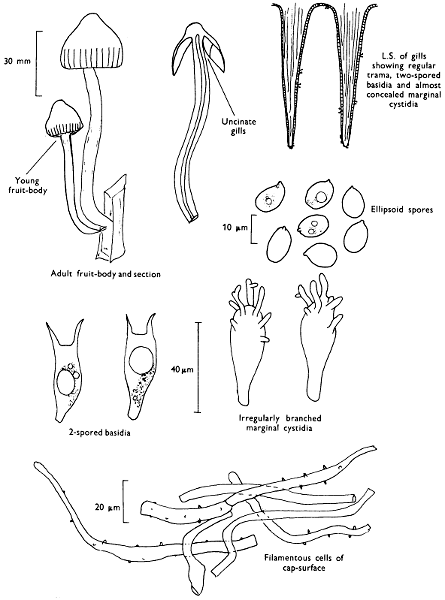
Mycena galericulata (Fries) S. F. Gray
Bonnet mycena
Cap: width 25-50 mm. Stem: width 3-6 mm; length 50-125 mm.
Description:
Cap: conical or bell-shaped then expanding but retaining a central
umbo, never completely flattened, smooth, greyish, pale sepia or
dirty white and striate with darker lines from the margin to the
centre.
Stem: similarly coloured to the cap, smooth, shiny, tough and usually
noticeably downy at base.
Gills: at first white flushed distinctly pale pink with age, uncinate,
rather distant and sometimes with interconnecting veins.
Flesh: white with little or no distinctive smell.
Spore-print: white.
Spores: medium-sized, hyaline, broadly ellipsoid, smooth, about 10 ×
7 µm in size (9-12 × 6-8 µm) and staining bluish grey when mounted
in solutions containing iodine.
Marginal cystidia: club-shaped but the apex ornamented with blunt
hairs of varying lengths.
Facial cystidia: absent.
Habitat & Distribution: Commonly found, in all but the coldest months,
in woods, parks or gardens, often in dense clusters on stumps and
fallen trunks of broad-leaved trees.
General Information: This is one of our commonest members, and one
of the largest in the genus Mycena; many species in this genus are
quite small yet are nevertheless very important components of the
woodland flora decomposing leaves, twigs, etc., and contributing in
this way to the recirculating of organic matter.
The name Mycena is derived from the same Greek word as that
which refers to the country around the ancient city of Mycenae in
the plain of Argos, and from whence Agamemnon came and gathered
his forces to invade Troy to reclaim Helen his wife. It has been
suggested that this similarity in name came about through the
necessity for an army stationed in Argos, early in the history of
Ancient Greece, to rely on the mushrooms found on the plains
about to save the soldiers from starvation.
Illustrations: F 17a; Hvass 119; LH 109; NB 1338; WD 263.
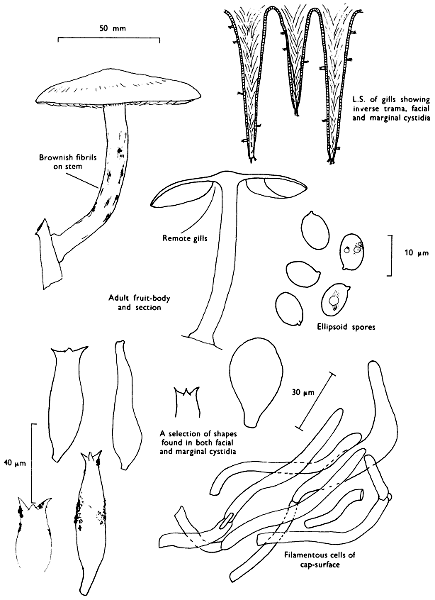
Pluteus cervinus (Fries) Kummer
Fawn pluteus
Cap: width 40-100 mm. Stem: width 10-15 mm; length 75-125 mm.
Description:
Cap: conical, rapidly expanding and then becoming plano-convex or
flattened with only a slight but persistent umbo, dark brown, umber
or vandyke brown, viscid when wet and often with radiating fibrils.
Stem: white, streaked to varying degrees with dark brown fibrils,
cylindrical or slightly swollen towards the base, where it is attached
to the substrate.
Gills: remote, very crowded, thin, at first white then distinctly salmon-pink.
Flesh: with pleasant smell, white and soft.
Spore-print: dull salmon-pink.
Spores: medium-sized, very faintly buff under the microscope,
broadly ellipsoid and 7-8 × 5-6 µm in size.
Marginal cystidia: flask-shaped, the majority with three or four hooks
at the distinctively thick-walled apex.
Facial cystidia: similar to marginal cystidia but sometimes intermixed
with those lacking hooks.
Habitat & Distribution: This fungus grows singly or in groups on old
stumps and fallen trunks throughout the year except for the most
wintry months; it is commonest in autumn.
General Information: This fungus may also grow on old sawdust heaps,
a habitat which is often very worth while examining in detail by the
interested amateur during wet seasons. In summer sawdust heaps
dry out but after a good soaking, which, of course, can be applied
artificially by frequent watering with a hose or watering-can, many
interesting fungi develop. On sawdust heaps containing conifer
debris a larger species with black or dark brown edge to the gills is
found—P. atromarginatus Kühner.
The peculiar pointed cystidia found on the gill-edge and on the
gill-face of P. cervinus were thought by some early mycologists to
stop mites and insect larvae from crawling up between the gills and
damaging the developing spores. There is no evidence that this
actually takes place in nature; the real purpose of these obscure
structures is unknown and has been little studied.
Illustrations: Hvass 127; LH 121; NB 1351; WD 502.
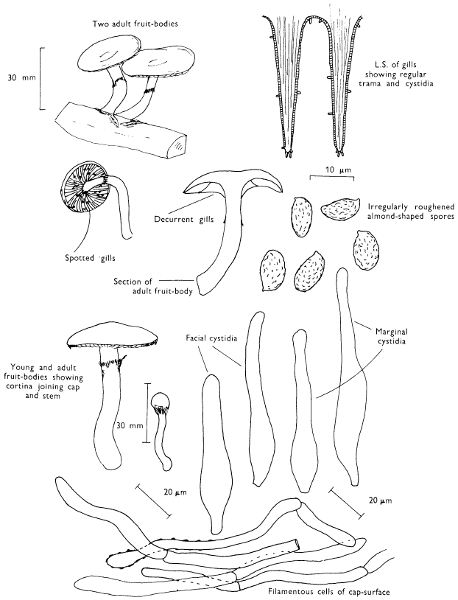
Gymnopilus penetrans (Fries) Murrill
Cap: width 20-50 mm. Stem: width 4-7 mm; length 20-50 mm.
Description:
Cap: convex then becoming flattened at maturity, dry, slightly scaly,
golden tawny, or rusty yellow and when young with the remnants
of a rapidly disappearing yellow cortina hanging from the margin.
Stem: yellow above and red-brown or orange-tawny below and
darkening on bruising; veil forming a delicate fibrillose zone in the
upper part of the stem which is soon lost on excessive handling.
Gills: adnate to slightly decurrent, thin and crowded, at first golden
yellow, but soon spotted rust colour.
Flesh: yellow and lacking distinctive smell.
Spore-print: rich orange-tawny.
Spores: medium-sized, ellipsoid, finely roughened and deep yellow
brown under the microscope, less than 10 µm in length (7-8 × 5-4
µm).
Marginal cystidia: hyaline, flask-shaped with long often slightly
irregular neck.
Facial cystidia: similar to the marginal cystidia, but often broader.
Habitat & Distribution: This fungus is found on sticks or twigs or
chips of coniferous wood, particularly in plantations.
General Information: Although it has only comparatively recently been
recognised in Britain it is very wide-spread. It has been confused
with, indeed described under, the name of the less-common fungus
Gymnopilus sapineus (Fries) Maire which also grows in conifer
woods; it is easily distinguished, however, by its spotted gills. Both
the fungi above can be found in books under the old name Flammula,
from the bright colour of the caps of many of its constituent members,
but Flammula has been used for a genus of flowering plants also
and this has precedence.
Illustrations: F 29a; Hvass 152 not very good; LH 175 not very good;
NB 1096.
Notes on the artificial family group ‘Pleurotaceae’—the Oyster
mushrooms
One of the common features of lignicolous fungi is the fact that they
lack a distinct stem or if one is present it is attached to one side of the
cap, i.e. lateral. However, in the past the correlation of the habitat
with lack of stem has induced mycologists to define a single family to
include all these forms. After studying the anatomy and microscopic
characters this grouping has been found to be entirely artificial and
simply reflects how the morphology is tied up intimately with the
ecology of a species.
In this one family members of the genera Panus, Panellus, Lentinus,
Lentinellus, Crepidotus, Pleurotellus, and Pleurotus have all been grouped
together, but some of the genera are more related to the polypores
referred to later (p. 135); many of those with brown spores are better
placed with Cortinarius and some of those with white or cream-coloured
spores are better placed close to Mycena and Tricholoma. This leaves
as a residue the genus Pleurotus, a genus which although rather heterogeneous
contains one familiar member, i.e. the common Oyster mushroom,
Pleurotus ostreatus.
Pleurotus ostreatus (Fries) Kummer
Oyster mushroom
Grows up to 150 mm across.
Cap: flattened, shell-shaped, smooth or slightly cracked, deep bluish
grey, gradually becoming brownish with age and finally dark buff.
Stem: absent or very short, passing gradually into one side of the cap.
Gills: white flushing dirty yellow with age, rather distant and deeply
decurrent.
Flesh: white, soft and with very pleasant smell.
Spore-print: pale lilac.
Spores: long, hyaline, oblong under the microscope and 10-11 × 4 µm
in size.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common, clustered in tiers on stumps, trunks,
posts, etc.
General Information: This fungus is not infrequent on old telephone-poles
and forms white sheets of mycelium immediately under the
bark of fallen trees. Although frequent in autumn it may be found
throughout the year and is easily recognised by its size and bracket-like,
shell-shaped caps. It surprisingly has a pale lilac spore-print
and not as might be expected a white spore-print. In the var.
columbinus Quélet the young caps are a beautiful peacock-blue; this
variety frequently grows on poplars.
Illustrations: F 1252; Hvass 109; LH 107; NB 1252; WD 311.
Plate 17. Wood-inhabiting, fleshy but leathery fungi: Spores whitish or brownish
and borne on gills—‘Pleurotaceae’
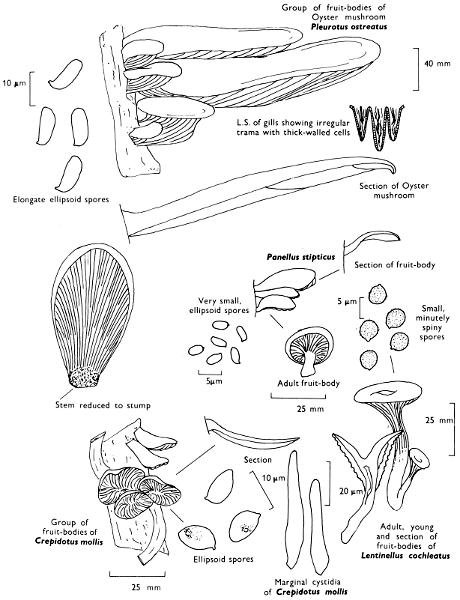
Larger illustration
Panus torulosus (Fries) Fries
is a tough, funnel-shaped, yellowish
cinnamon fungus with oblong-ellipsoid, small, hyaline spores
measuring 5-6 × 3 µm and changing yellowish not bluish grey in
iodine solutions.
Panellus stipticus (Fries) Karsten
forms tiers of pale cinnamon-brown,
more or less kidney-shaped, scurfy caps on old wood and has
egg-shaped, hyaline, small spores measuring 4 × 2-3 µm which
become bluish grey in iodine solutions.
Lentinellus cochleatus (Fries) Karsten
forms irregular lobed and
twisted, flattened or funnel-shaped dirty brownish caps with a
fragrant smell, toothed gill-edges and almost spherical, small, hyaline
spores measuring 5 × 4 µm which become bluish grey in iodine
solutions.
Lentinellus apparently has very close affinities to Auriscalpium, ‘the
Ear pick fungus’, (p. 158) both in the structure of the spores and the
anatomy of the fruit-body.
Lentinus lepideus (Fries) Fries
forms very tough fruit-bodies with
convex or flattened, pale yellowish caps and stems ornamented with
dark tawny or brown scales. The stem is often eccentric and buried
in cracks or soft rotten wood on which it grows; the spores are non-amyloid.
It grows on pine stumps but also on decaying or unprotected
railway sleepers and wooden paving blocks, joists, etc., made of
conifer wood. When the fungus fruits in a darkened environment,
such as a cellar, the mushroom-like fruit-bodies are not produced
but are replaced by slender branched structures similar to the ‘Stag’s
horn’ or ‘Candle-snuff fungus’ (p. 206), or to certain of the Fairy
Club fungi (p. 172). Similar growths have been recorded for
Polyporus squamosus which grows on hard wood timber and is
described in detail later (p. 140).
Crepidotus mollis (Fries) Kummer
Soft slipper toadstool
Cap: up to 45 mm across and in tiers, sessile, shell-shaped or kidney-shaped,
smooth, rubbery and brownish ochre in colour.
Gills: pale buff then cinnamon-brown and finally flushed snuff-brown,
thin and crowded.
Flesh: watery, gelatinous beneath the skin of the cap and whitish buff.
Spore-print: warm brown.
Spores: ellipsoid, smooth, medium-sized, pale buff under the microscope
and 8-9 × 5-5·5 µm in size.
Easily recognised by the soft elastic cap which can be stretched without
breaking, the brown gills and pale buff spores. (See Plate 49, p. 153.)
Illustrations: LH 177; NB 1453; WD 691.
The artificiality of classifying all those agarics with both a spoon-shaped
or bracket-shaped fruit-body, and a reduced (or lacking) stem
is further exemplified by the presence of similar genera in other
groups of fungi. For instance Claudopus is typified by pink, angular
spores (Plate 28) and Clitopilus is characterised by longitudinally
ridged spores, i.e. they are not angular in all optical sections but only
when seen end on (see p. 101). An example of the former is C.
parasiticus (Quélet) Ricken which grows on dead remains of woody
fungi, and of the latter C. passackerianus (Pilát) Singer which may
invade mushroom beds. Both species are quite small though the last
fungus is similarly coloured to the more familiar Clitopilus prunulus
(Fries) Kummer, ‘The Miller’, so common in woods and fields.
Thus in the British Isles agarics with eccentric stems may be found,
in the white, brown and pink-spored groups—and in the tropics and
subtropics the picture is completed by the existence of the genus
Melanotus in the black-spored agarics. M. bambusinus Pat. grows on
bamboos and M. musae (Berk. & Curt.) Singer grows on dead leaves
and debris of bananas; the latter is also a probable agent in the decay
of fibres in the tropics.
Melanoleuca melaleuca (Fries) Murrill
Cap: width 40-110 mm. Stem: width 50-80 mm; length 50-90 mm.
Description:
Cap: dark brown, umber or vandyke when moist, hygrophanous and
becoming very much paler on drying almost tan, convex then
flattened sometimes umbonate, smooth or wrinkled.
Stem: white or whitish covered in brownish fibrils which increase in
number with age or after handling; solid, rather elastic and slightly
swollen towards the base.
Gills: white, broad, crowded and as if cut out from behind before
joining the stem.
Flesh: with pleasant smell, soft, white, becoming brownish with age,
particularly in the stem.
Spore-print: very pale ivory-colour.
Spores: medium-sized, ellipsoid, hyaline under the microscope and
roughened by distinct dots which become blue-black when mounted
in solutions containing iodine, 8 × 4-5 µm.
Marginal cystidia: spear- or sword-shaped, roughened with crystals
at the top and appearing as if barbed like fish-spines.
Facial cystidia: numerous and similar to marginal cystidia.
Habitat & Distribution: Common in autumn in woods; also found in
pastures.
General Information: A very common fungus which is rather confusing
to the beginner because of its variation in colour, brought about by
the change in colour with change in content of water. However, this
fungus can be easily recognised by the unusually ornamented cystidia
found on the gill-faces and gill-margins. This character and the
fact that the spores possess amyloid ornamentation define in part
the genus Melanoleuca. In many books this common fungus is found
under the genus Tricholoma; however, members of this latter genus
have neither amyloid ornamented spores nor barbed cystidia.
Illustrations: LH 103; WD 131.
Clitocybe infundibuliformis (Weinm.) Quélet
Common funnel-cap
Cap: width 20-60 mm. Stem: width 8-13 mm; length 35-75 mm.
Description:
Cap: yellowish ochre flushed slightly pinkish buff or cinnamon
but later pale tan on ageing or drying, funnel shaped.
Stem: colour like cap or slightly darker, flexible but firm and solid.
Gills: white or faintly flushed buff, decurrent and crowded.
Flesh: with pleasant slightly floral smell, white, soft and fairly thin.
Spore-print: white.
Spores: medium-sized, hyaline, tear-drop shaped, smooth, 6-7 × 3-4
µm and not blueing when mounted in solutions containing iodine.
Marginal cystidia: little different from young basidia in dimension and
shape, although some may have a short apical prolongation.
Facial cystidia: absent.
Habitat & Distribution: Woods, copses, heaths and hill-pastures from
summer to autumn.
General Information: An easily recognisable fungus because of its
graceful stature, thin, funnel-shaped pinkish buff cap and tear-drop-shaped
spores. Several Clitocybe species grow in woodlands, many of
them appearing later in the season when colourful agarics are rarer.
The genus Clitocybe is characterised by the fleshy cap with incurved
margin when young, fibrous, fleshy stem and decurrent gills.
C. clavipes (Fries) Kummer has a smoky brown, top-shaped cap,
fragile stem which also has a distinct swelling at its base, and strong
rather unpleasant smell. C. nebularis (Fries) Kummer is similar, but
is pale cloudy grey, has a less fragile stem and a fairly pleasant smell.
This species if often covered in a bloom which develops further as
the fruit-body deteriorates. The agaric Volvariella surrecta (Knapp)
Singer is a rare parasite of C. nebularis (see p. 247) and it has been
suggested that this bloom may in fact belong to this species. However,
I have on several occasions tried to encourage the bloom to
reproduce by keeping hoary looking fruit-bodies of C. nebularis in
a damp-chamber, but as yet I have never been successful.
Nevertheless, it is an exercise which would be of great interest
to continue and a source of great excitement if the small pink-spored
agaric were produced. C. fragrans (Fries) Kummer is a small,
sweetly aromatic-smelling species found in frondose woods, and
C. langei Hora, is a mealy-smelling species of conifer plantations.
Illustrations: F 16a; Hvass 55; LH 95; WD 162.
Hebeloma crustuliniforme (St Amans) Quélet
Fairy-cake mushroom
Cap: width 40-80 mm. Stem: width 8-12 mm; length 38-85 mm.
Description:
Cap: pale yellow buff or pale tan with a distinct reddish buff or
cinnamon-brown tint, darkening only slightly with age; smooth,
at first tacky to the fingers, but then dry and shiny at centre,
convex and hardly expanding.
Stem: cylindrical or slightly swollen towards the base, whitish and with a
flush of pinkish buff at apex, and covered all over in small, white scales.
Gills: sinuate, crowded, pale clay-colour or buff, but finally dull dark
yellow ochre except for the distinct white margins which are beaded
in wet weather with droplets of liquid.
Flesh: whitish with a very strong smell of radishes.
Spore-print: dark clay-colour.
Spores: long, slightly almond-shaped, pale brown under the microscope,
distinctly warted and about 11 × 6 µm in size (10-12 × 6-7
µm).
Marginal cystidia: cylindrical to skittle-shaped with slightly to distinctly
swollen apex.
Facial cystidia: absent.
Habitat & Distribution: Common in autumn on the ground by pathsides
and in woodland clearings.
General Information: Recognisable by the uniform cinnamon or pinkish
buff cap, white woolly scales on the stem and distinctive, strong
smell of radish. There is some evidence that this species may on
occasions be mycorrhizal; further field studies are required.
There are several closely related fungi which are difficult for the
amateur to differentiate from H. crustuliniforme; there is no doubt
that there are several species present in the British Isles which do
not appear in the Check List of British Agarics & Boleti; in fact,
it would appear that there are several yet to be described as new to
science. Although individual species are fairly difficult to delimit,
the genus Hebeloma itself is easily recognised, most members being
medium sized with brown sinuate gills, whitish, yellowish, or pinkish,
i.e. pale, caps and white-powdered stems. The word ‘crustulin’
which appears in the Latin name of H. crustuliniforme is itself from
the Latin and means small cake, referring to the cap-shape, which
remains fairly constant throughout the fungus’ growth. The common
name is derived from this also.
Inocybe geophylla (Fries) Kummer
Common white inocybe
Cap: width 10-25 mm. Stem: width 3-6 mm; length 30-50 mm.
Description:
Cap: conical with incurved margin then bell-shaped and retaining a
distinct umbo even when mature, silvery white then ivory and
finally pale tan particularly centrally and silky fibrillose throughout.
Stem: slender, cylindrical but for a small swelling at the base, silky
and shining with a few fibrils from a former cortina which may be
brownish due to spores adhering to it at maturity.
Gills: adnexed to free, crowded, pale ochraceous becoming clay-coloured.
Flesh: white with smell of newly dug potatoes, strong when fresh.
Spore-print: clay-colour.
Spores: medium sized, ellipsoid or slightly French-bean-shaped,
smooth, yellow-brown under the microscope and 9-11 × 4-5 µm
in size.
Marginal and facial cystidia: flask- to spindle-shaped with distinctly
thickened walls and frequently ornamented with crystals apically.
Habitat & Distribution: Common in troops in woodland clearings, by
pathsides or on the edges of ditches bordering woods.
General Information: This fungus is easily recognised by the very pale
uniform colour, the colour of the spore-print, silky umbonate cap
and small size. The cortina connects the cap-margin and the stem
and consists of a cobwebby structure which collapses at maturity.
A violet coloured variety, var. lilacina Gillet is frequently found,
in fact, even accompanying var. geophylla; it differs only in the lilac-colour
of the cap and stem. I. geophylla is a member of the very large
genus Inocybe, further members of which will be dealt with later
(see p. 238).
The genus is well defined with dull-yellow spore-print, well
differentiated sterile cells on the gill-edge (and often on the gill-face)
and the cobweb-like veil, or cortina, stretching from the cap-margin
to the stem and easily observed in young specimens. The
genus is split into three distinct groups: those with smooth spores,
those with nodulose spores and those with subglobose spores ornamented
with long projections. I. geophylla is included in the first
group. The group which includes the nodulose-spored members
has been elevated to the rank of genus by some authors, i.e. Astrosporina—a
name referring to the spore-shape eg., I. asterospora.
Illustrations: F 13a (too blue); LH 155; NB 1395; WD 654.
Laccaria laccata (Fries) Cooke
Deceiver
Cap: width 12-28 mm. Stem: width 4-8 mm; length 15-60 mm.
Description:
Cap: hygrophanous, reddish brown or brick-colour becoming ochraceous
on drying, but can be rapidly returned to the original colour
by placing on the top a drop of water which is rapidly absorbed;
fragile, convex at first then flattened or depressed about centre,
smooth or surface scaley, striate at margin when moist.
Stem: similarly coloured to the cap, fibrous, cylindrical, tough and
usually with white woolly base.
Gills: adnate with or without a decurrent tooth, thick, distant and
pinkish or pale reddish-brown, powdered with white when mature.
Flesh: red-brown, soft in the cap and fibrous in the stem.
Spore-print: pure white.
Spores: medium sized, hyaline under the microscope and spherical,
7-8 µm in diameter and beautifully spiny.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common in troops in woodland, copses, on
heaths; in fact it may be found in nearly all possible habitats.
General Information: This is a very common agaric which in the future
will probably be split into several distinct species; unfortunately it
is as variable as it is common, hence the common name ‘deceiver’;
it is often mistaken at first glance for many other species quite unrelated.
I have seen even the most experienced mycologist pick up
rather unfamiliar specimens of Laccaria laccata in mistake for a species
of Lactarius or a species of Collybia, etc. I would hate to say more
because I have been ‘deceived’ myself on more than one occasion.
L. laccata appears to be a composite species, but because of the
difficulty in defining some of the characters the splitting of the
species has not as yet been satisfactorily solved. The smell, however,
may well give a clue for some specimens smell very strongly of
radish whilst others are odourless.
L. proxima (Boudier) Patouillard
, differs in having ellipsoid spores; it
is larger in stature and is common in wet places.
L. amethystea (Mérat) Murrill
, differs in the deep violet or amethyst-colour
of the fruit-body and commonly grows in shaded woods.
L. bicolor (Maire) P. D. Orton
, which is less frequent, has lilaceous
gills and violaceous mycelium at the base of the stem.
Illustrations: Hvass 66; NB 1331; WD 202.
Mycena sanguinolenta (Fries) Kummer
Small bleeding mycena
Cap: width 10-17 mm. Stem: width 2-4 mm; length 50-80 mm.
Description:
Cap: bell-shaped or conical expanding only slightly with age and so
remaining umbonate, reddish-brown, striate to the margin from the
darker apex and blotched age with red-brown spots.
Stem: pale reddish brown, very slender, fragile, woolly at the base and
exuding a red-brown juice when broken.
Gills: adnate, fairly distant, whitish to flesh-colour with a dark red-brown
edge and not noticeably becoming blotched with red-brown.
Flesh: with no distinctive smell, reddish-brown and very thin.
Spore-print: white.
Spores: medium sized, hyaline, ellipsoid to pip-shaped, smooth about
10 µm long (9-10 × 4-5 µm) and becoming bluish grey when
mounted in solutions containing iodine.
Marginal cystidia: awl-shaped, pointed at the apex, swollen below
and filled with dark red-brown contents.
Facial cystidia: absent.
Habitat & Distribution: Solitary or in small groups on poorly kept
lawns, in woods and copses; it is particularly frequent in the beds of
needles found in pine woods.
General Information: This fungus is easily recognised by the slender
habit, reddish juice exuded when broken and habitat preferences.
Mycena haematopus (Fries) Kummer is larger and grows in tufts
on wood, but also has a red-brown juice which, however, spots the
gills. Another very common species of Mycena is M. galopus (Fries)
Kummer which has a greyish or brownish cap and exudes a milk-like
juice. The related M. leucogala (Cooke) Saccardo is almost black
(see p. 216). These agarics exuding juice when broken have a flesh
composed of filaments, a very different flesh-structure to species of
Lactarius (see p. 50) and although their spores are amyloid they
do not turn blue-black in iodine because of the presence of amyloid
crests and warts. There are few additional species of agaric which
exude a milk-like liquid, but the majority of these are tropical or
subtropical. The second names or epithets for the four species
mentioned above all refer to the ‘latex’—sanguinolenta—bleeding,
haematopus blood-foot; galopus, milk-foot and leucogala, white milk.
For notes on Mycena one is referred to p. 68 describing M. galericulata
(Fries) S. F. Gray.
Illustrations: WD 284.
Collybia maculata (Fries) Kummer
Spotted tough-shank
Cap: width 80-130 mm. Stem: width 5-20 mm; length 50-158 mm.
Description:
Cap: white but soon becoming spotted with reddish-brown, finally
cream-colour with red-brown blotches, convex then becoming
flattened, fleshy, firm and tough.
Stem: white becoming streaked red-brown, thickest in the middle,
longitudinally furrowed or striate and often narrowed downwards
into a long irregular root embedded in the deep litter.
Gills: very crowded, cream-coloured, becoming spotted red-brown
with age.
Flesh: with pleasant smell, white and fibrous in the stem.
Spore-print: pinkish cream-colour.
Spores: small, almost spherical, hyaline under the microscope, about
5 µm in diameter (4-5 × 5 µm) and not blueing when placed in solutions
containing iodine.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common in troops in woods, particularly
beech but also found in pine woods and on heaths.
General Information: Easily recognised by the crowded, narrow, cream
coloured gills and the cap being entirely white when young, but which
rapidly becomes spotted red-brown as it develops. ‘Maculatus’
means spotted and refers to the red-brown blotches which develop
irregularly on the cap, stem and gills as the fruit-body matures.
The genus Collybia is characterised by the fruit-body being tough,
the cap-margin incurved at first and the spore-print white or whitish.
The common fungus C. maculata has always been assumed to have
a white spore-print but if a cap is placed on a piece of white paper
gills-down and left for twelve hours there is a surprise in store for
the careful observer.
Illustrations: F 15a; Hvass 77; LH 101; NB 1034; WD 212.
Plate 24. Fleshy fungi with tough stem: Spores white to cream and borne on gills
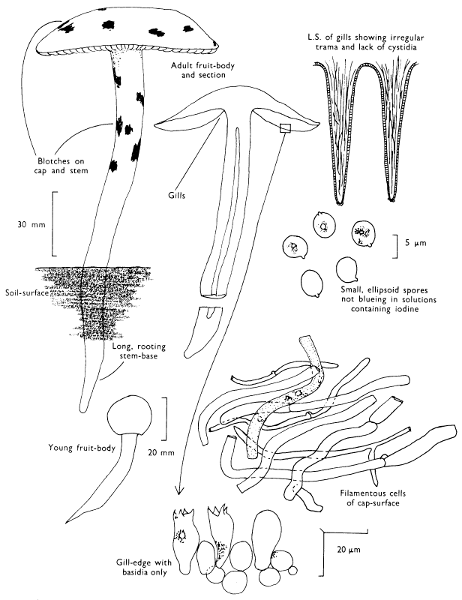
Larger illustration
The specialised substrates of certain species of Marasmius and
related genera
A whole series of very small fungi are found in woodland communities
which appear to be closely related one to another because their caps
are usually tough, although membranous, dry rapidly yet do not decay,
and, moreover, revive on remoistening. Their gills are also rather tough
and their spores always white in mass. They are placed in the genus
Marasmius. Collybia or Marasmius peronatus (Fries) Fries the ‘wood
woolly foot’ is one of our larger more familiar agarics related to this
group, but whereas it grows on all kinds of leafy detritus, even wood,
these small fungi appear to be very specific to the substrate on which
they grow.
M. androsaceus (Fries) Fries
grows both on heather and on pine-needles
(see p. 231).
Cap: whitish or pinkish buff.
Stem: black and hair-like.
Spores: pip-shaped and 7-9 × 3-4 µm.
M. buxi Fries
grows on box leaves.
M. epiphylloides (Rea) Saccardo & Trotter
grows on ivy leaves.
M. graminum (Libert) Berkeley
grows on grass stems.
Cap: red-brown.
Stem: dark brown.
Spores: pip-shaped, 8-12 × 4-6 µm.
M. hudsonii (Fries) Fries
grows on holly leaves.
M. perforans (Fries) Fries
grows on pine needles (now placed in the
genus Micromphale).
M. undatus (Berkeley) Fries
grows on bracken stems.
Cap: reddish brown or greyish and wrinkled.
Spores: egg-shaped, 8-9 × 6-7 µm.
Except for their rather special requirements as to substrate preference,
these species have in common small size, rather tough horny stems and
cap composed of erect ornamented cells.
Several agarics which grow on cones have also been placed in
Marasmius. They are frequent in spring and early summer the fruit-bodies
being attached by a very long rooting stem and cord of fluffy
hyphae to buried cones in conifers. The biology of these fungi is
still unknown, but the cones to which they are attached are always
closed yet buried often several inches beneath the surface of the soil.
It is yet to be found whether the spores of the agaric infect the cones
after they drop or whether the cones fall because they have become
infected. How do the cones become so deeply buried? Are squirrels
or rodents involved? All the species which grow on cones have brown
or tawny caps and yellowish brown stems.
Plate 25. Fleshy fungi with wiry to tough stem: Spores white and borne on gills,
fruit-body frequently reviving when moistened
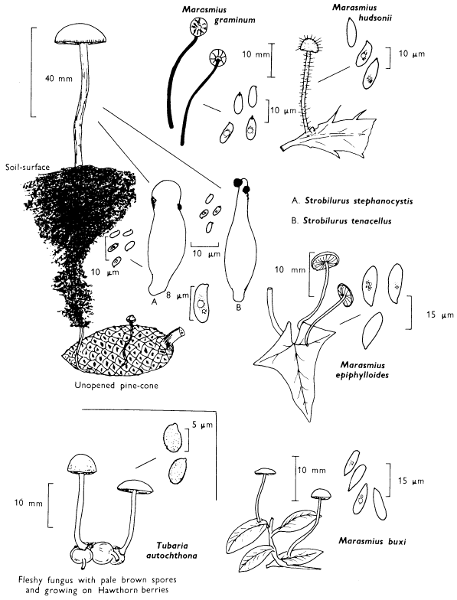
Larger illustration
Strobilurus stephanocystis (Hora) Singer
has cystidia with rounded
heads and grows on pine-cones.
S. tenacellus (Fries) Singer
has pointed cystidia and grows on pine-cones.
S. esculentus (Fries) Singer
has lance-shaped cystidia and grows on
spruce cones.
Baeospora myosura (Fries) Singer
is tough and pale-coloured and is
similar in general characters to species of Strobilurus, but has amyloid
spores and fruits on pine-cones in the autumn.
When discussing the specialised plant-substrates, such as cones, one
must mention the small brown-spored, pale buff coloured agaric
Tubaria dispersa (Persoon) Singer, or Tubaria autochthona (Berkeley &
Broome) Saccardo, which grows on the ground under hawthorns, often
in troops in summer and autumn, attached to old hardened hawthorn
berries.
Hygrocybe pratensis (Fries) Donk
Butter mushroom
Cap: width 20-80 mm. Stem: width 5-12 mm; length 30-70 mm.
Description:
Cap: convex then expanding to become plano-convex with a broad
low umbo, tan, pale russet or even yellowish buff throughout or
slightly darker at the centre.
Stem: gradually thickened upwards, similarly coloured to the cap or
paler if the cap is dark russet.
Gills: pale buff, deeply decurrent and often connected up at their
bases by veins.
Flesh: buff or pale tan, thick and soft in the cap, slightly fibrous in the
stem.
Spore-print: white.
Spores: medium-sized, ellipsoid to egg-shaped, hyaline under the
microscope, 7-8 × 5 µm in size and not becoming bluish grey in
solutions containing iodine.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common in pastures or on heaths from early
summer to late autumn.
General Information: A fungus easily recognised by the uniform buff-colour
of the stem, cap and gills. As one might expect from the
common name it is edible; it is held in high regard by many mushroom-pickers.
Although ‘pratensis’ specifically means fields, reflecting the habitat
of the fungus, this and related species can also be found on heaths and
pastures often intermixed and forming a most interesting flora. The
following are perhaps the most commonly seen:
H. lacma (Fries) Orton & Watling and H. cinerea (Fries) Orton &
Watling are similar in stature, but metallic grey in colour except for
the persistently yellow stem-base in H. lacma.
H. subradiata (Secretan) Orton & Watling is flesh-coloured or brownish
and H. virginea (Fries) Orton & Watling is white.
H. nivea (Fries) Orton & Watling and H. russocoriacea (Berkeley &
Miller) Orton & Watling are much smaller, the former white and
odourless and the latter off-white with a very strong smell of incense.
Illustrations: F 12b; Hvass 95; LH 77; NB 332; WD 333.
Hygrocybe psittacina (Fries) Wunsche
Parrot hygrophorus
Cap: width 12-25 mm. Stem: width 3-8 mm; length 30-60 mm.
Description:
Cap: very slimy with colourless sticky fluid, deep bluish green when
fresh, but becoming more and more ochraceous-orange with age or
completely fading out to a yellow ochre, bell-shaped at first then
expanded except for central umbo.
Stem: like the cap very slimy, apple-green or bluish green throughout
but becoming ochraceous like the cap except at the apex which is
persistently green.
Gills: adnate yellow or apricot-coloured, greenish towards their base,
broad, distant and rather tough.
Flesh: whitish, tinged green in the cap and yellow or apricot-colour
in the stem.
Spore-print: white.
Spores: medium-sized, hyaline, ellipsoid, not blue-grey in solutions
containing iodine and 8-9 × 4-5 µm in size.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common in grassland and hill-pastures, but it
also occurs in copses and woodlands.
General Information: This fungus is easily recognised by the distinctive
colours, but it is rather deceptive for the cap and the stem soon
become faded; however, the green colouration persists at the apex
of the stem and it is by this that in the faded state the fungus can
still be identified. H. laeta (Fries) Kummer fades to similar colours
but the cap is flesh-colour at first or sordid brown and the gills are
flesh-coloured or greyish; it prefers upland pastures and heathland:
its spores are smaller, being 5-7 × 4 µm.
Illustrations: F 12a; Hvass 92; LH 79; NB 336; WD 345.
General notes on Hygrophori
Hygrophori are some of our most colourful groups of agarics,
many are brightly coloured with caps in reds, greens, yellows,
oranges, etc., the colour often accentuated by the usually slimy aspect.
Traditionally the genus Hygrophorus has been split into three groups
as follows:—
Limacium with slimy cap, adnate to decurrent gills and slimy or tacky
stem which may also often be ornamented with dots, especially
towards the top.
Camarophyllus with dry cap, smooth and fibrous stem and decurrent
gills.
Hygrocybe with thin, fragile, sticky or moist cap, smooth fibrillose stem
and gills varying from free to decurrent.
The last two sections have been joined together into the single
genus Hygrocybe and all the members seem to be saprophytic or intimately
associated with grassland communities. The first section
Limacium now makes up the genus Hygrophorus and its members
are thought to be mycorrhizal with trees, e.g. H. hypothejus (Fries)
Fries with pine, the ‘Herald of the winter’ because it occurs at the end
of the fungus season and H. chrysaspis Métrod, a whitish, sickly-smelling
fungus under beech. Results from examining the anatomy of the gills
appears to confirm these divisions. All the Hygrophori have a homogeneous
flesh, white spores, central, fleshy stem and thick, waxy gills;
microscopically this group of fungi can be recognised by the very
long basidia.
The following are common examples of the genus Hygrocybe:—
H. calyptraeformis (Berkeley & Broome)
Fayod has a rose-pink, conical
cap which expands to become upturned at the edge with age.
H. coccinea (Fries) Kummer
has a bright scarlet cap which becomes
yellow-ochre on drying and a yellow base to a scarlet stem.
H. conica (Fries) Kummer
has an orange to red stem and sharply
conical cap which turns blackish with age and whose gills when cut
exude a clear watery liquid.
H. flavescens (Kauffman) Singer
has a slimy, golden yellow cap and
similarly coloured stem.
H. chlorophana
is similar, but has a lemon-yellow cap and stem.
H. punicea (Fries) Kummer
is a large and robust species, similar in
colour to H. coccinea but with a white base to the stem.
H. unguinosa (Fries) Karsten
has a smoky grey, very slimy cap and
stem.
H. nitrata (Persoon) Wunsche
is as dull coloured as H. unguinosa, but
is not slimy, and in addition strongly smells of cleaning fluid or
bleaching-powder. It is one of three dull coloured, strong bleaching-powder-smelling
species found in Britain. H. ovina is another, but
is darker than H. nitrata and becomes red when bruised or cut.
Plate 27. Fleshy brightly coloured fungi: Spores white and borne on thick, waxy gills
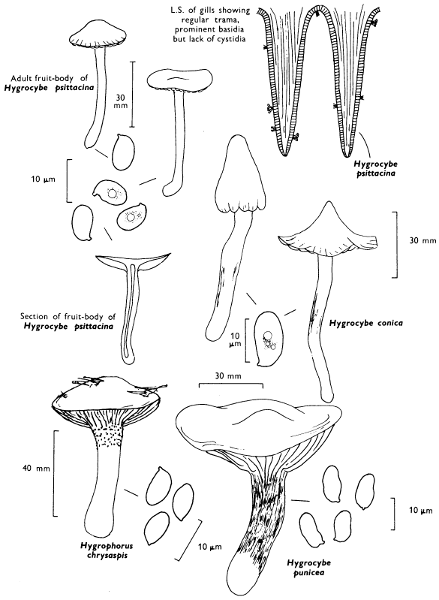
Larger illustration
H. metapodia (Fries) Moser
has a sooty brown fibrillose-streaky cap and
stem. The gills are distant and grey, and the fruit-body may reach
up to 100 mm across. It is probably the biggest of our native species
of Hygrocybe.
For completion examples of Hygrophorus include:
H. bresadolae Quélet
has a slimy orange-yellow cap, yellow gills and
yellow, slimy, smooth stem. It is found under larch trees.
H. chrysaspis Métrod
has ivory white cap, stem and gills which soon
become flushed with rust-brown and finally the whole fruit-body
becomes red-brown. The stem is slimy and white dotted at the apex.
It grows in beech woods.
H. hedrychii Velenovsky
has a slimy cream-coloured cap flushed with
pale peach colour. The gills and stem are cream and the latter slimy
and dotted at the top. It is found in pine woods.
H. hypothejus (Fries) Fries
has an olive-brown slimy cap, yellow stem
and gills; the stem is slimy and smooth. It is found in pine woods
and under pines on heaths.
H. pustulatus (Persoon) Fries
has an ash-grey cap brownish towards
its centre, viscid white stem with dark grey dots at the apex and
white gills. H. agathosmus (Secretan) Fries is similar, but smells
strongly of bitter almonds. Both species are found in plantations.
Species of the genus Hygrophorus are infrequently encountered in
Britain, although twenty species are recorded for the British Isles.
They are ecologically distinct from members of the genus Hygrocybe
in preferring woodland communities to grassland areas; they are
probably mycorrhizal. The anatomy of the fruit-body is also rather
different to that found in Hygrocybe; the gill-trama is bilateral as in
Leccinum (p. 27), Suillus (p. 28),
Boletus (p. 31), Chroogomphus
(p. 36), Paxillus (p. 38) and Amanita
(p. 54). Members of the
genus Hygrocybe have regular to irregular gill-tramas. In fact,
although both genera are united into a single family, the Hygrophoraceae
is based on one character common to both, i.e. the long
basidium; there is every indication that the genus Hygrocybe has
greater affinity to Omphalina in the Tricholomataceae (p. 232).
Surprisingly enough in North America many of our familiar
grassland species including H. pratensis are to be found in deep
shaded woodland!
Angular, pink-spored agarics—Rhodophyllaceae
The name of the family refers to the pink gills and it unites all those
fungi with a salmon-pinkish buff spore-print and whose spores are
angular in all optical sections. There are a few agarics, e.g. Clitopilus
prunulus (Fries) Kummer with ridged spores which appear angular in
end-on view, but which are ellipsoid in both side and face views and
so are considered less related.
The family Rhodophyllaceae by some authorities contains one genus
Rhodophyllus, more correctly called Entoloma; in the British Isles five
constituent genera are recognised, but they will have to be more
critically defined to make a more meaningful classification. At the
moment, many of the species are poorly documented and it would
appear that anatomical studies will assist in the future in the recognition
of species-groups.
If one selects the eight most distinctive shaped spore-types exhibited
in members of this family, then when their spores are examined side-on
a feature is available for correlation with the traditional field characters,
such as cap scaliness and gill-attachment. The most distinctive spore-shape
is Type G, found in Nolanea staurospora Bresadola, which is
probably the most common and widespread species of the family. It
grows in woodlands, grassland and on lawns and will be dealt with
later (p. 122). The other spore types are illustrated and range from
irregularly rhomboid to elongate angular.
The majority of the members of this group grow in grassland, hill-pastures
and meadows and distinct communities containing members
of this family and of the Hygrophoraceae can be recognised. It is not
proposed to deal in detail with any individual members because they
can be so easily confused with each other by the specialist let alone by
the amateur.
However, the genera as at present accepted are as follows:—
1. Entoloma
in its original sense contains agarics with fleshy caps,
fibrous stems and sinuate or adnexed gills, e.g. Ent. clypeatum (Fries)
Kummer with grey to yellow-brown cap, found growing with
members of the apple and rose-family in the summer and early
autumn. This genus corresponds to Calocybe in the white-spored
agarics (p. 110).
2. Leptonia
contains those agarics with rather thin caps whose margin
is incurved, cartilaginous stems and adnate to adnexed, rarely
decurrent, gills and whose cap flesh is indistinct from that of the
stem, e.g. Lept. serrulata (Fries) Kummer with dark blue to violet-blue
cap and dark blue edge to the gills. This genus approaches the
tough-shanks (Collybia) in the white-spored genera (p. 90).
3. Nolanea
is characterised by agarics with delicate caps, whose flesh
is distinct from that of the stem and whose edge is straight and
pressed against the fragile stem when young, and the adnexed or
adnate, rarely decurrent, gills, e.g. N. staurospora (see p. 122).
N. cetrata (Fries) Kummer with yellow-brown to tan-coloured cap
is found from spring to autumn in conifer woodland, especially
plantations. The genus corresponds to Mycena in the white-spored
agaric genera (p. 68).
4. Eccilia
is a small genus containing agarics with thin, membranous
caps and distinctly decurrent gills, e.g. E. sericeonitida P. D. Orton
with convex, then umbilicate, silky greyish brown cap. This genus
corresponds to Omphalina in the white-spored agarics (p. 232).
5. Claudopus
has three British representatives, all of which have a very
small stem which may even be absent, e.g. C. depluens (Fries)
Gillet grows on soil and C. parasiticus (Quélet) Ricken grows on
old decaying fruit-bodies of woody fungi. This genus corresponds to
Pleurotellus in the white-spored genera and to Crepidotus in the
brown-spored genera (p. 77).
Plate 28. Fleshy fungi: Spores pinkish and angular and borne on gills - Rhodophyllaceae
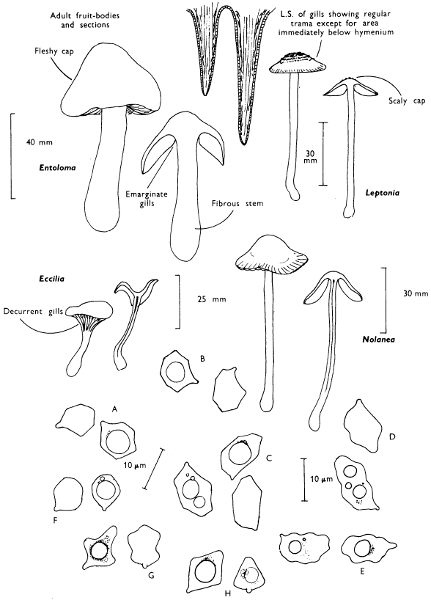
Larger illustration
Cystoderma amianthinum (Fries) Fayod
Cap: width 15-35 mm. Stem: width 4-8 mm; length 15-30 mm.
Description:
Cap: pale ochraceous yellow to sand-colour, convex then expanded,
with central umbo and often radially wrinkled-reticulate, covered
completely in powdery granules when fresh but these gradually
disappear with age or on excessive handling.
Stem: slender, white above a narrow, easily lost ring which is composed
of floccose, ochraceous yellow granules which also clothe the lower
part of the stem.
Gills: adnate, cream-coloured and crowded.
Flesh: yellowish with a strong smell of new-mown hay.
Spore-print: white.
Spores: small to medium sized, hyaline under the microscope, smooth,
ellipsoid, 5-7 × 3-4 µm and becoming blue-grey when mounted
in solutions containing iodine.
Marginal and facial cystidia: absent.
Habitat & Distribution: Frequently found amongst grass on heaths,
in hill-pastures and in woodlands from summer to autumn.
General Information: This fungus is recognised by the gill-attachment
and the powdery-scurfy cap formed by the breaking up of an
enveloping veil composed of thick-walled, rounded cells, similar to
those on the surface of the stem.
This fungus was formerly placed in the genus Lepiota because of
the ring but the veil in Cystoderma amianthinum is formed in quite
a different way to the ring in the true parasol mushrooms. The gills
are also adnate and not free as in the true species of Lepiota (see
p. 112). C. carcharias (Secretan) Fayod is found under similar conditions,
but is white or flesh-coloured. C. cinnabarinum (Secretan)
Fayod is also found in short grass and moss, but has a cinnabar-red,
floccose cap and C. granulosum (Fries) Fayod is yellowish brown
with non-amyloid spores and adnexed gills.
Many authorities prefer to connect this small group of closely
related species more to members of the Tricholomataceae (i.e. the
family which contains the Wood Blewits (p. 131), Mycena (p. 68,
etc.) than to the parasol mushrooms—Lepiota (p. 112).
Illustrations: Hvass 23; LH 129; NB 1037; WD 84.
Hygrophoropsis aurantiaca (Fries) Maire
False chanterelle
Cap: width 25-70 mm. Stem: width 4-7 mm; length 25-50 mm.
Description:
Cap: bright orange-yellow or apricot, fleshy, soft, depressed at centre
and with wavy, incurved, slightly downy margin.
Stem: yellow at apex, rich red-brown or orange about the middle and
sometimes dark brown at the very base.
Gills: decurrent, deep orange, thin, crowded, repeatedly forked and
easily separable from the cap-tissue.
Flesh: yellowish, pale in the cap, darker in the stem.
Spore-print: white.
Spores: medium sized, hyaline under the microscope, ellipsoid or
pip-shaped, smooth, 7-8 × 4 µm and red-brown when mounted in
solutions of iodine.
Marginal and facial cystidia: absent.
Habitat & Distribution: Common in woodlands, particularly with
pines, and on heaths or in rough hill-pastures.
General Information: This fungus is recognisable by the orange or
yellow cap and stem and the decurrent gills. It was formerly placed
in Cantharellus because of the colours, white spores and the decurrent
gills, but it really differs in many other respects. It is true, however,
that it is frequently confused with the true Chanterelle (Cantharellus
cibarius Fries, p. 162) by those who do not inspect their specimens
carefully. The gills are thin, plate-like as in other agarics and not
fold-like as in Cantharellus (see p. 162). The Chanterelle is edible
and sought after as a delicacy, but there are varying reports as to the
edibility of Hygrophoropsis. Certainly it is not of the best quality
and there is evidence for it causing upsets: therefore it is best to take
the name ‘False Chanterelle’ at face value and treat this fungus as
truely false; ‘aurantiaca’ means orange-coloured and refers to the
colour of the fungus.
A pale form is frequently collected, particularly in hill-pastures,
and is probably worthy of specific recognition. The cap is ochraceous
yellow to cream and the stem distinctly dark in the lower half.
There is some confusion as to the true position in classification of
this fungus. The anatomical details of the fruit-body parallel those
of Paxillus involutus (Fries) Fries (see p. 38) although the spore-print
is white. There is little doubt that future research will answer
this problem.
Illustrations: Hvass 183; LH 185; NB 1031; WD 163.
Agaricus campestris Fries
Field mushroom
Cap: width 40-100 mm. Stem: width 12-20 mm; length 40-80 mm.
Description:
Cap: rounded then expanding to become plano-convex, fleshy with the
margin incurved at first, initially pure white, but soon becoming cream-colour
and at maturity streaked brownish particularly at the centre.
Stem: white with a simple, very thin, white ring which becomes
brownish on rubbing and is easily lost with age or by handling.
Gills: free, pink but finally umber-brown at maturity.
Flesh: white, flushed reddish when cut especially in the stem.
Spore-print: cigar-brown, with hint of purple.
Spores: medium sized, ellipsoid or egg-shaped, smooth, small, 7-8 ×
4-5 µm and dark brown under the microscope.
Marginal and facial cystidia: absent. Basidia 4-spored.
Habitat & Distribution: The field-mushroom grows amongst grass in
pastures, etc., and also on old lawns where it may form fairy-rings.
General Information: This is the common wild, edible mushroom for
which many people have in the past unwisely substituted many quite
unrelated species. Deaths have often been caused by lack of careful
observation when selecting wild fungi for the table; this only
emphasises why white mushrooms found in fields should not be
casually eaten.
A. arvensis
Secretan the Horse-mushroom is also edible, but is
much bigger (up to 180 mm), creamy white and bruises slightly
yellowish on handling; it also has larger spores (7-10 × 5 µm),
club-shaped cells on the gill-edge, gills commencing white and not
pink, and the presence of a complex ring.
A. xanthodermus
Genevier the ‘Yellow-staining mushroom’ has even
smaller spores than the field mushroom, i.e. 5-6 × 4 µm and a
rather strong, unpleasant smell; if eaten many people subsequently
suffer from stomach-pains and this shows that even amongst those
fungi which the scientist would call true mushrooms, i.e. those
fungi in the genus Agaricus, there are some poisonous members.
Thus it is always necessary to have wide experience before one
collects fungi for eating and until this is achieved all specimens
should be discarded.
Illustrations: Field mushroom—Hvass 163; LH 133; NB 316; WD 712.
Horse mushroom—Hvass 160; LH 135; WD 721. Yellow-staining
mushroom—Hvass 159; WD 713.
Calocybe gambosum (Fries) Singer.
St George’s mushroom
Cap: width 70-100 mm. Stem: width 15-25 mm; length 50-70 mm.
Description:
Cap: creamy white, ivory or light buff, slightly darker at the centre
with age, fleshy, rounded and with wavy margin, finally expanding
to become plane-convex; the margin is incurved and slightly downy
at first.
Stem: firm, rather thick, white at the top, creamy or buff below and
slightly downy when fresh.
Gills: sinuate to adnexed with a slight decurrent tooth, white to
pale buff.
Flesh: with a very strong smell of meal, white and thick.
Spore-print: white.
Spores: small, ellipsoid, smooth, hyaline under the microscope, 5-6 ×
3-4 µm and not becoming blue-grey with solutions containing
iodine.
Marginal and facial cystidia: absent.
Habitat & Distribution: Found amongst grass in base rich pastures,
often in fairly large rings from April to June and on golf-courses
particularly those near the sea.
General Information: The common name refers to the early appearance
of this agaric; St George’s Day is April 23rd, and this mushroom
is found about this time in favourable years, its fruiting often extending
into early June, particularly if the fruiting is retarded by a
cold and wet spring. It is easily recognised by the pale colour of the
cap, strong mealy smell, but particularly by its appearance in spring.
In each new year it is probably the first of the larger agarics to
appear. This species will be found in most books under the genus
Tricholoma, but differs from typical members of this group in the
anatomy and chemistry of the gill-tissues.
The Latin name ‘gambosum’ is derived from ‘gamba’ meaning a
hoof and this reflects the shape of the fleshy cap as it pushes up
through the grass. Another much older name is Tricholoma georgii
(Fries) Quélet which was used by Clusius and is derived from the
legend of St George.
Illustrations: Hvass 28; LH 83; WD 92.
Lepiota procera (Fries) S. F. Gray
Parasol mushroom
Cap: width 70-200 mm. Stem: width 12-20 mm; length 100-250 mm.
Description:
Cap: dull brown or greyish brown, oval or rounded at first, but later
becoming bell-shaped, finally expanding but for the central umbo
and the surface breaking up into shaggy scales.
Stem: straight, tapering upwards from a slightly bulbous base, felty
at first but then the surface breaking up into small patches which
finally resemble the pattern of a snake-skin; there is also a large,
thick, white ring which is brown below and becomes loose on the
stem.
Gills: remote, white, crowded and fairly broad.
Flesh: white, thin, soft.
Spore-print: white.
Spores: very long, ellipsoid with a germ-pore, hyaline under the
microscope about 16 × 10 µm (14-17 × 9-12 µm), and becoming
reddish brown in solutions containing iodine.
Marginal cystidia: variable, elongate balloon-shaped and hyaline.
Facial cystidia: absent.
Habitat & Distribution: Found from summer until mid-autumn, on
the outskirts of copses, in fields, at edges of woodland or in woodland
clearings; it is sometimes found in very large rings.
General Information: When this fungus first appears through the soil
it resembles a drum-stick with the margin of the unexpanded cap
tightly hugging the stem. It is an easily recognised fungus because
of its straight and graceful stature with large cap and tall stem. It is
one of our best edible fungi and cannot be confused with any other
agaric. L. rhacodes (Vittadini) Quélet is not as elegant and has much
smaller spores.
Illustrations: F 26a; Hvass 15; LH 125; NB 311; WD 51.
Psilocybe semilanceata (Secretan) Kummer
Liberty caps
Cap: width 8-14 mm; height up to 18 mm. Stem: width 4-6 mm;
length 50-70 mm.
Description:
Cap: sharply conical, in fact often with a very distinct apical point,
never or very rarely becoming expanded, often fluted and puckered
at the incurved margin, smooth, viscid, pale buff or clay colour, but
soon flushed with greyish green at maturity and becoming free of
the fibrils of veil which ornament the margin when young.
Stem: slender, tough and smooth, similarly coloured to the cap and
sometimes blueing at the base when picked.
Gills: adnate to adnexed, crowded, purplish black except for white edge.
Flesh: white or pallid.
Spore-print: purple-brown.
Spores: long, ellipsoid, slightly lemon-shaped, smooth and with a
distinct germ-pore at one end and 12-14 × 7 µm in size.
Marginal cystidia: bottle-shaped with an elongate tapering neck,
with thin walls which at most become pale honey in solutions containing
ammonia, unlike the cystidia of Hypholoma (p. 64).
Habitat & Distribution: Commonly growing amongst grass in fields
near farm-yards, on heaths and by roadsides; often it occurs in
small troops.
General Information: Psilocybe semilanceata is recognised by the uniquely
shaped cap; ‘semilanceata’ means half spear-shaped, from the
papilla at the top of the cap, giving it a pointed aspect. However,
the common name is more descriptive and comes from the fact that
these caps resemble the helmets worn by French soldiers in the
early part of the century.
This fungus was once very isolated amongst British agarics, but
now it has been united with a group of small purplish brown-spored
fungi formerly placed in the genus Deconica. What is of more
interest is the fact that unlike many British agarics the cap often
does not expand fully in order to release the spores. In this way it
allows mycologists to hypothesise on how certain of the enclosed,
stalked Gastromycetes evolved in some of the desert regions of the
world.
Illustrations: LH 149; NB 3311; WD 787.
Conocybe tenera (Fries) Fayod
Brown cone-cap
Cap: width 10-20 mm. Stem: width 3-6 mm; length 70-100 mm.
Description:
Cap: very hygrophanous, sand colour, orange-yellow or ochraceous
brown tinted cinnamon when fresh but drying uniformly yellow-ochre,
thin, fragile, striate when moist, but soon non-striate as water
is lost from the cap.
Stem: tall, slender and similarly coloured to the cap, straight, fragile,
minutely striate from the top to bottom with what appears to be
minute powdery granules.
Gills: adnate then becoming free, crowded, ochraceous and finally
cinnamon-rust in colour.
Flesh: russet when moist but rapidly becoming yellowish as the fruit-body
dries.
Spore-print: rust-brown.
Spores: long, ellipsoid, with thick, bright yellow-brown walls and
distinct germ-pores at their ends when seen under the microscope,
and over 10 µm in length (11-12 × 6 µm.)
Marginal cystidia: pinheaded or skittle-shaped.
Facial cystidia: absent.
Habitat & Distribution: This fungus grows in ones and twos, more rarely
in troops amongst grass.
General Information: This is one member of a whole complex group
of ochraceous, brown, tawny or cinnamon-brown capped agarics
which superficially appear to be the same, but on closer examination
the expert can split them into several distinct species.
The use of microscopic characters is essential and outside the scope
of this book or the ordinary mushroom-picker’s manual. However,
the closely related C. lactea (J. Lange) Métrod can be more easily
distinguished for it has a white or cream-coloured cap and stem.
It also has larger broadly ellipsoid spores, measuring 12-14 × 6-9
µm, but the same shaped cells on the gill-edge.
Illustrations: LH 153; NB 354; WD 682.
Many agarics grow in circles, but not all of them produce zones in the
vegetation. It is the distinct zonation caused by the ‘fairy-ring champignon’
Marasmius oreades (Fries) Fries and related fungi which have
given rise to the name of Fairy-ring and which resulted in the foundation
of many folk tales.
A fairy-ring can be divided into four distinct zones, a central zone of
fairly normally developed vegetation on the outside of which is a
green, actively growing zone of grass; outside this is a zone composed
of brown or dead vegetation. The outermost zone again appears to
be far more lush than the normal grass in the vicinity and it is in this
last zone that the fruit-bodies of the fungus causing the pattern
appear.
A generalised explanation of the zoning appears to be as follows:—
In the outermost zone the actively growing mycelium decomposes
soil constituents and liberates nitrogenous material which is in turn
taken up by the plant roots nearby and utilised for their growth. In the
penultimate zone the grass is dead, probably not caused by a direct
parasitic attack but by the mycelial threads filling the air-spaces in the
soil and so inhibiting water flow. This destruction of the delicate balance
of water and air found in any soil induces drying out and gradual death
of the plants whose roots permeate the soil. Behind the dead-zone is
vegetation which shows increased vigour apparently due to plant-nutrients
being released by the decaying mycelium and plant-material,
whose death has been caused by the presence of the fungus. The
innermost zone is not so stimulated.
With nothing more than graph and tracing paper, a tape-measure,
note-book and pencil, pieces of cane about four inches long, and
coloured dye or indian ink, it is exciting to assess the annual radial
growth of fairy-rings and to correlate these with environmental conditions.
This can be carried out on a school lawn or on a home lawn;
the method and further experiments are given in Appendix iii.
Marasmius oreades (Fries) Fries
Fairy-ring champignon
Cap: width 25-60 mm. Stem: width 5-9 mm; length 30-80 mm.
Description:
Cap: pinkish tan with slight flush of brown at centre, hygrophanous
and drying out buff-coloured or clay-coloured, convex at first then
expanding to become plane, but for an obtuse umbo which is
retained at the centre.
Stem: pale buff, tough, flexible and smooth.
Gills: adnexed, pale cream colour or pinkish buff and fairly distant.
Flesh: whitish or pinkish tan, smelling of cherry laurel (cyanic).
Spore-print: white.
Spores: medium sized, hyaline, pip-shaped, smooth, not staining
bluish grey when mounted in solutions containing iodine and about
10 × 6 µm in size (9-11 × 5-6 µm).
Marginal and facial cystidia: absent.
Habitat & Distribution: This agaric is very common from May to
October on lawns and grass-verges.
General Information: M. oreades forms well developed fairy-rings, and
is easily recognised by its tough nature, pale colours and ability to
revive after having been dried. This ability to revive in moist weather
even after the fruit-body has been dried by the sun or wind is a
character which was used to distinguish members of the genus
Marasmius. However, this is a very subjective character and since
microscopic techniques were introduced and used widely in the
study of agarics the genus has been delimited rather more critically.
Marasmius is close to Collybia (p. 90), in fact many species
appear in one book in one genus and in another book in the second
genus; M. oreades itself is not a typical member of the genus.
Marasmius seems to be a much more important genus in the tropical
and subtropical regions of the world; we have already mentioned
how some of the small species of Marasmius in Europe grow only
on leaves of a particular plant (see p. 92). M. androsaceus (Fries)
Fries (see p. 231) is the horse-hair fungus.
Illustrations: F 19a; Hvass 81; LH 115; NB 351; WD 2410 (not very
good).
Plate 37. Fleshy fungi reviving when moistened even after drying: Spores white and borne on gills
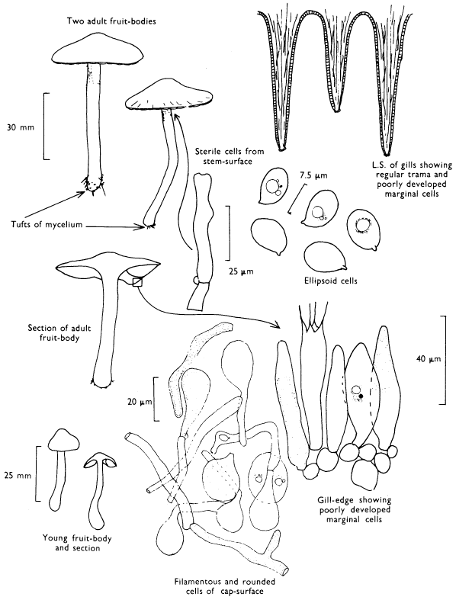
Larger illustration
Nolanea staurospora Bresadola
Cap: width 20-40 mm. Stem: width 3-5 mm; length 45-70 mm.
Description:
Cap: bell-shaped at first then expanded, hygrophanous, date-brown,
striate when moist but pale fawn or tan and non-striate when dry,
and usually becoming quite silky-shiny.
Stem: slender, fragile, greyish brown, silky fibrillose-striate and shiny.
Gills: almost free, crowded and pale greyish brown when young, but
finally flesh coloured.
Flesh: brownish and smelling very strongly of meal when cut or broken
between the fingers.
Spore-print: salmon-pink with flush of cinnamon.
Spores: medium sized, fawn under the microscope, star-shaped with
4-6 prominent angles, 9-10 × 7-9 µm, smooth and with no germ-pore.
Marginal and facial cystidia: absent.
Nolanea sericea (Mérat) P. D. Orton
Silky nolanea
Cap: width 25-40 mm. Stem: width 5-9 mm; length 25-50 mm.
Description:
Cap: convex then flattened or with slight umbo, umber-brown with
a greyish cast which becomes accentuated as the cap dries out and
finally becoming silky-shiny; the margin is incurved and striate at
first but on expanding it becomes non-striate with time.
Stem: short, fibrillose, greyish brown, shining and white at the base,
very fragile and often snaps just above the soil-level when collected.
Gills: crowded, adnate and pale greyish brown then pinkish brown.
Flesh: with a strong smell of new meal, brownish becoming paler as
it dries out.
Spore-print: salmon-pink.
Spores: medium sized, smooth, pale fawn under the microscope,
angular almost cubic and 10-13 × 8-9 µm in size.
Marginal and facial cystidia: absent.
General Information: Nolanea staurospora is very common amongst
grass, in many habitats such as on heaths, and in woodlands and
copses, but it is particularly common in pastures and on lawns.
It is difficult to separate from close relatives on field-characters,
except for the strong mealy smell; however, it is recognised immediately
by the spore-shape, in fact stauro—means a cross and spora—spore!
Because of the flattened cap and gill-shape N. sericea (Mérat)
P. D. Orton was first placed in Entoloma, but for a long time it was
one of the smallest members of that genus. The European species
of Nolanea have recently been critically analysed, and now that
closely related species to the silky Nolanea have been found, it
appears better placed in Nolanea although it is still found under
Entoloma in many books. The Latin word ‘sericeum’ means silky
and refers to the silky cap and stem of this fungus which is a very
noticeable feature when the fungus is collected in the dry state.
The common name which has been given to this fungus also refers
to the silky nature of the fruit-body.
Illustrations: N. staurospora—LH 181; ND 312; WD 522.
N. sericea—LH
181; WD 525.
Panaeolus foenisecii (Fries) Schroeter
Brown hay-cap
Cap: width 12-28 mm. Stem: width 3-6 mm; length 40-60 mm.
Description:
Cap: semiglobate to convex and hardly expanding even with age,
smooth, expallent, dull cinnamon-brown or dark tan-colour, becoming
clay-colour or pale cinnamon-colour from centre outwards
on drying and so sometimes appearing as if it is zoned.
Stem: slender, fragile, smooth and pale cinnamon-brown, except at
apex where it is dotted with white; it is usually more brownish below.
Gills: adnate, crowded, pale brown and mottled, but becoming more
uniformly umber-brown except for whitish margin.
Flesh: whitish or pale cinnamon colour.
Spore-print: purple-brown.
Spores: long, lemon-shaped under the microscope, dull brown,
warted all over but for the distinct germ-pore; 12-15 × 7-8 µm in
size.
Marginal cystidia: variable spindle-shaped with flexuous neck and subcapitate
apex, about 5-6 µm wide.
Facial cystidia: absent.
Habitat & Distribution: Common amongst short grass on lawns, in
pastures, on grass-verges, etc., from May until October.
General Information: P. foenisecii is recognised under the microscope
by the ornamented spores; this character was used to separate this
fungus in the new genus Panaeolina. However, although the spore-print
is not exactly black the stature, mottled gills and anatomy
conform closely with Panaeolus sphinctrinus (Fries) Quélet and
P. rickenii Hora (see p. 210 and below respectively). The same
fungus has been placed in Psilocybe (see p. 114), but it has little in
common with members of that genus. The word ‘foenisecii’ means
hay-harvest, reflecting the habitat of growing in fields. This fungus
is variable in colour depending on its state of turgidity; it can be
easily confused with other species of Panaeolus when moist and with
certain species of Conocybe when dry. P. rickenii is an equally
common agaric growing on similar or slightly less base-rich soil-types.
It has a distinctly bell-shaped reddish brown cap with a pale
incurved margin which in wet weather is, like the entire stem,
beaded with droplets of liquid. This gives the fungus a glistening
appearance when seen fresh and as it dries these droplets are lost
and the cap becomes slightly zoned. The stem is pale reddish-brown
with a strong frosted appearance because of the minute hairs which
cover it. I have no doubt that the classification of these fungi will
be assisted by careful analysis of the shapes of the hairs found in
the different species.
Illustrations: Panaeolina foenisecii—LH 145; WD 784. Panaeolus
rickenii—LH 145.
Coprinus comatus (Fries) S. F. Gray
Lawyer’s wig
Cap: width 30-60 mm; height 80-200 mm. Stem: width 10-20 mm;
length 80-250 mm.
Description: Plate 40.
Cap: at first cylindrical or oval then bell-shaped, fleshy, fragile, white
and covered with woolly, whitish, shaggy scales which have brown
tips; the centre of the cap is smooth and yellow to ochraceous
whilst the margin becomes striate and lilaceous and finally black
as the tissue liquefies (autodigests) and the margin rolls up to expose
new areas of spore-bearing tissue.
Stem: tall, white, smooth and tapered towards the apex, with a white
ring which can easily move up and down the stem with handling,
and which soon disappears with age.
Plate 40. Fleshy fungi becoming reduced to an inky mass:
Spores black and borne on gills
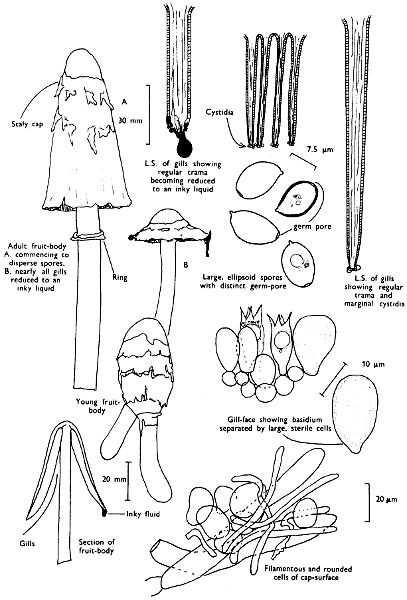
Larger illustration
Gills: free at first, white then pink and finally black, becoming gradually
dissolved into a black fluid from the base of the cap upwards.
Flesh: white, thin, except immediately in the central area of the cap.
Spore-print: blackish-purple.
Spores: long, elongate-ellipsoid, large and about 13 × 5-8 µm in size,
(12-15 × 7-9 µm).
Marginal cystidia: elongate club-shaped to balloon-shaped, hyaline
and thin-walled.
Facial cystidia: absent.
Habitat & Distribution: Grows in clusters on rich ground, in gardens,
on sides of newly prepared roads and central reservations of motor-ways,
on path-sides, in cultivated fields and on rubbish dumps;
it grows from spring to autumn and sometimes occurs in huge
troops.
General Information: Easily recognised by its size, the shape of the
cap with its scaly surface and from its resemblance to a ‘judge’s
wig’; it is frequently called the ‘lawyer’s wig’ and whereas some
common names are not very descriptive and one has to use a lot of
imagination to conjure up what the common name implies, in this
case it is not so. It is also known as the ‘shaggy cap’ or ‘shaggy
ink-cap’. Ink or inky cap is, however, a common name for many
species of the genus Coprinus (see p. 211-4).
The unrelated Lyophyllum decastes (Fries) Singer and L. connatum
(Fries) Singer are also common fungi growing on roadsides, on soil
and compost-heaps. They too break through embankments, soil,
paths, etc., producing large craters and mounds of debris.
Illustrations: Coprinus comatus—F 34b; Hvass 172; LH 137; NB 355;
WD 822. Lyophyllum decastes—LH 81; WD 142.
Lacrymaria velutina (Fries) Konrad & Maublanc
Weeping widow
Cap: width 45-90 mm. Stem: width 8-14 mm; length 50-125 mm.
Description: Plate 41.
Cap: convex then expanded with obtuse central umbo, dull clay-brown
or date-brown and at first covered with flattened, woolly fibrils
which are gradually lost with age; the margin is incurved and
fringed with remnants of the veil.
Stem: fragile, pale dingy-coloured or clay-coloured at apex, dull
brown below the ring-zone which consists of white fibrils; later in
development these fibrils catch the spores and the stem becomes
black and fibrillose-scaly, particularly below the ring-zone.
Gills: sinuate, crowded and very dark brown or almost black with
distinct white margin which is covered in tiny beads of liquid in
moist weather.
Flesh: pale buff.
Spore-print: almost black.
Spores: long, dark brown, lemon-shaped and warted with distinct and
prominent germ-pore and 10-12 × 6-7 µm in size.
Marginal cystidia: club-shaped or with a distinctly rounded head.
Facial cystidia: absent.
Habitat & Distribution: Common on the ground near newly built
houses, on roadsides, tips and paths in woods, either solitary or
in groups; it is also found in pastures.
General Information: The fibrillose scaly cap and stem and the almost
black gills which frequently have liquid droplets at their edge
separate this species from all other agarics and microscopically it
can be easily recognised by the warted spores. ‘Velutina’ means
velvety and refers to the texture of the cap-surface, of the young
fruit-body. The genus name Lacrymaria refers to this peculiar, but
certainly not unique, phenomenon, of exuding liquid from cells on
the gill-edge. This has been compared with weeping and ‘lacrymans’
means weeping; the common name reflects this also—weeping widow
(cf. p. 154).
This fungus has had a chequered history, for it is also known in
some books as Hypholoma lacrymabunda (again meaning weeping)
or H. velutina; the anatomy of the fungus, however, is quite different
to Hypholoma (e.g. H. fasciculare p. 64). More recently it has found
a place in Psathyrella, but it seems unsatisfactorily placed there because
of the warty spores, black spore-print and fibrillose cap-surface;
it warrants a separate genus, i.e., Lacrymaria. L. pyrotricha (Fries)
Konrad & Maublanc is the only other British species of this genus
but it has a bright orange cap colour; it is rare.
Illustrations: Hvass 180; LH 141; WD 863.
Lepista nuda (Fries) Cooke
Wood blewits
Cap: width 70-100 mm. Stem: width 10-15 mm; length 70-100 mm.
Description: Plate 42.
Cap: rounded then flattened or slightly depressed in the centre,
smooth, bluish lilac, or violaceous when young but gradually with
age becoming reddish-brown, with or without a flush of wine colour.
Stem: similarly coloured to the cap, equal, fleshy, elastic, fibrillose
and streaky.
Gills: adnate with or without a decurrent tooth, crowded, lilac and
easily separable from the cap-tissue by the fingers.
Flesh: bluish violaceous, but drying out dirty buff in the base of the
stem.
Spore-print: flesh-coloured.
Spores: medium-sized, ellipsoid appearing smooth but very minutely
roughened under the microscope, although it is very difficult to see
except with a good instrument (6-8 × 4-5 µm in size).
Marginal and facial cystidia: absent.
Habitat & Distribution: Widespread in troops or small groups in copses
and under hedgerows and not uncommon in flower-beds in gardens
in late autumn and early winter especially on compost heaps and in
rhubarb patches which have been mulched with piles of moribund
leaves.
General Information: This fungus was originally placed in Tricholoma,
but due to differences in anatomy and the distinctly coloured and
ornamented spores it has been placed along with ‘common blewits’
T. personatum (Fries) Kummer (or better L. saeva (Fries) P. D.
Orton), in the genus Lepista. This genus which is also called Rhodopaxillus,
again referring to the pinkish spore-print, is not found in
many of the easily obtainable books. One should look for the fungus
under Tricholoma, from which it can be separated easily by the
beautiful colour.
Both the ‘wood blewits’ and ‘common blewits’ have been regularly
sold in markets in England within the last fifty years. They are
edible and considered of high quality. In their fresh state they are
easily recognised, but as they age they become browned and so
resemble many other less desirable fungi.
Illustrations: F 17d; Hvass 49; LH 91; NB 1252; WD 123 (a bit too
pastel).
Agaricus bisporus (J. Lange) Pilát
Common mushroom
Cap: width 40-100 mm. Stem: width 15-25 mm; length 50-75 mm.
Description: Plate 43.
Cap: rounded gradually expanding to become plane, whitish with
numerous brown radiating fibrils and with the margin irregular
because of fragments from the ring which are left there after expansion
of the cap.
Stem: short, cylindrical, smooth, bruising reddish-brown when handled
and with a narrow ring which soon collapses and disappears.
Gills: free, pink at first then purple-brown, narrow and crowded.
Flesh: solid, thick, firm and slowly flushing brownish on cutting.
Spore-print: purple-brown.
Spores: medium-sized, broadly ellipsoid, purple-brown under the
microscope, less than 10 µm long, (6-8 × 5-6 µm).
Marginal cystidia: club-shaped, 10-12 µm at apex.
Facial cystidia: absent.
Basidia: 2-spored.
Habitat & Distribution: Frequent on manure heaps, straw heaps, on
road scrapings and around garden plants.
General Information: This fungus is recognised by the dark fibrils on
the cap, the 2-spored basidia easily seen with the low power of a
microscope, and the pink gills when young. Much confusion has
existed over this fungus and its nearest relatives. It is similar to
the ‘Cultivated mushroom’, A. hortensis (Cooke) Pilát, which is offered
for sale in shops. However, it differs in several minor details and it
may be that A. bisporus is the fungus from which the cultivated
mushroom developed, very probably unconsciously by man, but the
history of the cultivated mushroom is very obscure. The cultivated
mushroom when bought in British shops is white but in the United
States two varieties are sold, one with the brownish fibrils predominating
and a snow-white one where the fibrils do not darken;
the former is frequently found in Europe. The white form is sometimes
found in gardens where spent-mushroom spawn is used as
mulching around fruit-trees but it has a rounder cap than A. bisporus.
The cultivated mushroom accounts for an annual income of £14
million in the British Isles.
Illustrations: A. hortensis—LH 133 (as the forma albida); NB 317;
WD 711. A. bisporus—Hvass 161; LH 133.