Gastric digestion is essentially an acid digestion. As a
proteolytic agent, pepsin can act only in the presence of
acid, and we have every reason for believing that the
enzyme and the acid form a compound, which in turn combines
with the proteid undergoing digestion; or, what
amounts to much the same thing, that the acid perhaps
forms first a compound with the proteid, to which the pepsin
can then unite to form a still more complex compound
capable of undergoing hydration and cleavage. Pepsin-proteolysis,
therefore, is strictly the proteolysis produced
by pepsin-acid. In view of this fact, we may well give a
moment’s thought to the nature and origin of this acid.
Without attempting any statement of the gradual development
of our knowledge regarding the acid of the gastric
juice, we may accept the now well-established fact that the
acid is hydrochloric acid, and that it has its origin in the
parietal, or so-called border-cells of the gastric glands.
That the acid is derived from the decomposition of chlorides
is practically self-evident, but Cahn94 has added experimental
proof which removes all shadow of doubt, through
his study of the gastric secretion in animals deprived for
many days of salt; the gastric juice in such cases being perfectly
neutral in reaction, but normal as regards its content
of pepsin.
The way in which the specific gland-cells manufacture
free hydrochloric acid out of material contained in an alkaline
medium is somewhat doubtful. There are, however,
at the present day two theories worthy of special notice.
The first is based upon observations made by Maly95 many
years ago, which tend to show that certain mineral salts
present in the blood are capable of reacting upon each
other with formation of hydrochloric acid. Thus, while
the blood is an alkaline fluid, it really owes its alkalinity to
the presence of two acid salts, viz., sodium bicarbonate
(HNaCO3) and disodium hydrogen phosphate (HNa2PO4).
This latter compound, acted upon by the carbonic acid of
the blood, is transformed into a dihydrogen sodium phosphate
with simultaneous formation of acid sodium carbonate,
as shown in the following equation:
Na2HPO4 + CO2 + H2O = NaH2PO4 + HNaCO3.
This acid sodium phosphate dissolved in a fluid containing
sodium chloride, gives rise to free hydrochloric acid by a
very simple reaction:
NaH2PO4 + NaCl = Na2HPO4 + HCl.
It is also to be noted that the disodium hydrogen phosphate,
may, likewise, give rise to hydrochloric acid through
its action on calcium chloride, as indicated by the following
equation:
2Na2HPO4 + 3CaCl2 = Ca3(PO4)2 + 4NaCl + 2HCl.
It is thus evident that hydrochloric acid may originate
in the inter-reaction of these several salts which are known
to be present in the blood; but obviously, the above reactions
cannot take place in the blood itself, and we must
look to the selective power of the epithelial cells of the
gastric glands, as suggested by Gamgee,96 for the withdrawal
of the needed salts from the blood. Once present
in the acid-forming cells, and perhaps aided by the inherent
qualities of the protoplasm, the necessary chemical
reactions may be assumed to take place, after which the
newly formed acid may pass from the gland-cells into the
secretion of the gland.
A later theory regarding the formation of the acid of the
gastric juice emanates from Liebermann.97 This investigator
claims the existence in the mucous membrane of the
stomach of an acid-reacting, nuclein-like body, which is
apparently a combination of the phosphorized substance
lecithin with a proteid. To this compound body Liebermann
gives the name of lecithalbumin. It is apparently
located in the nuclei of the gastric cells, is strongly acid in
reaction, and, according to Liebermann, is an important
agent in the production of the free hydrochloric acid of the
gastric juice, although its action is somewhat indirect.
According to this theory, the free acid is formed in the
mucous membrane of the stomach from sodium chloride,
through the dissociating action of the carbonic acid coming
from normal oxidation. The thus-formed acid then diffuses
in both directions, viz., through the lumen of the gland
into the stomach-cavity, and in part in the opposite direction
into the veins and lymphatics. It is the assumed
function of the lecithalbumin to react with the alkaline
sodium carbonate, produced simultaneously with the hydrochloric
acid. This naturally gives rise to the liberation of
carbonic acid and to the formation of a non-diffusible
sodium-lecithalbumin compound, which is retained for the
time being in the body of the cell. When the circulation
of the blood, accelerated by the digestive process, returns
to its ordinary pace, this latter compound is slowly decomposed
by the carbonic acid with formation of the readily
diffusible sodium carbonate, which passes into the blood-current.
The rate of this latter reaction is impeded, or,
perhaps regulated, by the swelling up of the lecithalbumin-containing
cells, thus rendering the imbibition of the
carbonic acid a slow process. The rate of production of
the hydrochloric acid by this hypothetical process depends
primarily upon the blood supply, and the oxidative changes
by which carbonic acid is formed.
There is much that might be said for and against this
theory,98 but we cannot stop to discuss it here. Like the
previous theory, it implies the production of hydrochloric
acid from a chloride or chlorides, through chemical processes
taking place in the stomach-mucosa, and presumably
in the large border-cells of the peptic glands. This hydrochloric
acid, as you know, in the act of secretion, reacts
upon the pepsinogen with which it may come in contact,
transforming it into pepsin. It also has the power of combining
with all forms of proteid matter, not excepting the
products of proteolytic action, to form acid compounds in
which the so-combined acid, although equal quantitatively
to the original amount of free acid, is less active in many
ways. Thus, it does not possess in the same degree a
destructive action on the amylolytic ferments;99 it does not
play the same part in aiding the proteolytic action of pepsin,
and its antiseptic power is far from equal to that of a
like amount of free acid.100
With relatively large amounts of proteid, we may have
half or even quarter saturated proteid molecules, in which
the weakness of the combined acid is far more pronounced
than in the case of the fully saturated molecule. Such a
condition of things must obviously exist in the early
stages of gastric digestion. With an excess of proteid
matter in the stomach, some time must elapse before the
secretion of hydrochloric acid will be sufficient to furnish
acid for all of the proteid matter present, yet pepsin-proteolysis
does not wait the appearance of free acid. Indeed,
the proteid matter may not have combined with more than
half its complement of hydrochloric acid before digestive
proteolysis is well under way. I have made many analyses
of the stomach-contents after test meals, and under
other conditions, where no free acid could be detected by
the tropaeolin test, or better, by Günzburg’s reagent (phloroglucin-vanillin),
although phenolphthalein as well as litmus
showed strong acid reaction, and yet not only could
acid-albumin be detected in the filtered fluid, but likewise
proteoses and peptones. In other words, pepsin-proteolysis
can proceed in the absence of free hydrochloric acid,
although not at the same pace. Hence, proteoses and even
peptones may make their appearance in the stomach-contents
at a very early period of digestion, i. e., the final products
of proteolysis may be found in a mixture containing
even a large proportion of wholly unaltered proteid,
and obviously at an early stage in the process.
Expressed in other language, a portion of the first formed
acid-albumin or syntonin may be carried forward by the
digestive process to the secondary proteose and peptone
stage, before the larger portion of the ingested proteid food
has even combined with sufficient acid to insure the complete
formation of acid-albumin. This introduces another
factor, to be referred to later on, viz., the relative combining
power of different forms of proteid matter, especially the
proteoses and peptones, as contrasted with native proteids.
In proof of the statement that pepsin-proteolysis can proceed
in the absence of free hydrochloric acid, provided combined
acid be present, allow me to cite one or two experiments
bearing on this point. A perfectly neutral solution
of egg-albumen, containing 0.8169 gramme of ash-free
albumin per 10 c.c. of fluid, was employed as the proteid
material. In order to completely saturate the proteid contained
in 20 c.c. of this neutral albumen solution, 50 c.c. of
0.2 per cent. HCl were required. Two mixtures were
then prepared as follows:
A. Twenty c.c. of the neutral albumen solution + 50 c.c.
0.2 per cent. HCl + 30 c.c. of a weak aqueous solution of
pepsin, perfectly neutral to litmus. This mixture gave
only the faintest tinge of a reaction for free acid when
tested by Günzburg’s reagent.
B. Twenty c.c. of the neutral albumen solution + 25 c.c.
0.2 per cent. HCl + 30 c.c. of the neutral pepsin solution.
In this mixture, the proteid matter was obviously only half
saturated with acid.
The two solutions were placed in a bath at 40° C.,
where they were allowed to remain for forty-four hours, a
little thymol being added to guard against any possible
putrefactive changes. At the end of this time the amount
of undigested albumin was accurately determined. The 20 c.c.
of original albumen solution contained 1.6338 grammes
of dry coagulable albumin. At the end of the forty-four
hours, A contained only 0.5430 gramme of unaltered albumin,
or acid-albumin, while B contained 1.2225 grammes.
That is to say, in the mixture A, where the acid existed
wholly in the form of combined acid, but with the albumin
completely saturated, 1.0908 grammes of the proteid were
converted into soluble albumoses and peptones. In B, on
the other hand, where the albumin was only half saturated
with acid, 0.4113 gramme of the proteid was converted
into soluble products. This difference in action is made
more striking by the statement that where the proteid was
only half saturated with acid, 25.1 per cent. of the albumin
was digested; while with a complete saturation of the proteid,
66.7 per cent. of the albumin was digested.
To give emphasis to this matter, a second experiment
may be quoted as follows: The proteid used was the
same neutral solution of egg-albumen containing 0.8169
gramme of albumin per 10 c.c. Two mixtures were prepared
as follows:
A. Ten c.c. of the neutral albumen solution + 21.7 c.c.
0.2 per cent. HCl, the amount needed to completely saturate
the proteid, + 40 c.c. of a weak solution of pepsin,
perfectly neutral.
B. Ten c.c. of the albumen solution + 10.9 c.c. 0.2 per
cent. HCl + 40 c.c. of the pepsin solution, making a mixture
half saturated with acid.
These two solutions were warmed at 40° C. for seventeen
hours. The extent of digestive action was then determined,
when it was found that in A only 0.1638 gramme
of the proteid was undigested, while in B, 0.6088 gramme
remained unaltered. In other words, where the proteid
was completely saturated with acid, but with an utter lack
of free acid, 79.9 per cent. of the albumin was converted
into albumoses and peptone, while in the mixture half saturated
with acid only 25.4 per cent. was digested.
These two experiments thus give striking proof that free
acid is not absolutely essential for pepsin-proteolysis.
Digestion is, to be sure, more rapid and complete when
free hydrochloric acid is present, but proteolysis is still
possible, and even vigorous, when there is a marked deficiency
of free acid. Further, as we have seen, proteolysis
may proceed to a certain extent even though the amount
of acid available is not sufficient to combine with more
than half the proteid matter present.
These facts at once raise the question whether the products
of proteolysis may not have a stronger affinity for acid
than the native proteids; an affinity so strong that they may
be able to withdraw acid from the acid-albumin first formed.
One of our conceptions regarding pepsin-proteolysis is that
acid is necessary for every step in the proteolytic process.
A primary albumose, for example, cannot be further
changed by pepsin, unless there is acid present for it to
combine with. This being true, it is clear, in view of the
fact that even peptones may appear in a digestive mixture
containing an amount of acid insufficient to combine even
with the albumin present, that the products of proteolysis
must withdraw acid from the acid-albumin first formed. In
regard to the first point, my own experiments certainly
tend to show that the products of gastric digestion do combine
with larger amounts of hydrochloric acid than undigested
proteids; and further, that of the several products
of proteolysis, the secondary proteoses combine with a
larger percentage of acid than the primary proteoses,
while true peptones combine with still larger amounts.
In other words, the simpler and more soluble the proteid,
the larger the amount of acid it is capable of combining
with; a statement which accords with results obtained by
other workers101 in this direction. Further, another factor
of considerable importance in connection with the
natural digestive process is that a dissolved proteid, such
as protoalbumose for example, will combine more readily
with free acid than an insoluble proteid; from which
Gillespie102 is led to infer that in pepsin-proteolysis where
there is no free acid present, only acid-albumin, proteoses
may be formed to a limited extent at the expense of some
of the acid of the acid-albumin, a portion of the latter being
perhaps reconverted into albumin. The ability of the proteoses,
however, to withdraw acid from its combination
with a native proteid is perhaps best indicated by Kossler’s103
experiments, which show that a solution of acid-albumin
containing only enough hydrochloric acid to hold the albumin
dissolved, on being warmed at 40° C. for some hours
with addition of a neutral solution of pepsin, may undergo
partial conversion into albumose or peptone.
In spite of these facts, there is some evidence that while
proteoses and peptones have the power of combining with
more acid than a like weight of native proteid, the latter,
leaving out all action of the pepsin, has a stronger affinity
for the acid; in fact, the firmness or strength of the union
appears to diminish as the products become simpler.104
Hence, a peptone separated from a digestive mixture, will
part with its combined acid somewhat more readily than
acid-albumin for example, although on this point there is
not complete unanimity of opinion.105 In digestive proteolysis,
however, where the pepsin is accompanied by a
minimal amount of hydrochloric acid, insufficient perhaps
to even half saturate the proteid present, the formation of
proteoses and peptones must be accompanied by a withdrawal
of acid from its combination with the native
proteid.
In illustration of some of these points, and especially of
the statement that the products of gastric digestion have
the power of combining with more hydrochloric acid than
the original proteid, allow me to cite the following experiment:
10 c.c. of a neutral solution of egg-albumen containing
about 0.82 gramme of pure dry albumin, free from
mineral salts, required 23.8 c.c. of 0.2 per cent. hydrochloric
acid to completely saturate the proteid matter. A
mixture was then prepared as follows: 10 c.c. of the
albumen + 24 c.c. 0.2 per cent. HCl + 30 c.c. of a neutral
pepsin solution, the mixture showing a faint trace of free
acid when tested by Günzburg’s reagent. This solution
was placed in a thermostat at 38° C., and from time to
time a drop of the fluid was removed and tested for free
acid. If no reaction could be obtained, 0.2 per cent.
hydrochloric acid was added to the mixture, until Günzburg’s
reagent showed free acid to be again present. The
following table shows the rate of disappearance of free
acid, and the amounts of 0.2 per cent. HCl required to
make good the deficiency. The mixture was placed at
38° C. on February 6th, at 11.30 A.M., and, as stated, contained
a trace of free acid, 24 c.c. 0.2 per cent. HCl having
been added to accomplish this result.
| Time. | Acid added to show trace of free acid. |
| February 6, | 11.30 A.M. | |
| " | 2.15 P.M. | | 4.5 | c.c., | 0.2 | per cent. | HCl. | |
| " | 5.00 P.M. | | 1.0 | " | " | " | " | |
| February 7, | 8.45 A.M. | | 3.0 | " | " | " | " | |
| " | 2.00 P.M. | | 1.0 | " | " | " | " | |
| " | 5.00 P.M. | | 1.5 | " | " | " | " | |
| February 8, | 8.30 A.M. | | 1.0 | " | " | " | " | |
| " | 2.30 P.M. | | 0.0 | " | " | " | " | |
| February 9, | 8.30 A.M. | | 3.0 | " | " | " | " | |
| February 10, | 9.30 A.M. | | 2.0 | " | " | " | " | |
| | | —— |
| | | 17.0 |
From these results several interesting conclusions may
be drawn, in conformity with the statements already made.
Thus, as soon as proteolysis commences, the products
formed begin to show their greater affinity for acid by
withdrawing acid from its combination with the native
proteid, a supposition which is necessary to account for
even the starting of the proteolytic process. Further, it is
evident that proteoses and peptones combine with a far
larger equivalent of acid than the native albumin is capable
of; 17 c.c. of 0.2 per cent. HCl being required in the
above experiment to satisfy the greater combining power
of the newly formed products. This doubtless depends
upon the cleavage of the large proteid molecule into a
number of smaller or simpler molecules, each of the latter,
perhaps, combining with a like number of HCl molecules.
This view of the relationship of the individual proteoses
and peptones is one more or less generally held, and is supported
by many facts.106 However this may be, it is evident
that the products of pepsin-proteolysis combine with a
larger amount of hydrochloric acid than the mother-proteid,
and that the transformation of the latter, at least
under the conditions of this experiment, is a slow and
gradual process. In the living stomach, on the other
hand, where the secretion of acid is progressing with ever-increasing
rapidity, it is easy to see that the process of
proteolysis would naturally be much more rapid.
Just here we may recall the theory advanced by Richet107
quite a number of years ago that the acid of the gastric
juice is a conjugate acid, composed of leucin and hydrochloric
acid, a theory which has found little acceptance.
Klemperer,108 however, assumed that solutions of leucin
hydrochloride with pepsin would not digest albumin, but
Salkowski and Kumagawa109 have shown by experiments
that leucin and other amido-acids, as glycocoll, may be dissolved
in hydrochloric acid in such proportion that the
solution is practically composed of leucin hydrochloride,
without interfering with the digestive action of pepsin-acid
on blood-fibrin; the solution being physiologically active,
although Günzburg’s reagent shows an entirely negative
result for free acid. If the matter is studied quantitatively,
however, it will be found that the amido-acids
combining in this manner with the hydrochloric acid of
the gastric juice do give rise to some disturbance of proteolytic
action;110 i. e., digestion may be less rapid, especially
on egg-albumin, a conclusion which Salkowski111 has lately
confirmed. Still, under such circumstances, digestion does
go on and at a fairly rapid rate; hence, if there is a combination
between the acid and these organic bodies, as is
indicated by Günzburg’s reagent, the acid is still active
physiologically, even more so than in the compound formed
by the interaction of proteid and acid. In other words,
many of these neutral organic bodies that may originate in
the stomach through fermentative processes, or otherwise,
and which tend to combine with the acid of the gastric
juice, do not, as a rule, impede pepsin-proteolysis to the
same extent that an excess of proteid matter may. In
fact, in artificial digestions long continued, pepsin-acid
solutions containing considerable leucin, for example, may
accomplish as much in the way of digesting proteid matter
as the same amount of pepsin-acid without leucin; but the
inhibitory action of the amido-acid is there, and may be
shown during the first few hours of the experiment, when
less proteoses and peptones are formed than in the control
experiment without leucin.
It is foreign to our subject to discuss here methods for
the detection of so-called free and combined hydrochloric
acid in the stomach-contents, or the special significance of
such findings in health and disease. I cannot refrain,
however, in connection with what has been said above
concerning the proteolytic action of pepsin in the presence
of combined acid, from saying a word concerning the
usual deductions drawn from the absence of free acid in
the stomach-contents. As Langermann112 has recently
expressed it, we have methods for discriminating between
free and combined acid; we can, moreover, determine the
amount of free acid, but is it not equally important to be
able to say something definite concerning the amount of
combined acid in the stomach-contents? Even in the
absence of free hydrochloric acid there may be a sufficient
amount of HCl secreted to answer all the purposes of
digestion, and yet at no time may there be any free acid
present to be detected by the various color-tests ordinarily
made use of. I am aware that in ordinary examinations of
the stomach-contents after a test meal the results are
essentially comparative, and possibly all that are necessary
for clinical purposes. What I wish to emphasize, however,
is that in order to pass conclusively upon tsufficiency
or insufficiency of the gastric secretion, it is wise
to know not only the total acidity of the stomach contents
and whether there is free acid or not, but to know more
about the amount of combined acid present. Thus, there
is a natural tendency to divide the fluids withdrawn from
the stomach into three groups, viz., those which contain free
acid in moderate amount, those which contain free acid in
excess, and those in which free acid is entirely absent; but
in the latter group, there may be very marked differences
in the amount of acid combined with the proteid and other
material present. It appears to me that one of the questions
to be answered is whether there is sufficient combined
HCl present to meet all the requirements for digestion.
If there is, that gastric juice may be just as normal as the
one containing free mineral acid, and yet, according to our
present tendencies, we should be inclined to call the juice
containing no free acid abnormal, although there may be
sufficient combined acid present to meet all the requirements
for digestion. Hence, in examination of the stomach-contents,
it is well to consider the use of those methods
which tend to throw light upon the amount of combined
acid present, for in my opinion it is only by a determination
of the total amount of combined acid that we can
arrive at a true estimate of the extent of the HCl
deficiency. Obviously, in simple clinical examinations of
the stomach-contents after a test meal, where proteid
matter is not present in large amount, free acid may reasonably
be expected to appear after a definite period; but
in any event, it is well to remember that free hydrochloric
acid is not absolutely indispensable for fairly vigorous proteolytic
action, and that in the presence of moderate
amounts of proteid matter a large quantity of acid is
required to even saturate the albuminous material.
Consider for a moment the amount of acid a given
weight of proteid will combine with, before a reaction for
free acid can be obtained. Thus, Blum113 has stated that
100 grammes of dry fibrin will require 9.1 litres of 0.1 per
cent. hydrochloric acid to completely saturate it. Hence,
with a daily consumption of 100 grammes of proteid, there
would be needed for gastric digestion 4.5 litres of 0.2 per
cent. hydrochloric acid daily, and even this would not
suffice to give any free acid, assuming that none of the
acid is used over again. The results I have already given
for egg-albumin tend to show that 1 gramme of pure
albumin, free from inorganic salts, when dissolved in a
moderate amount of water will combine with about 30 c.c.
of 0.2 per cent. hydrochloric acid. Consequently, on this
basis, 100 grammes of dry egg-albumin will combine with
3 litres of 0.2 per cent. HCl, and not until this amount of
acid has been added to such a mixture will reaction for
free acid be obtained with Günzburg’s reagent. Hence
we can easily see, in view of these figures, that the production
of hydrochloric acid by the gastric glands may at
times be very extensive, without the stomach-contents
necessarily containing free acid.
While I am by no means willing to agree with Bunge114
that the chief importance of the acid of the gastric juice is
its action as an antiseptic, I am decidedly of the opinion
that the lack of free hydrochloric acid in the stomach-contents
is more liable to cause disturbance through the consequent
unchecked development of bacteria than through
lack of proteolytic action, assuming, of course, the presence
of a reasonable amount of combined HCl. The hydrochloric
acid of the gastric juice unquestionably plays a
very important part in checking the growth and development
of many pathogenic bacteria, as well as of less
poisonous organisms, which are taken into the mouth with
the food. On all, or at least on nearly all of these organisms,
hydrochloric acid exerts a far greater destructive
action when free than when combined with proteid matter.
As Cohn115 has plainly shown, both hydrochloric acid and
pepsin-hydrochloric acid quickly hinder acetic- and lactic-acid
fermentation, but when the acid is combined with
peptone, for example, it is no longer able to exercise the
same inhibitory influence. It is also important to note
that the lactic-acid ferment is not so sensitive to hydrochloric
acid as the acetic-acid ferment. Consequently,
when lactic-acid fermentation is once developed a comparatively
large amount of HCl is required to arrest it.
Hence, as we all know, a diminished secretion of hydrochloric
acid renders possible acid fermentation of the
stomach-contents, as well as putrefactive changes which
would not occur in the presence of free HCl, and which
are very incompletely checked when the acid is over-saturated
with proteid matter.
Pepsin-proteolysis, however, may proceed, to some
extent, at least, even though a small amount only of combined
acid is present. The combined acid, however, must
be hydrochloric acid, if proteolysis is to be at all marked.
To be sure, pepsin will act in the presence of lactic acid,
as well as in the presence of other organic acids, and inorganic
acids, likewise, but such action at the best is considerably
weaker than the action of pepsin-hydrochloric acid.116
The ferment pepsin can exert its maximum action only
in the presence of free hydrochloric acid. There must be
sufficient HCl to combine with all of the proteid matter
present, and the products of proteolysis as fast as they are
formed, if digestion is to be rapid and attended with the
formation of a large proportion of the final products of
proteolysis. It is under such conditions that our study of
pepsin-proteolysis is usually conducted. Further, it is to
be remembered that our knowledge of the products of
such proteolytic action depends almost entirely upon data
accumulated by artificial digestive experiments. In no
other way can we be absolutely certain of the conditions
under which the proteolysis is accomplished, for it is a
significant fact, perhaps plainly evident from what has
already been said in the preceding lecture, that the character
of the products resulting from ordinary proteolysis is
dependent in great part upon the attendant circumstances.
Thus, with a relatively small amount of acid, and perhaps
also of pepsin, the initial products of proteolysis are especially
prominent, while with an abundance of both pepsin
and free acid, coupled with long-continued action, the final
products predominate. Between these two extremes there
are many possible variations, as was, I think, made clear in
the previous lecture. At the same time, it is to be noticed
that these differences are mainly differences in the proportion
of the several products, rather than in the nature of
the resultant bodies.
In a general way, the products of pepsin-proteolysis may
be divided into three main groups, viz., bodies precipitated
by neutralization and represented mainly by the
so-called syntonin or acid-albumin; bodies precipitated by
saturation of the neutralized fluid with ammonium sulphate
and represented by proteoses; bodies non-precipitable by
saturation with ammonium sulphate and represented by
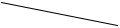
amphopeptones. The relationship of the individual products
may be clearly seen from the following scheme,
arranged after the plan suggested by Neumeister.
| | Native Proteid. | | |
| |  | | |
| | Syntonin. | | |
|  |  | |
| Protoproteose. | | | Heteroproteose. |
 | | | (dysproteose). |
| | |
| Deuteroproteose. | | | Deuteroproteose. |
| | | |
| Peptone. | | | Peptone. |
It is, of course, to be understood that this is not intended
to represent anything more than the order of formation of
the several bodies, no attention being paid here to the hemi-
or anti-character of the several products, or classes of
products. Thus, proto and heteroproteose are primary
bodies formed directly from the initial product syntonin
by the further action of the ferment. In the same sense,
deuteroproteose is a secondary proteose, being formed by
the further hydration of the primary body. Lastly, peptones,
the final products of pepsin-proteolysis, are the result
of the hydration and possible cleavage of deuteroproteoses.
Further, in almost every gastric digestion there is also
formed a small amount of antialbumid, a product insoluble
in dilute hydrochloric acid and which consequently appears
as an insoluble residue. This body is very resistant to the
action of pepsin-acid when once formed, but may be slowly
converted, in part at least, into a soluble antialbumose and
thence into antipeptone.
All of these bodies can be readily identified in any
digestive mixture containing them by a few simple reactions.
Thus, after having removed any acid-albumin or
syntonin present by neutralization, the concentrated fluid
can be tested at once. If primary proteoses are present,
the neutral fluid will yield a more or less heavy precipitate
on addition of crystals of rock-salt, precipitation being complete
only when the fluid is saturated with the salt.
Further, if the proteoses are present in not too small quantity,
nitric acid added drop by drop to the neutralized fluid
will produce a white precipitate, readily soluble on application
of heat but reappearing as the solution cools. If
primary proteoses are wholly wanting, then no precipitate
will be obtained by acid unless the fluid is saturated with
salt, in which case a portion of the deuteroproteose will be
precipitated. The two primary proteoses differ from each
other especially in solubility; protoproteose being readily
soluble in water alone, while heteroproteose is soluble only
in salt solutions, dilute acids, and alkalies. Hence, when
these two bodies are precipitated together by saturation
with salt, they may be readily separated by dissolving them
in a little dilute salt solution, and dialyzing the fluid in running
water until the salt is entirely removed; heteroproteose
will then be precipitated, while the proto-body remains in
solution.
By long contact with water, and even with concentrated
salt solutions, heteroproteose tends to undergo change into
a semi-coagulated form, named dysproteose, insoluble in
dilute sodium-chloride solutions. This body can be reconverted
into heteroproteose, in part at least, by solution in
dilute acid, or alkali, and reprecipitation by neutralization.
As a class, the proteoses are characterized by far readier
solubility in water than native proteids, by a far greater
degree of diffusibility, by non-coagulability by heat and by
alcohol, although precipitable by the latter agent. Further,
nearly all proteose precipitates are exceedingly sensitive
toward heat, tending to dissolve as the fluid is warmed and
reappearing as the solution cools. In fact, this peculiarity
often serves as a means of identification. Potassium ferrocyanide
and acetic acid, picric acid in excess, and likewise
cupric sulphate, all precipitate the primary proteoses, while
deuteroproteose is only slightly affected by these reagents,
or indeed not at all.
In order to separate the secondary proteose from the
primary bodies in the absence of peptones, the fluid is neutralized
as nearly as possible, and then, after suitable concentration,
is saturated with sodium chloride for the partial
precipitation of the primary proteoses. To the clear filtrate,
acetic acid117 is added drop by drop as long as a precipitate
results, the latter being composed of a mixture of protoproteose
and deuteroproteose. That is to say, protoproteoses
are not completely precipitated from neutral solutions by
saturation with salt alone; a little acid is required to complete
it, but this tends to bring down a certain amount of
deuteroproteose. From this filtrate, however, the deutero-body
can be separated in a pure form by dialyzing away
the salt and acid, and then concentrating the fluid and precipitating
with alcohol. When the proteoses are mixed
with peptones, the former must first be separated collectively
by saturation of the fluid with ammonium sulphate.
Peptones are especially characterized by non-precipitation
with the ordinary precipitants for proteid bodies,
and especially by the fact that they are wholly indifferent
to saturation with ammonium sulphate either in neutral,
acid, or alkaline fluids. This reaction, which constitutes
the main, and perhaps the only absolute method of separating
peptones from proteoses must be carried out with great
thoroughness in order to insure a complete precipitation of
deuteroproteose. The latter stands midway between primary
proteoses and peptones in many respects, and seems to
share with peptones something of a tendency to resist precipitation
by the ammonium salt. Indeed, as Kühne118 has
recently pointed out, the last traces of deuteroproteose can
be precipitated from the fluid only by long continued boiling
of the ammonium sulphate-saturated fluid, and even
then it is seldom complete unless the reaction of the fluid
is alternately made neutral, acid, and alkaline, and the heating
continued for some time after each change in reaction.
Under such circumstances, the last portions of deuteroproteose
separate from the salt-saturated fluid and float on the
surface in the form of an oily or gummy mass, while the
true peptone remains in the fluid absolutely non-precipitable
by the salt.
In this filtrate, peptone can be detected by adding to a
small portion of the fluid a very large excess of a strong
solution of potassium hydroxide, followed by the addition
of a few drops of a very dilute solution of cupric sulphate.
If peptone is present a bright red color will appear, the
intensity of which, with the proper amount of cupric sulphate,
will be proportional to the amount of peptone present.
If it is desired to separate the peptone from the
ammonium-sulphate-saturated fluid, there are several
methods available, of which the following is perhaps the
most satisfactory: The fluid is concentrated somewhat,
and set aside in a cool place for crystallization of a
portion of the ammonium salt. The fluid is then mixed
with about one-fifth its volume of alcohol, and allowed to
stand for some time, when it separates into two layers—an
upper one, rich in alcohol, and a lower one, rich in salts.
The latter is again treated with alcohol, by which another
separation of the same order is accomplished. Finally,
the lighter alcoholic layers containing the peptone are
united, and exposed to a low temperature until considerable
of the contained salt crystallizes out. The fluid is
then concentrated, and after addition of a little water is
boiled with barium carbonate until the fluid is entirely
free from ammonium sulphate. Any excess of baryta
in the filtrate is removed by cautious addition of dilute
sulphuric acid, after which the concentrated fluid,
reduced almost to a sirupy mass, is poured into absolute
alcohol for precipitation of the peptone.
So separated, the peptone formed in gastric digestion is
exceedingly gummy, but can be transformed into a yellowish
powder, very hygroscopic, of more or less bitter taste,
and, when thoroughly dry, dissolving in water with a hissing
sound and with considerable development of heat, like
phosphoric anhydride.119
I have introduced these dry chemical facts, none of
which are especially new, because I deem them of considerable
importance and because they are not very generally
known. In fact, there seems to be a tendency on the part
of some who are more or less familiar with the advances
made in our knowledge of the products of pepsin-proteolysis
to question the existence of these different bodies, or to
show at least a spirit of indifference toward these recent
facts which have been gradually accumulated, and I may
say accumulated at the expense of considerable labor. The
time is past for calling the products of gastric digestion
peptones; it is time for a full recognition of the fact that
pepsin-proteolysis is synonymous with the production of a
row of bodies, chemically and physiologically distinct from
each other, each endowed with individuality enough to
admit of certain detection, and all bearing a certain
specific and harmonious relationship to their neighbors, the
other members of the series.
Further, it is not enough to admit the formation of a single
intermediate body, midway between syntonin and peptone.
The so-called propeptone of the past is simply a mixture
of proteoses, of ever changing composition, varying
with each change in the proportion of the component proteoses.
Each of these proteoses can be detected, under
suitable conditions, in the products of every artificial digestion
as well as in the stomach-contents, and no better
measure of the proteolytic power of the natural stomach-secretion
can be devised than a study of the character of
the individual bodies present in the stomach-contents after
a suitable test meal. The proper tests and separations can
be made with a small amount of the filtered fluid, and much
light thrown upon the digestive power of the secretion by
even a rough estimate of the proportion of primary and
secondary proteoses and peptones formed in a given time,
after the ingestion of a certain amount of proteid food.
In pepsin-proteolysis we have to deal, in my opinion,
with a series of progressive hydrolytic changes in which
peptones are the final products of the transformation.
Commencing with the formation of acid-albumin or syntonin,
hydrolysis and cleavage proceed hand in hand, under
the guiding influence of the proteolytic enzyme, and each
onward step in the process is marked by the appearance of
a new body corresponding to the extent of the hydrolysis;
each body, perhaps, being represented by a row or series of
isomers, all externally alike, but different in their inner
structure, according to the proportion of hemi- and anti-groups
contained in the molecule. As opposed to this
theory, we have the older views of Maly,120 Herth,121 Henninger122
and others, based upon observations which tend to
show that peptones do not differ in chemical composition
from the proteids which yield them. As a matter of fact,
the products then analyzed were not peptones at all; they
were merely the primary products of pepsin-proteolysis, i. e.,
what we now term primary proteoses, and it is time we
stopped using such data to enforce the theory that peptones
are polymers of the proteids from which they are derived.
In 1886, the writer, in conjunction with Professor
Kühne, commenced a study of the various cleavage products123
formed by the action of pepsin-hydrochloric acid
from the better characterized and purer proteids, this being
a continuation of our earlier work on the proteoses and
peptones formed from blood-fibrin, serum-albumin, etc.
This work I have continued in my laboratory up to the
present time, with many co-workers, and as a result we
have to-day a series of observations gradually accumulated
during these last seven years, some the results of work carried
on this last year, which speak in no uncertain way of
the character of both the primary and secondary products
of pepsin-proteolysis. Furthermore, in attempting to settle
this question once for all, I have selected for study examples
from the various classes of both animal and vegetable
proteids; and as representatives of the latter have had carried
out two lengthy series of experiments on the crystallized
proteids which occur so abundantly in some seeds, on
the assumption that these crystalline bodies would furnish
a certain guarantee of purity which might naturally be
lacking in the amorphous proteids of animal origin. Some
of these results are now placed together in the following
tables, a study of which reveals some very interesting facts:
COMPOSITION OF PROTEOLYTIC PRODUCTS FORMED BY
PEPSIN-HYDROCHLORIC ACID.
Proteolysis of Blood-fibrin.
| Mother Proteid. | Protofibrinose.124 | Heterofibrinose.124 | Deuterofibrinose.124 | Amphopeptone.125 |
| C | 52.68 | 51.50 | 50.74 | 50.47 | 48.75 |
| H | 6.83 | 6.80 | 6.72 | 6.81 | 7.21 |
| N | 16.91 | 17.13 | 17.14 | 17.20 | 16.26 |
| S | 1.10 | 0.94 | 1.16 | 0.87 | 0.77 |
| O | 22.48 | 23.63 | 24.24 | 24.65 | 27.01 |
Proteolysis of Paraglobulin.126
| Mother Proteid. | Protoglobulose. | Heteroglobulose. | Deuteroglobulose. |
| C | 52.71 | | 51.57 | 52.10 | 51.52 |
| H | 7.01 | | 6.98 | 6.98 | 6.95 |
| N | 15.85 | | 16.09 | 16.08 | 15.94 |
| S | 1.11 |  | 25.36 | 24.84 | 25.59 |
| O | 23.24 |
Proteolysis of Coagulated Egg-albumin.
| Mother Proteid. | Protoalbumose.127 | Heteroalbumose.127 | Deuteroalbumose.127 | Hemipeptone.128 |
| C | 52.33 | 51.44 | 52.06 | 51.19 | 49.38 |
| H | 6.98 | 7.10 | 6.95 | 6.94 | 6.81 |
| N | 15.84 | 16.18 | 15.55 | 15.77 | 15.07 |
| S | 1.81 | 2.00 | 1.63 | 2.02 | 1.10 |
| O | 23.04 | 23.28 | 23.81 | 24.08 | 27.64 |
Proteolysis of Casein from Milk.
| Mother Proteid. | Protocaseose.129 | Heterocaseose.130 | α Deuterocaseose.129 | β Deuterocaseose.129 |
| C | 53.30 | | 54.58 | 53.88 | 52.10 | 47.72 |
| H | 7.07 | | 7.10 | 7.27 | 6.93 | 6.73 |
| N | 15.91 | | 15.80 | 15.67 | 15.51 | 15.97 |
| S | 0.82 | | 22.52 | 23.18 | 25.46 | 29.58 |
| O | 22.03 |
Proteolysis of Myosin from Muscle.131
| Mother Proteid. | Protomyosinose. | Deuteromyosinose. |
| C | 52.82 | 52.43 | 50.97 |
| H | 7.11 | 7.17 | 7.42 |
| N | 16.77 | 16.92 | 17.00 |
| S | 1.27 | 1.32 | 1.22 |
| O | 21.90 | 22.16 | 23.39 |
Proteolysis of Elastin.132
| Mother Proteid. | Protoelastose. | Deuteroelastose. |
| C | | 54.24 | 54.52 | 53.11 |
| H | | 7.27 | 7.01 | 7.08 |
| N | | 16.70 | 16.96 | 16.85 |
| S | | 21.79 | 21.51 | 22.96 |
| O |
Proteolysis of Gelatin.133
| Mother Proteid. | Protogelatose. | Deuterogelatose. |
| C | 49.38 | 49.98 | 49.23 |
| H | 6.81 | 6.78 | 6.84 |
| N | 17.97 | 17.86 | 17.40 |
| S | 0.71 | 0.52 | 0.51 |
| O | 25.13 | 24.86 | 26.02 |
Proteolysis of Phytovitellin134 (Crystallized) from Squash Seed.
| Mother Proteid. | Protovitellose. | Deuterovitellose. |
| C | 51.60 | | 51.52 | 49.27 |
| H | 6.97 | | 6.98 | 6.70 |
| N | 18.80 | | 18.67 | 18.78 |
| S | 1.01 | | 22.83 | 25.25 |
| O | 21.62 |
Proteolysis of Phytovitellin135 (Crystallized) from Hemp Seed.
| Mother Proteid. | Protovitellose. | Deuterovitellose. | Peptone. |
| C | 51.63 | 51.55 | 49.78 | 49.40 |
| H | 6.90 | 6.73 | 6.73 | 6.77 |
| N | 18.78 | 18.90 | 17.97 | 18.40 |
| S | 0.90 | 1.09 | 1.08 | 0.49 |
| O | 21.79 | 21.73 | 24.44 | 24.94 |
Proteolysis of Glutenin136 from Wheat.
| Mother Proteid. | Protoglutenose. | Heteroglutenose. | Deuteroglutenose. |
| C | 52.34 | 51.42 | 51.82 | 49.85 |
| H | 6.83 | 6.70 | 6.79 | 6.69 |
| N | 17.49 | 17.56 | 17.43 | 17.57 |
| S | 1.08 | 1.34 | 1.59 | 0.80 |
| O | 22.26 | 22.98 | 22.37 | 25.09 |
Proteolysis of Zein.137
| Mother Proteid. | Protozeose. | Deuterozeose. |
| C | 55.23 | 53.29 | 51.31 |
| H | 7.26 | 6.87 | 6.88 |
| N | 16.13 | 16.10 | 16.27 |
| S | 0.60 | 1.54 | 1.08 |
| O | 20.78 | 22.20 | 24.46 |
In considering these results, it is to be noticed that there
is a general unanimity of agreement except in the case of
the albuminoid gelatin. In the proteolysis of this body,
for some reason not explainable, the digestive products
show no marked deviation from the composition of the
mother-proteid, but in every other instance there is to be
traced a distinct tendency toward diminution in the content
of carbon, proportional to the extent of proteolysis.
In the primary bodies, proto and heteroproteoses, the percentage
of carbon is only slightly lowered; indeed, in
some few cases, notably in elastin and casein, the primary
products show a slight increase in their content of carbon,
but in most instances there is a slight falling off in the
percentage of this element. In the deuteroproteoses, however,
the loss of carbon is very marked. The percentage
loss, to be sure, varies with the different proteids, doubtless
dependent in part upon the nature of the proteid itself,
and also, I think, upon the strength of the proteolytic
agent employed and the duration of the proteolysis. It is
to be further noticed that peptones, whenever analyzed,
show a still further loss of carbon and also a marked loss
of sulphur. In nitrogen there is no constant difference.
On the assumption that these various products of proteolysis
are formed by a series of hydrolytic changes,
accompanied by cleavage of the molecule, we might at first
glance look for a marked increase in the content of hydrogen.
But when we consider the size of the proteid molecule,
with the small proportion of hydrogen contained
therein and the large amount of carbon, it is plain that
hydrolytic cleavage might naturally leave its mark on the
percentage of carbon, rather than on the percentage of
hydrogen of the resultant products. In view of these facts,
the above results show nothing inconsistent with the theory
that pepsin-proteolysis, as a rule, is accompanied by a series
of progressive hydrolytic cleavages in which the primary
proteoses are the result of a slight hydration, these bodies
by continued proteolysis being further hydrated with
formation of secondary proteoses, which in turn undergo
final hydration and cleavage into true peptones. In accord
with this theory, true peptones always show a marked difference
in composition from that of the mother-proteid,
the most striking feature being the greatly diminished content
of carbon, which may be taken as a measure, in part
at least, of the extent of the hydrolytic change. And it is
to be noticed that the crystallized phytovitellins are no
exception to the general rule; the secondary vitelloses and
peptones resulting from proteolysis bear essentially the
same relationship to the mother-proteids that the albumoses
from egg-albumin do. Moreover, the alcohol-soluble proteids,
of which the zein of cornmeal is a good example,
show the same general tendency, and it is an interesting
fact that the proteoses, or more specifically the zeoses,
formed from this peculiar proteid, are readily soluble in
water and show the general proteose reactions. It may
also be mentioned that these zeoses, as well as the elastoses,
are very resistant to further hydrolysis by pepsin-acid, and
yield only comparatively small amounts of true peptones.
In connection with this question of the composition of
proteoses and peptones as formed by pepsin-proteolysis, it
is interesting to note a recent observation recorded by
Schützenberger.138 This experimenter took 350 grammes
of moist blood-fibrin, corresponding to 75.5 grammes of
dry substance, and subjected it to proteolysis with 2.5 litres
of a very strong pepsin-hydrochloric acid solution for five
days. The resultant fluid was then freed from acid by
treatment with silver oxide, after which the solution was
evaporated to dryness on a water-bath and the residue dried
in vacuo. This residue, termed by Schützenberger fibrin-peptone,
was found on analysis to contain 49.18 per cent.
of carbon, 7.09 per cent. of hydrogen, and 16.33 per cent.
of nitrogen, thus agreeing very closely with true fibrin-peptone
as analyzed by Kühne and myself. Further,
Schützenberger showed that the fibrin in undergoing this
transformation had taken on 3.97 per cent. of water. But
to my mind, the most significant fact connected with this
experiment is the positive evidence it affords, not only of
hydration as a feature of peptonization by pepsin-acid, but
that this greatly diminished content of carbon, so characteristic
of peptones, and to a less extent of deuteroproteoses,
is wholly independent of the methods of separation and
purification ordinarily made use of. Thus, Schützenberger,
in the above experiment, did not attempt any separation of
individual bodies. Proteolysis was carried out under conditions
favoring maximum conversion into peptone, and
the resultant product, or products, was analyzed directly
without recourse to any methods of precipitation or purification.
To be sure, the substance analyzed could not
have been peptone entirely free from proteose, but in any
event it represented the terminal products of pepsin-proteolysis,
and like true amphopeptone contained 3.5 per
cent. less carbon than the original fibrin. Hence, we may
conclude, without further argument, that peptonization in
gastric digestion is the result of distinct hydrolytic action,
in which the original proteid molecule is gradually broken
down, or split apart, into a number of simpler molecules,
the proteoses and peptones.
Peptones, i. e., amphopeptones, are the final products of
gastric digestion; but to how great an extent is actual
peptonization carried on in pepsin-proteolysis? As we
have seen, syntonin, primary proteoses, secondary proteoses,
and peptones are all products of pepsin-digestion, and
it might perhaps be assumed that ultimately all of a given
proteid undergoing pepsin-proteolysis would be converted
into amphopeptone. Examination, however, shows that
such is not the case, at least in artificial digestive experiments.
Peptones are truly formed, and many times in
large amount, but never under any circumstances have I
been able to effect a complete transformation of any proteid
into true peptone by pepsin-proteolysis; there is
always found a certain amount of proteoses more or less
resistant to the further action of the ferment. Obviously,
the nature and proportion of the individual products
formed in any digestive experiment are dependent greatly
upon the attendant conditions; but even with a large
amount of active ferment, an abundance of free hydrochloric
acid, a proper temperature, and a long-continued
period of digestion, even five and six days, there is never
found a complete conversion into peptone. Indeed, the
largest yield of peptone I have ever obtained in an artificial
digestion is sixty per cent., while the average of a large
number of results under most favorable circumstances is
somewhat less than fifty per cent.139
We understand that peptones are the products of the
hydration and cleavage of previously formed proteoses.
The primary proteoses pass into secondary proteoses and
these into peptones, but for some reason this transformation
after a time becomes a slow and gradual process. At
first there is a marked and rapid progression; the proteid
undergoing proteolysis is rapidly dissolved, and both proteoses
and peptones may be detected in abundance. But if
we continue to watch the changing relations of primary
and secondary proteoses and peptones, we find that progression
soon ceases to be rapid, and eventually travels
onward at a snail’s pace. Thus, in one experiment with
coagulated egg-albumin, there was found at the end of
forty-eight hours’ digestion with pepsin-hydrochloric acid,
only thirty-seven per cent. of peptones with fifty-eight per
cent. of proteoses, and yet digestion had been sufficiently
vigorous to allow of a complete solution of the proteid in
two hours. At the end of seventy-two hours the amount
of peptones had increased to about forty-two per cent., the
proteoses having correspondingly diminished; but even at
the end of seventeen days only fifty-four per cent. of peptones
were to be found, thus affording striking evidence of
the slow conversion of the first-formed products into peptones.
Naturally, the individual proteoses show marked differences
in their rate of conversion into secondary or final
products. Take as an illustration some results140 obtained
with caseoses formed in the digestion of the casein of milk.
Thus, heterocaseose, a primary product, yielded only fifteen
per cent. of peptone after ninety-four hours at 40° C. with a
strong pepsin-acid solution. Protocaseose, however, containing
some deuterocaseose, under like conditions, yielded
thirty-two per cent. of peptone in one hundred and nineteen
hours, while pure deuterocaseose gave sixty-six per
cent. of peptone in one hundred and thirty-seven hours.
Evidently, then, the first-formed soluble products of gastric
digestion, i. e., the primary proteoses, are only slowly converted
into peptone, since they must first pass through the
intermediate stage of deuteroproteose, which is plainly not
a rapid process. The deutero-body, on the other hand,
once formed is more rapidly converted into peptone, but
even this is in no sense a rapid process. Hence, in the
artificial digestion of proteids with pepsin-hydrochloric
acid, solubility of the proteids may be quite rapid, and
even complete in a very short time, but the resultant products
will be mainly proteoses and not peptones. The
latter are truly formed and in considerable amount, but
proteoses, either as primary or secondary bodies, are invariably
present and usually in excess of the peptones.
In this connection the question naturally arises how far
we are to trust these results in their bearing on the natural
process of digestion as it occurs in the living stomach.
Obviously, the conditions are quite different in the two
cases. In artificial digestions, we have especially the
influence of an ever-increasing percentage of soluble products
on the activity of the ferment, a condition of things
generally considered as more or less inhibitory to enzyme
action. We have attempted to measure the real value of
this influence by experiments141 conducted in parchment
dialyzing tubes, in which the conditions are made favorable
for the removal of at least some of the products of digestion
as fast as they are formed. In these experiments, the
dialyzer tubes containing the proteid and pepsin-acid were
immersed in a large volume of 0.2 per cent. hydrochloric
acid (about three litres), which was gradually changed from
time to time, the whole mixture being kept at 40° C. during
the entire period of the experiment. The extent of
peptonization was then ascertained by analysis of both the
contents of the dialyzer tubes and of the surrounding acid,
the results being compared with those obtained from control
experiments carried on in flasks. Without considering
the results in detail, it may be mentioned that the slow
and incomplete peptonization so characteristic of artificial
gastric digestion is not materially modified by this closer
approach to the natural process. The several digestions
carried on in the dialyzer tubes were certainly accompanied
by a fairly rapid withdrawal of the diffusible products of
digestion, yet no noticeable increase in the amount of peptone
formed was observed. The results certainly favor
the view that the conversion of the primary products of
gastric digestion into true peptone is a slow and gradual
process, even under the most favorable circumstances, and
that this lack of complete peptonization is not due to
accumulation of the products of digestion, but is rather an
inherent quality of pepsin-proteolysis under all circumstances.
In these dialyzer experiments it was observed that not
only did peptones diffuse, but also the proteoses. In fact,
it was found that six to eight per cent. of the proteoses
formed passed through the parchment walls of the dialyzer
tubes into the surrounding acid in the nine hours’ digestion.
This led to a study of the diffusibility of proteoses
in general, from which we were led to conclude that these
bodies possess this power to a greater degree than had
hitherto been supposed. As might be expected, it was
also found that the attendant conditions modify materially
the rate of diffusibility; the two factors especially prominent
being temperature and the volume of the surrounding
fluid. Thus, 1.9 grammes of protoalbumose dissolved in
200 c.c. of water and suspended in 4.5 litres of water
heated to 38° C., diffused through the parchment tube to
the-extent of 5.09 per cent., while at 10° C. diffusion
amounted to only 2.57 per cent. Under somewhat similar
conditions, pure peptone diffused to the extent of eleven
per cent. in six hours at 38° C. Somewhat singular, however,
was the result obtained with deuteroalbumose; this
proteose showing a diffusibility considerably less than that
of the proto-body. But as Kühne142 has independently
obtained essentially the same results, this apparent anomaly
cannot depend upon any errors of work.
It is of course to be understood that diffusion experiments
made with dead parchment membranes cannot
necessarily be expected to throw much light upon the rate
of absorption of these bodies through the living membranes
of the stomach and intestine, where, as Waymouth Reid143
has well said, we have to deal with an absorptive force
dependent, no doubt, upon protoplasmic activity, and comparable,
in part at least, to the excretive force of a gland-cell.
Furthermore, in considering absorption as it occurs
in the living stomach, we must necessarily give due weight
to the selective power of the epithelial cells, a power which
may be far more potent even than we suppose. Hence,
without attempting at this point to draw any broad deductions
from our experiments we may simply lay stress upon
the facts themselves, viz., that the primary products of
pepsin-proteolysis are diffusible, and, like true peptones,
are capable of passing through animal and vegetable membranes,
although to a less extent. We may further emphasize
the fact that experiments of this character on diffusibility
can, at the most, only indicate general tendencies, since
every variation in the attendant conditions will exercise
some influence upon the final result.
With reference to the bearing digestive experiments
made in dialyzer tubes have upon the natural process as
carried on in the living stomach, we must necessarily grant
that the conditions approximate only in the crudest way to
those existent in the alimentary tract. At the same time,
if complete peptonization is characteristic of pepsin-proteolysis
in the stomach, and failure to obtain such results in
an artificial digestion is due to lack of withdrawal of the
diffusible products formed, then certainly the experiments
carried on in dialyzer tubes, with abundant opportunity for
diffusion, and with a large excess of free hydrochloric acid,
should show some indications of increased peptone-formation.
But none were obtained.
It is more than probable that the rate of absorption of
diffusible products from the stomach has been overestimated.
Lea,144 for example, assumes that, “normally the
products of digestion, whether proteid or carbohydrate,
are never met with in either the stomach or intestine
in other than the smallest amounts, frequently to be
described as merely traces.” This certainly implies a far
more rapid absorption of proteoses and peptones from the
stomach than results seem to justify. Indeed, recent facts
obtained by Brandl,145 working under Tappeiner’s direction,
tend to show that absorption from the stomach is, under
some circumstances at least, comparatively slow. Brandl’s
experiments were conducted on large and vigorous dogs
with gastric fistulæ, the stomach being shut off from the
intestine by the simple introduction of a small rubber
balloon into the pylorus, which when dilated completely
closed the orifice. By carefully conducted experiments, it
was shown that pure peptone, entirely free from proteose,
is absorbed from the empty stomach in proportion to the
concentration of the peptone solution. Thus, 7.5 grammes
of peptone dissolved in water in such proportion as to
make a five per cent. solution, and allowed to remain in
the stomach for two hours, lost by absorption only 0.28
gramme, equal to 2.68 per cent. of the peptone introduced.
Under similar conditions, a ten per cent. aqueous solution
of peptone lost only 4.5 per cent. by absorption. On the
other hand, when peptone was introduced in larger quantity,
viz., in a twenty per cent. solution, absorption
amounted to thirteen per cent. in two hours.
It is thus evident that pure peptones, even when taken
into the stomach in fairly large amounts, and under conditions
very favorable for rapid absorption, pass into the
circulating blood very slowly. Obviously, however, one
must not lose sight of the fact that when digestion is under
way and the volume of blood consequently increased, there
may be a corresponding rise in the rate of absorption.
There is perhaps a hint of this conclusion in the influence
of alcohol on the absorption of peptone as brought out by
some of Brandl’s experiments. Thus, it was found that
when alcohol was added in considerable quantity to a ten
per cent. solution of peptone, the stomach-mucosa was
greatly reddened, while in two hours the absorption of
peptone amounted to 11.8 per cent. But in any event,
these results certainly do not favor the view that the products
of gastric digestion are absorbed as soon as they are
formed. It is, no doubt, quite different in the intestine,
but in the stomach, where pepsin-proteolysis occurs, we
have, I think, no grounds for assuming that either peptones
or proteoses are rapidly absorbed. Hence, it might
perhaps be considered that the results of pepsin-proteolysis
in the living stomach are much the same as those obtained
in artificial digestion experiments.
Still, there are other differences between natural digestion
and artificial proteolysis than those connected with the
possible absorption of the more diffusible products of
digestion. Thus, in the living stomach there is an ever-increasing
secretion of hydrochloric acid, and perhaps also
of pepsin, more or less proportional to the extent of proteolysis.
On this point Brandl’s experiments again give us
some light. Thus, it was found that the introduction of
an aqueous solution of peptone into the empty stomach led
to the secretion of an acid fluid containing on an average
0.24 per cent. HCl, while, under similar conditions,
the introduction of sugar or potassium iodide was followed
by the secretion of a fluid containing on an average only
0.13 per cent. HCl. Further, the absolute amount of acid
found after the introduction of peptone was far greater
than when sugar or iodide was introduced, since peptone
led to an increase of at least fifty per cent. in the volume
of fluid secreted. Hence, proteolysis in the living stomach
may give rise to such an increased production and secretion
of hydrochloric acid that formation of the terminal
products of gastric digestion may be greatly accelerated.
That such in fact is the case, I have no manner of doubt,
but that it may result in the complete conversion of the
so-called primary and secondary proteoses into peptone I
very much question. In fact, such examinations as I
have made of the stomach-contents after a suitable test-meal
have always resulted in the finding of a relatively
large amount of proteoses. To be sure, true peptone may
be detected and in fairly large amounts, but whenever a
quantitative determination of the relative proportion of the
two has been made, the proteoses have always been in
excess. I have already reported elsewhere the results of
some experiments in this direction made on a healthy
young man, where the stomach-contents were withdrawn
at varying periods after the ingestion of weighed amounts
of coagulated egg-albumin. Thus, in one experiment146 the
stomach was thoroughly rinsed with water, after which 138
grammes of finely divided coagulated-albumin, equal to 16
grammes of dry albumin, were ingested. Three-quarters
of an hour thereafter, the stomach-contents were withdrawn
by lavage and analyzed. As a result, 1.41 grammes
of albumoses were separated and weighed, and 0.84 gramme
of peptones, the relative proportion being expressed by
sixty-two per cent. of albumoses and thirty-seven per cent.
of peptones, calculated on the 2.25 grammes of soluble products
recovered. This expresses the general character of
the results obtained in experiments of this nature, and in
my opinion adds emphasis to the statement already made,
that complete peptonization is not a feature of pepsin-proteolysis,
either in the artificial or in the natural process
as it takes place in the living stomach.
Gastric digestion is to be considered rather as a preliminary
step in proteolysis, preparatory to the more profound
changes characteristic of pancreatic digestion, in which the
ferment trypsin is the important factor. We can thus see
how, as in the case of Czerny’s dogs, an animal may be perfectly
nourished without a stomach, digestive proteolysis
being carried on solely by the pancreatic fluid. You will
remember that two of the dogs operated on by Czerny and
his pupils lived between four and five years after the
operation, with the stomach completely removed, and yet
during this period they were well nourished and ate all
varieties of food with apparently a normal appetite.147
Evidently, then, in some cases at least, digestive proteolysis
can be carried on without this preliminary action of
the gastric juice. Ogata148 arrived at essentially the same
conclusion by the establishment of a duodenal fistula, shutting
off the stomach from the intestine by means of a small
rubber ball which could be inflated with water. On then
introducing coagulated egg-albumin and other forms of
proteid matter into the duodenum, he found that digestion
was at least sufficiently complete to satisfy all the demands
of the system. The only unsatisfactory result was with
collagenous foods, which plainly showed the need of a preliminary
acid digestion. More recently still, Cawallo and
Pachon,149 working in Richet’s laboratory, have studied the
digestibility of different kinds of proteid foods in a dog,
upon which they had performed a gastrectomy; the
entire fundus, as well as the pyloric portion, of the stomach
having been removed. In an animal so operated upon,
after recovery was complete, solid food, as meat, was completely
digested when taken in small quantities at a time.
Raw meat, however, was less completely utilized, the fæces
showing portions of undigested fibres. Still, it was
apparent that intestinal digestion alone was capable of
accomplishing all that was necessary for the complete
nourishment of the animal, when it had once become
accustomed to the changed condition of its alimentary
tract.
These facts are cited not to belittle the importance of
gastric digestion in the nutrition of the body, but rather to
emphasize the probability that pepsin-proteolysis is simply
a preliminary step in digestion; that its function is not in
the direction of a complete peptonization of the proteid
foods ingested, but that its action is especially directed to
the production of soluble products, proteoses, which can be
further digested in the small intestine, or perhaps directly
absorbed after they have passed through the pylorus, or
even from the stomach itself to a certain extent.
It is very evident from what has been said that all forms
of proteid matter, i.e., all the members of the three main
groups spoken of in our classification of the proteids,
excepting only nuclein, reticulin, and the keratins, are
capable of undergoing proteolysis with pepsin-hydrochloric
acid. Further, in every case the main products of the
transformation are proteoses; viz., albumoses, caseoses,
gelatoses, vitelloses, myosinoses, etc., according to the
nature of the proteid undergoing proteolysis; true peptones
being formed in less abundance. Corresponding to
each of these groups are primary and secondary proteoses,
all possessed of many points in common, both chemical
and physiological, yet differing from each other in many
minor respects. These are the important products of
gastric digestion, of pepsin-proteolysis, and it may be well
to consider for a moment some of the physiological properties
of the proteoses and of peptones as well, in order that
we may the better comprehend the general nature of these
substances with reference to their possible action in the
economy.
As far back as 1880, Schmidt-Mülheim150 discovered that
the injection of aqueous solutions of peptone into the
blood-vessels of living dogs was attended by a series of
remarkable phenomena. Thus, the animal passed at once
into a condition of narcosis resembling that produced by
chloroform, accompanied by a fall of general blood-pressure
so great that the animal was liable to die, as from
asphyxia. Further, there was evidence of some marked
change in the condition of the blood, as indicated by loss
of the power of spontaneous coagulation, while the peptone
itself evidently underwent some alteration, or else was
rapidly eliminated, since it could not be detected in the
blood a short time after its introduction. These experiments,
however, were not conducted with true peptone
but with Witte’s “peptonum siccum,” which at that time,
at least, was composed in great part of proteoses. The
general character of these interesting results was confirmed
by Fano,151 who found that the injection of so-called peptone
in the proportion of 0.3 gramme per kilo. of body-weight
was sufficient to bring about complete narcosis,
together with loss of coagulability on the part of the blood.
Very suggestive, however, was the fact that Fano, on trying
similar experiments with the peptone formed by pancreatic
digestion, viz., with antipeptone, which presumably
contained a far smaller proportion of proteoses, failed to
obtain like results; the tryptone, so-called, being exceedingly
irregular in its action, in many cases producing no
effect whatever.
The discovery at this date of the several albumoses, and
their presence in large amounts in all so-called peptones,
led to a study of their physiological action with special
reference to the observations of Schmidt-Mülheim and
Fano. Politzer,152 working under Kühne’s guidance, was
the first to experiment in this direction, and his results are
full of interest as throwing light on the action of the
individual albumoses. Thus proto, hetero, and deuteroalbumose
are all active physiologically, giving rise when
injected into the veins of dogs and cats to strong narcotic
action, varying somewhat in intensity in different individuals.
There is also produced a marked fall in blood-pressure,
due apparently to vaso-motor paralysis, the action
being manifested chiefly, if not wholly, on the splanchnic
region. Thus, after an injection of one of these albumoses,
the mesenteric vessels are always strongly congested,
accompanied frequently by the appearance of a bloody
serum in the peritoneal cavity. Narcotic action is manifested
only so long as the blood-pressure remains sub-normal,
and is due presumably to this marked accumulation of
blood in the large abdominal veins, thus leading to anæmia
of the brain. Albumoses and peptones injected into the
jugular vein likewise produce fever, presumably through
some action on the nervous system by which the equilibrium
of tissue-metamorphosis is interfered with.153
Further, Politzer found that all of the albumoses either
delayed or prevented altogether the coagulation of the
blood, in conformity with the observations of Schmidt-Mülheim
and Fano. In all of these actions the primary
albumoses appeared most effective, deuteroalbumose least
so. Heteroalbumose, however, was constantly most active,
especially in delaying the coagulation of the blood. With
amphopeptone, there was far less narcosis and less diminution
of blood-pressure, while the effect on the coagulability
of the blood was more or less variable, frequently being
entirely negative. Antipeptone, on the other hand, was
found almost wholly wanting in any constant effects,
although in one instance deep narcosis was produced.
Thus, from Politzer’s experiments, it was made clear that
the albumoses, when introduced directly into the blood-current,
possess a far greater toxic action than either
amphopeptone or antipeptone. Albumoses, in sufficiently
large doses, were invariably fatal, while peptones never
produced fatal results so long as the kidneys of the animal
remained intact. The extreme solubility and diffusibility
of peptones, coupled perhaps with their marked diuretic
action, lead to rapid elimination through the kidneys, and
their consequent removal from the system.
Many of these observations made with the albumoses I
have repeated with several of the proteoses and peptones
more recently studied, as protocaseose, protoelastose, the
globuloses, and others. The results may be taken as practically
confirmatory of the older observations, and I make
mention of them in this general way simply to emphasize
the fact that all of the proteoses, though perhaps showing
individual peculiarities, are possessed of marked physiological
properties, which plainly testify to their toxic nature,
when introduced directly into the blood-current.
Young animals are particularly sensitive to the injection
of proteoses into the blood, even when the introduction
takes place very gradually.154 Thus, a young, healthy dog
of 2 kilos. body-weight, eight weeks old, died in one hour
after the injection into the jugular vein of 1 gramme of
protoalbumose in 20 c.c. of water, thus affording a good
illustration of the extreme toxicity of this albumose when
introduced directly into the blood.
Of greater interest, physiologically, are the changes the
individual proteoses undergo after their injection into the
blood. As already stated, peptone so injected may appear
in the urine wholly unaltered. Thus, Neumeister155 has
made injections of both amphopeptone and antipeptone in
the case of dogs, and was able to detect the peptone very
quickly in the urine. I have made like experiments with
other forms of peptone and obtained similar results; thus,
a pure amphopeptone formed from casein by pepsin-proteolysis
(2 grammes in 15 c.c. water) was injected into the
jugular vein of a dog weighing 5 kilos. The urine collected
during several hours after the injection was heated
to boiling, and saturated while hot with ammonium
sulphate. The filtrate, on being tested with cupric sulphate
and potassium hydroxide, gave a fairly strong biuret
reaction for peptone. Another similar experiment made
with antipeptone, formed from the myosin of muscle-tissue,
gave like results.
With proteoses, however, different results are obtained,
as Neumeister156 first pointed out. These bodies introduced
into the blood undergo more or less of a change prior to
their excretion in the urine, the change partaking of the
character of a hydrolytic cleavage in which the primary
proteoses are transformed into secondary proteoses, while
deuteroproteoses are changed into peptones. This is not
necessarily to be interpreted as meaning that the full
equivalent of the proteose injected appears in the urine,
but that the portion which is eliminated through the kidneys
tends to undergo a transformation somewhere en
route, akin to the change produced in pepsin-proteolysis.
As to how common or complete this transformation is
under the above circumstances, we have no positive knowledge.
Such a hydrolytic change certainly occurs in the
case of the dog, and the experimental evidence is in favor
of the view that the transformation is effected in the kidneys
by the pepsin secreted through the urinary tubules,
where there is momentarily a formation of free acid. In
the rabbit, on the other hand, no such change occurs; the
urine from this animal contains practically no pepsin, and
consequently the proteoses eliminated through the kidneys
are excreted unaltered. As, however, the experiments of
Stadelmann157 and others have shown that the urine of all
carnivora, and of man as well, contains a ferment which,
on the addition of a suitable amount of hydrochloric acid,
will digest fibrin with formation of the ordinary products
of pepsin-proteolysis, it is to be presumed that all proteoses
passing through the kidneys will undergo at least some
change prior to their excretion in the urine.
However this may be, it is very evident that the proteoses
formed in gastric digestion cannot be absorbed as
such directly into the blood-current. Introduced into the
blood, they behave in such a manner as to warrant the conclusion
that they are truly foreign substances, and the system
makes a brave endeavor to remove them as speedily as
possible. The same may be said of amphopeptones, from
which we may conclude that all of these products of pepsin-proteolysis
undergo some transformation during the
process of absorption, by which their toxicity is destroyed
and their nutritive qualities rendered fully available for
the needs of the body. Discussion of this question, however,
will be left until the next lecture.
In view of these pronounced physiological properties of
the proteoses, it is interesting to recall the now well-known
fact that many of the chemical poisons produced by bacteria
are proteose-like bodies, chemically, at least, closely akin
to the proteoses resulting from pepsin-proteolysis. Thus,
Wooldridge158 as early as 1888 pointed out that an alkaline
solution of tissue-fibrinogen exposed to the action of
anthrax-bacilli suffered some change, so that when introduced
into the blood it possessed the power of producing
immunity to anthrax. This observation was verified by
Hankin,159 who further showed that the substance formed
by the anthrax-bacilli was a veritable albumose, and that it
truly possessed the power of producing immunity. Sidney
Martin160 carried the matter still further, and by growing the
anthrax-bacilli in a pure solution of alkali-albuminate prepared
from blood-serum, proved the formation of both
primary and secondary albumoses, as well as of peptone,
leucin, tyrosin, and a peculiar alkaloidal substance of pronounced
toxic properties. Martin finds that the albumoses
are not as poisonous as the alkaloid, and surmises that the
alkaloid is contained in the albumose molecule in the
nascent state; further, he suggests that the albumoses in
small doses may exert some protective influence, while in
larger doses they act as vigorous poisons. How true this
may be I cannot say, but my own experience convinces me
that the anthrax-bacilli grown in a culture medium composed
of alkali-albuminate, prepared from egg-albumin, to
which the necessary inorganic salts and some glycerin have
been added, do give rise to albumoses and peptones which
are truly endowed with toxic properties.
Albumose-like bodies have also been obtained by Brieger
and Fränkel161 with the bacillus of diphtheria. These, too,
were endowed with powerful poisonous properties, and
when introduced into the tissues of the body gave rise to
reactions resembling those produced by the Löffler bacillus.
In my own laboratory, recent experiments made with the
bacillus of glanders have shown that when grown in a
slightly acid medium containing alkali-albuminate, albumoses,
peptones, and crystalline bodies such as leucin and tyrosin
are formed in considerable quantities. Kresling162 has
reported similar results. With the tubercle-bacilli, many
like results have been recorded. Thus, among others,
Crookshank and Herroun163 have reported the finding of
albumoses, peptone, and a ptomaine when the bacilli have
been grown in glycerin agar-agar, and also in fluid media.
Koch164 has made a special study of the albumose which
he considers as the specific toxic agent of the so-called
tuberculin. This albumose was found by Brieger and
Proskauer165 to have a somewhat peculiar composition, inasmuch
as it contains forty-seven to forty-eight per cent. of
carbon and only 14.73 per cent. of nitrogen, agreeing,
however, in this respect very closely with the peptone
formed from egg-albumin by the action of bromelin.166 Still
more recently, Kühne167 has made a thorough study of this
albumose, as well as of the other products elaborated by the
growth of the tubercle-bacillus. He designates all of the
peculiar albumoses formed by these bacilli as acrooalbumoses.
They are endowed with marked chemical and
physiological properties, causing a rise of temperature
when injected into the blood, as well as other phenomena
more or less pronounced. It is thus evident there is ample
ground for the statement that all nutritive media in which
pathogenic bacteria have been planted are liable to contain,
sooner or later, toxic substances, many of which at least are
closely related to, if not identical with, the albumoses. It
is not my purpose, however, to consider these points in
detail, nor to quote the many results obtained by other
workers in this direction.
I wish merely to call attention to the fact that the proteoses,
and likewise the peptones formed by pepsin-proteolysis,
are more or less toxic when introduced directly into
the blood, and that they share this property with the proteoses
formed by bacterial organisms, or by the enzymes which
they give rise to. In other words, these primary cleavage
or alteration products of the proteid molecule, however
produced, are more or less poisonous, and if introduced
into the blood-current without undergoing previous change
may show marked physiological action. It is, of course, not
to be understood that these bodies are all alike. They are
surely closely related and possess many points in common,
especially so far as their chemical properties are concerned,
but their chemical constitution and their physiological
action must vary more or less with their mode of origin.
In any event, it is very evident that the proteoses and
peptones formed in the alimentary tract by pepsin-proteolysis
must undergo some transformation, before reaching
the blood-current, by which their peculiar physiological
properties are modified. This modification may be associated
with a conversion into the serum-albumin, or globulin
of the blood. However this may be, the fact remains
that these proteoses formed so abundantly during digestion
can be absorbed and serve as nutriment for the animal
body, but between their formation as a result of proteolysis
and their passage into the blood they are exposed to some
agency, or agencies, doubtless in the very act of absorption,
by which a further transformation is accomplished. With
this point we shall be able to deal more in detail in the
next lecture.