After considerable experimentation as to a suitable culture medium
for the bacteriological study of sour hams, a modification of the “egg-meat
mixture” used by Rettger[2] in his studies on putrefaction was
found to be the most satisfactory. This medium, which consists of
chopped meat and egg albumen, furnishes an excellent medium for
the growth of putrefactive organisms which rapidly break down the
proteids of the meat, giving rise to the characteristic odors of putrid
decomposition. Rettger used chopped beef and egg albumen, but for
the present work chopped pork was substituted for the beef, as affording
a more suitable medium for the growth of organisms accustomed
to growth in pork hams. The modified medium is prepared as follows:
A. One-half pound of lean pork, freed from excess of fat and
sinew, is finely chopped in a meat chopper, 250 cubic centimeters of
water is then added, the meat acids are neutralized with sodium carbonate,
and the mixture is heated in an Arnold sterilizer for 30
minutes, with occasional stirring. It is then set away in a cold
place for several hours. A small amount of fat collects at the top in
the form of a fatty scum, as it is impossible to remove all of the fat
from the meat before it is chopped. The fatty scum, which hardens
upon standing in the cold, is now removed.
B. The whites of three eggs are mixed with 250 cubic centimeters
of water. The mixture is rendered neutral to phenolphthalein by
means of dilute hydrochloric acid and heated for 30 minutes in the
Arnold sterilizer, with occasional stirring.
A and B are now mixed and 2.5 grams (0.5 per cent) of powdered
calcium carbonate added. The mixture is next run into large sterile
test tubes, or sterile flasks, and sterilized in an Arnold sterilizer on
three successive days.
In addition to the egg-pork mixture described above, culture tubes
of agar and bouillon prepared from pork instead of beef, with the
addition of 1 per cent of glucose, were also used; but the best results
were obtained with the egg-pork medium, as with this medium, the
early development of sour or putrefactive odors furnished a valuable
indication as to the presence of organisms capable of producing sour
or putrefactive changes in meat.
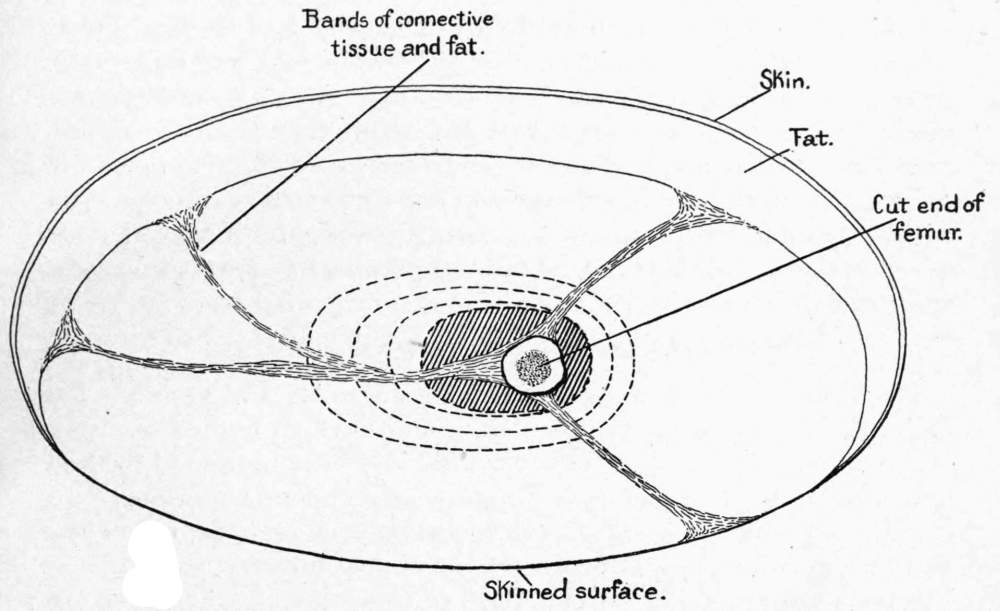
The hams were sectioned through the body, the femur, or “middle
bone,” as it is known in packing-house parlance, being cut at a point
about 1-1/2 or 2 inches below its head. A cross section of a ham thus
cut is shown in figure 1. After sectioning, the hams were subjected
to a microscopical, bacteriological, and chemical examination as
follows:
Microscopical examination.—Bits of muscular tissue, taken from
various points, were teased out in salt solution and the condition of
the muscle fibers noted. Smear preparations were also made from
bits of muscular tissue and from the bone marrow, and these were
stained and subjected to microscopical examination. Portions of
the meat were also hardened and cut into microscopic sections, which
were stained and mounted for histological and bacteriological study.
Bacteriological examination.—In the bacteriological examination
of sour hams, especial attention was directed to the detection of
anaerobic species, as it seemed reasonable to suppose that if the
changes taking place in sour hams were due to bacteria these bacteria
would in all likelihood be anaerobes (i. e., organisms which develop
in the absence of oxygen). This assumption was based upon the fact
that, as a rule, souring begins in the interior of the ham next to the
bone, and, furthermore, the hams are cured in large vats where they
are completely submerged in the pickling fluids, so that any bacteria
which develop within the bodies of the hams while they are in cure
are probably restricted to practically anaerobic conditions.
Cultures were made from the interiors of the hams at various points
by first searing the cut surface thoroughly with a heavy metal spatula
and then cutting out, by means of sterile scissors and forceps, plugs
of meat about 1 cm. square. The plugs of meat were then dropped
into tubes containing the egg-pork medium and pushed down to the
bottom of the tubes, where they were held in place by the chopped
meat above; in this way conditions favorable for the development
of anaerobic organisms were obtained. In inoculating the pork-agar
tubes, the medium was first boiled to expel any inclosed air and cooled
to 43° to 45° C; the plugs of meat were then dropped into the tubes
and the agar rapidly solidified by plunging the tubes in cold water;
in this way the bits of meat were inclosed in the agar at the bottom
of the tubes, affording suitable conditions for anaerobic growth.
Aerobic and anaerobic plates were also made from the meat, and in
most cases bouillon tubes were also inoculated. Cultures were always
taken from the bone marrow as well as from the meat. Novy jars
were also used for obtaining anaerobic conditions in growing the cultures.
Chemical examination.—In order to determine whether the souring
was connected with or dependent upon a lack of penetration of the
pickling fluids to the interior of the meat, the hams were further subjected
to a chemical examination and the content of the meat in
sodium chlorid and potassium nitrate determined at varying depths.
The sour hams examined were obtained from four different packing
establishments. All of the hams studied were “sweet-pickle hams”
which had not been smoked. The sour hams selected for examination
were good typical body sours, in which the sour odor was well developed,
but not of the very pronounced or putrefactive type.
The sour odor in every case was found to be more pronounced next
to the bone, being usually rather more pronounced just behind the
bone, that is, on the fat side of the bone. The sour odor in each
instance was confined to an area of meat immediately surrounding
the femur and extending out through the body of the ham for a variable
distance, as shown by the dotted lines in figure 1, but in no case
did the sour odor extend all the way to the margin of the meat, nor
did it as a rule extend below the tibio-femoral articulation, the shank
proper and the bone marrow of the shank (i. e., of the tibia) being
usually sweet. The butt portion of the hams—that portion above
and behind the hitch bone (symphasis pubis)—was also sweet.
Immediately after sectioning, the sour areas, as a rule, could be
readily distinguished by a difference in color. In the freshly cut hams
the muscular tissue near the bone, where the sour odor was more
pronounced, exhibited a slight but distinct grayish hue, at times having
a slight greenish tinge; in other words, the muscular tissue in the
sour areas lacked the normal bright red color of the sound meat and
was distinctly lighter in color than the surrounding tissues. Upon
exposure to air, however, the lighter, grayish, sour areas tend to
assume a reddish hue and become much less pronounced than in the
freshly cut ham. After the cut surface of the ham has been exposed
to the air for some time it may be difficult to distinguish the sour
areas by any difference in color.
Bul. 132, Bureau of Animal Industry, U. S. Dept. of Agriculture. Plate I.
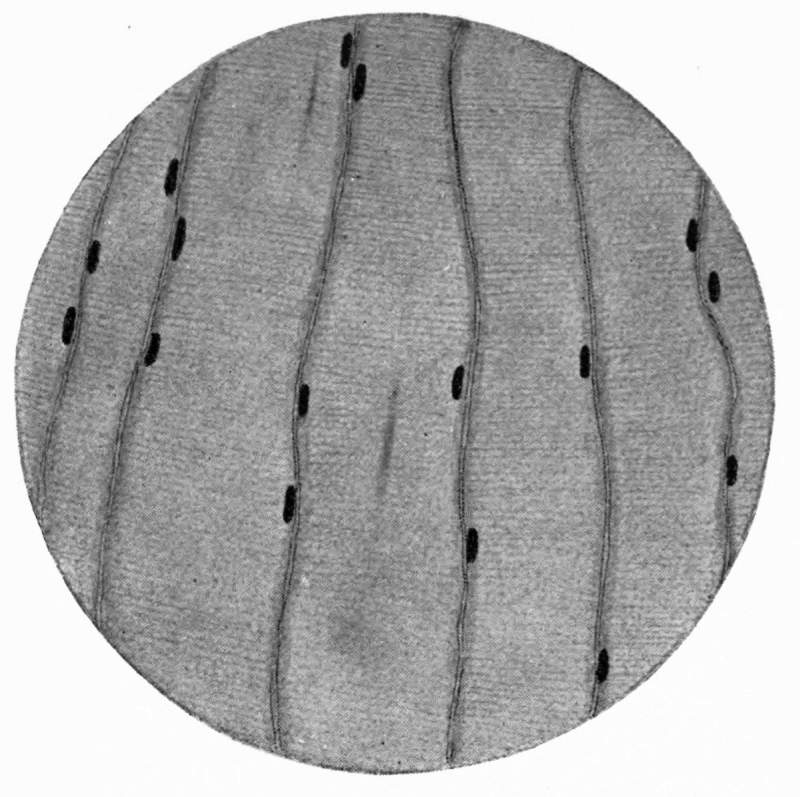
Fig. 1.—Section of Muscular Tissue from Sound Ham, Showing
Muscle Fibers Cut Longitudinally; Nuclei Sharply Defined
and Cross Striation Distinct.
(Pen-and-ink drawing made with camera lucida from section stained with
hematoxylin and eosin to show histological structure.× 320.)
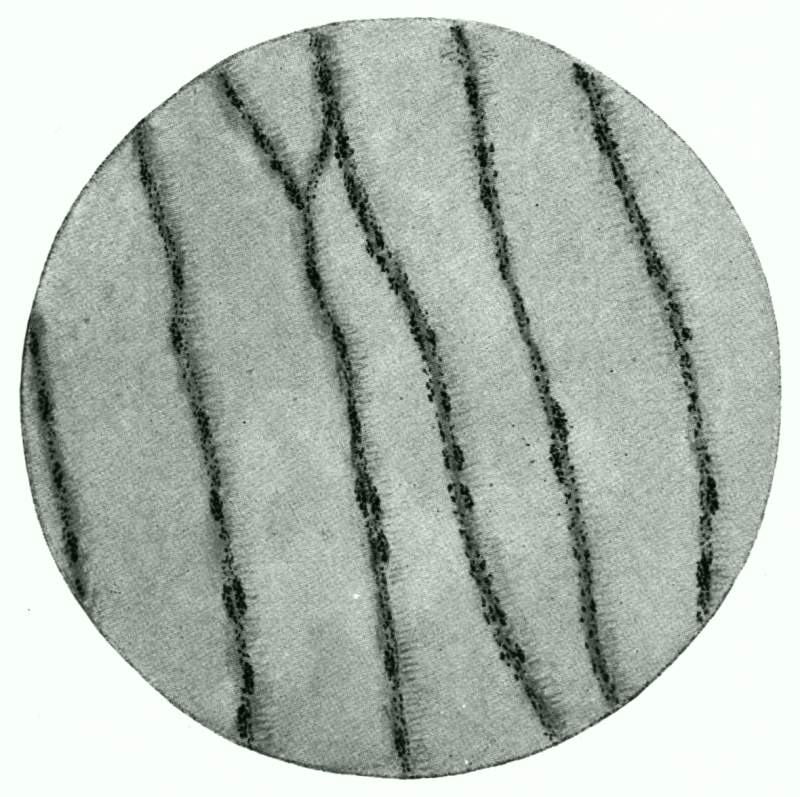
Fig. 2.—Section of Muscular Tissue from Sour Ham, Showing
Muscle Fibers Cut Longitudinally; Nuclei Undergoing Disintegration
and Cross Striation Indistinct.
(Pen-and-ink drawing made with camera lucida from section stained with
hematoxylin and eosin to show histological structure.× 320.)
Bul. 132, Bureau of Animal Industry, U. S. Dept. of Agriculture. Plate II.

Fig. 1.—Section Through Muscular Tissue of Ham which has
Undergone Natural or Spontaneous Souring, Showing Distribution
of Bacilli Between the Muscle Fibers, which are Cut
Obliquely. The Dark Masses Between the Muscle Fibers
Represent Clumps of Bacilli.
(Pen-and-ink drawing made with camera lucida from section stained with
hematoxylin and eosin to show histological structure.× 320.)
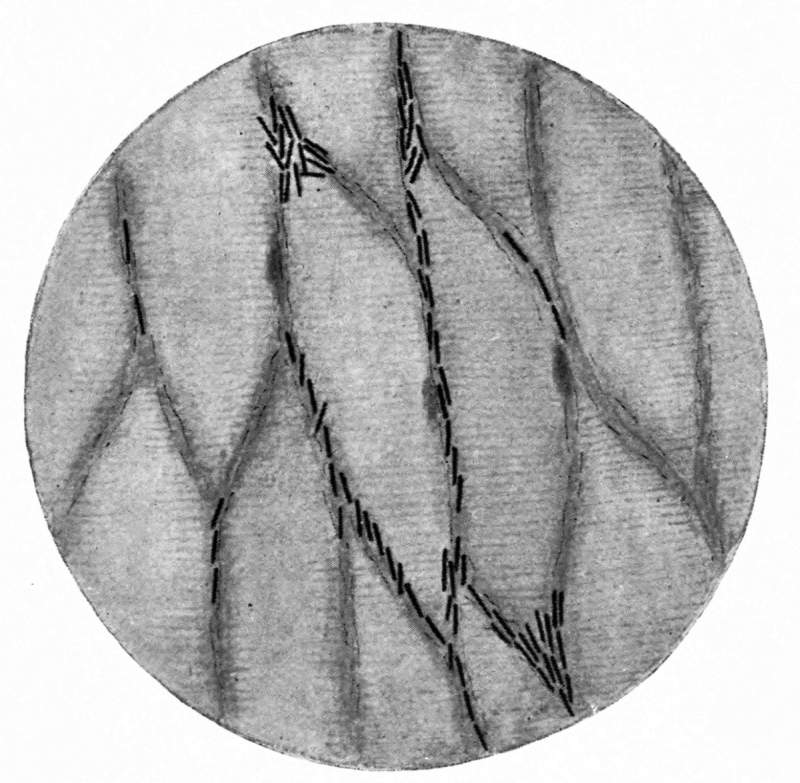
Fig. 2.—Section Through Muscular Tissue of Ham which has
Undergone Natural or Spontaneous Souring, Showing Individual
Bacilli Between the Muscle Fibers, which are Cut Somewhat
Obliquely. Nuclei have Lost Sharp Outline and Cross Striation
is Indistinct.
(Pen-and-ink drawing made with camera lucida from section stained with
hematoxylin and eosin to show histological structure.× 320.)
In the sour areas near the bone the muscular tissue was distinctly
softer; that is, it broke and cut more readily than the surrounding
tissues. This was usually quite noticeable in cutting out plugs of
the meat for making cultures. In a ham which shows pronounced
souring the muscular tissues in the worst affected areas may become
quite soft and even slightly gelatinous.
The sour areas, when tested with litmus paper, frequently showed
a slight but distinct alkaline reaction. When aqueous extracts of
the sour meat, however, were titrated with phenolphthalein they
were found to be acid.
In preparations made by teasing out bits of the meat in physiological
salt solution, the cross striation of the muscle fibers from the sour
areas was found to be much less distinct than in similar preparations
taken from sound portions of the meat or from sound hams. At
times it was found that the muscle fibers in the sour areas had completely
lost their cross striæ, but the longitudinal striation could still
be made out. In cases where the souring was pronounced there was
sometimes complete loss of both longitudinal and cross striation; in
these cases the muscle fibers appeared to have undergone slight swelling
and the protoplasm exhibited a finely granular appearance.
In stained sections of the sour meat another striking change was
noticed in the disintegration of the nuclei of the muscle fibers, which
are at times completely broken up, appearing as bluish granular
masses in sections stained with hematoxylin and eosin.(Compare
figs. 1 and 2 of Pl. I.)
In sections stained by the Gram-Weigert method to show the presence
of bacteria, a large Gram-staining bacillus was noted between
the muscle fibers in the connective-tissue elements of the muscle.
In some of the sections these bacilli were present in great numbers,
sometimes in densely packed clumps or masses, while in other sections,
or in other portions of the same section, they were only sparsely distributed
between the muscle fibers. Where the bacteria were more
numerous the histological changes in the muscle fibers, especially the
breaking down of the nuclei, were more noticeable. The intermuscular
connective tissue had apparently furnished paths of least resistance
along which the organism followed. In Plate II, figures 1 and
2, the bacteria are shown between the muscle fibers under low and
high power magnifications.
In Plate II, figure 1, under the low-power magnification, the bacteria
appear as dark clumps or bands between the muscle bundles.
Under the high power they are shown following along the sarcolemma
sheaths between the muscle fibers.
In order to determine whether there was any difference in regard
to the penetration of the pickling fluids in the sour hams as compared
with sound hams, a series of four sour hams were subjected to a
chemical examination in comparison with four sound hams. All
were sweet-pickle hams and were obtained from the same packing
establishment. They were all of the same cure and the same approximate
age (i. e., length of cure) and the same approximate weight.
In taking samples for chemical analysis, the following procedure
was adopted: A section about 2-1/2 inches wide was cut from the center
of the body. The two ends of this section were then trimmed off
along the lines L-M and N-O, as shown in figure 2. Beginning at the
skinned surface, four slices, A, B, C, and D, were then made, as indicated
by the dotted lines. Slice B contained the bone in each
instance. Slice D was practically all fat. Each slice was ground
separately in a meat chopper and the sample thoroughly mixed before
taking out portions for analysis.
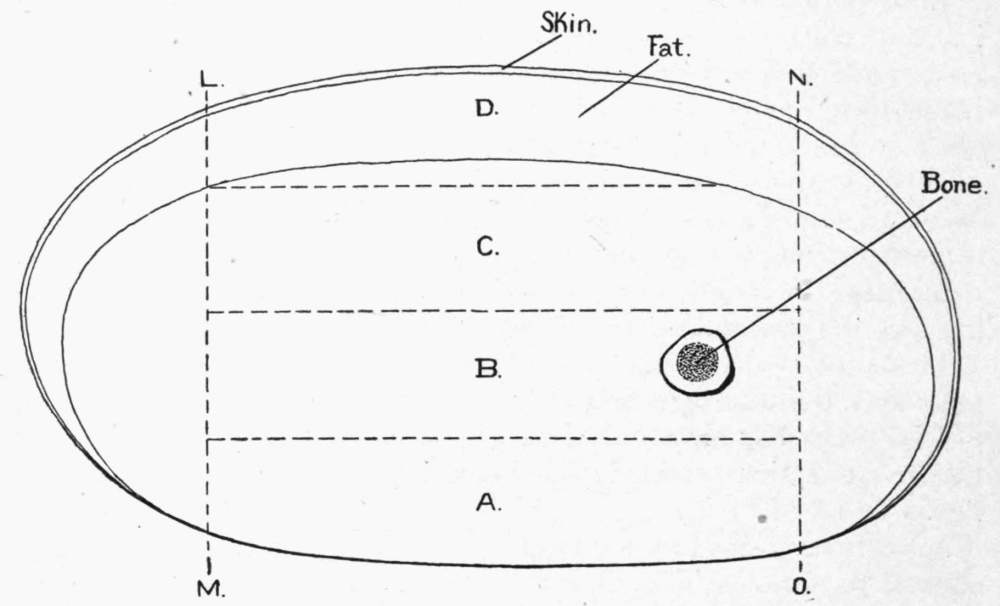
Fig. 2.—Cross section through body of ham to show method of sampling for chemical analysis. A, slice
below bone; B, bone slice; C, slice above bone; D, fat slice.
As all of the hams examined were mild-cure hams, that is, had
been pumped in the shank only, the pickling fluids in order to reach
the bodies of these hams had to penetrate chiefly from the skinned
surface of the ham, as little if any penetration takes place through
the thick skin of the ham.
The analyses[3] shown in the following tables therefore indicate the
degree of penetration of the pickling fluids.
Analyses of sour hams.
| No. |
Description. |
Slice. |
NaCl. |
KNO₃. |
|
|
|
Per cent. |
Per cent. |
| 1 |
Sour body |
A |
6.18 |
0.175 |
|
|
B |
4.83 |
.224 |
|
|
C |
3.65 |
.299 |
|
|
D |
1.03 |
.074 |
| 2 |
do |
A |
5.34 |
.174 |
|
|
B |
3.70 |
.150 |
|
|
C |
2.79 |
.174 |
|
|
D |
1.12 |
.012 |
| 3 |
do |
A |
5.04 |
.125 |
|
|
B |
4.08 |
.149 |
|
|
C |
2.72 |
.099 |
|
|
D |
1.19 |
.048 |
| 4 |
do |
A |
7.78 |
.250 |
|
|
B |
5.31 |
.100 |
|
|
C |
4.76 |
.200 |
|
|
D |
1.96 |
.048 |
Analyses of sound hams.
| No. |
Description. |
Slice. |
NaCl. |
KNO₃. |
|
|
|
Per cent. |
Per cent. |
| 1 |
Sound |
A |
5.80 |
0.211 |
|
|
B |
4.83 |
.188 |
|
|
C |
3.86 |
.221 |
|
|
D |
1.33 |
.063 |
| 2 |
do |
A |
4.94 |
.197 |
|
|
B |
4.08 |
.149 |
|
|
C |
3.05 |
.223 |
|
|
D |
1.56 |
.059 |
| 3 |
do |
A |
5.92 |
.173 |
|
|
B |
4.29 |
.099 |
|
|
C |
4.12 |
.139 |
|
|
D |
2.32 |
.049 |
| 4 |
do |
A |
5.53 |
.119 |
|
|
B |
4.89 |
.079 |
|
|
C |
4.32 |
.099 |
|
|
D |
2.19 |
.041 |
Taking an average of the four slices in each ham so as to get an
average for the entire ham, and comparing the sour hams with the
sound hams, we have the following comparison:
|
|
NaCl. |
KNO₃. |
| Average for 4 sour hams (entire ham) |
per cent. |
3.84 |
0.143 |
| Average for 4 sound hams (entire ham) |
do |
3.93 |
.131 |
These figures show practically no difference between the sour and
the sound hams as regards the sodium chlorid and potassium nitrate
content of the entire ham.
If, now, we compare the bone slices—and these afford really a
better basis for comparison, as in sour-body hams the souring is
always more pronounced around the bone—we have the following
figures:
|
|
NaCl. |
KNO₃. |
| Average for 4 sour hams (bone slice) |
per cent. |
4.48 |
0.155 |
| Average for 4 sound hams (bone slice) |
do |
4.52 |
0.129 |
Here, again, we find no essential difference between the sour and
the sound hams, and we must conclude from these analyses that
souring does not depend upon or result from a lack of penetration
of the pickling fluids.
It seems probable that in mild-cure hams, which are pumped in the
shank only, the souring begins in the upper portion of the shank and
extends upward along the bone into the body of the ham, and that
it takes place before the pickling fluid has penetrated to the interior
of the ham. When the pickling fluid reaches the interior of the ham
it tends to inhibit the souring, which, as will be shown later, is due
to the development of bacteria within the bodies of the hams. The
growth of the bacteria, however, within the bodies of the hams and
the histological changes in the muscle fibers do not seem to interfere
with the penetration of the pickling fluids.
In all of the sour hams which were examined bacteriologically a
large anaerobic bacillus was found to be constantly present. From
several of the hams this bacillus was obtained in pure culture; that is,
it was the only organism present in cultures made from the sour
meat and from the bone marrow of the femur. Such cultures, when
held at room temperature, gave, at three days, a sour-meat odor
exactly resembling that obtained from sour hams.
In many of the sour hams other bacteria were found in association
with the anaerobic bacillus noted above. These other bacteria, however,
were not constant, being sometimes present and sometimes
absent. Among the other bacteria noted in the sour hams, the
following forms occurred most frequently:
1. A nonmotile, gram-positive bacillus, measuring from 1.5 to 4
microns in length by 0.5 micron in breadth, sometimes in chains and
filaments.
2. A small, nonmotile, gram-negative bacillus, about the size of
Bacillus coli and usually in pairs.
3. A large micrococcus.
Sometimes one and sometimes all of these bacteria were present
in a given ham. They were encountered most frequently in hams
which had been pumped in both body and shank, and were probably
ordinary pickle bacteria. They were not strict anaerobes, but
belonged to the class of facultative or optional anaerobes; that is,
organisms which will grow either with or without free oxygen.
These bacteria were isolated and grown on the egg-pork medium,
but failed to give any characteristic sour or putrefactive odors, and
were therefore discarded.
A series of sound hams, all of them of mild cure—that is, hams
which had been pumped in the shank only—were also examined
bacteriologically. In examining these hams cultures were taken
at varying depths, beginning at the skinned surface and going backward
toward the fat. Cultures were also taken from the bone
marrow of the femur. In the cultures taken near the skinned
surfaces the ordinary pickle bacteria were obtained, but these did
not, as a rule, extend beyond a depth of 3 centimeters below the
skinned surface. The cultures taken from the deeper portions of
the hams and from the bone marrow of the femur were entirely
negative—that is, failed to show any growth—and the anaerobic
bacillus noted in the sour hams was not encountered in any of the
cultures made from these hams.
The anaerobic bacillus isolated from the sour hams was found
to correspond in morphology with the organism noted in the microscopic
sections made from the muscular tissue. In view of this
fact and the fact that it was constantly present in the sour hams
examined, and was capable of producing in egg-pork cultures a
sour-meat odor of the same nature as that obtained from sour hams,
this organism was subjected to further study and experimentation.
The experiments which follow were conducted at two different
packing establishments in one of the larger packing centers of the
country. The officials at each of these establishments showed
great interest in the experiments and were most courteous and
obliging in supplying the necessary materials.
The first question to be decided was whether the bacillus isolated
from sour hams was actually capable of causing ham souring. The
bacillus in question had, when cultivated on the egg-pork medium,
given rise to a sour odor similar to that obtained from sour hams,
but this was not regarded as proof positive that the organism was the
actual cause of souring in hams. The proper way to decide this
point seemed to be to inoculate hams with the bacillus and then
subject these hams to the regular method of cure and see whether
they became sour, just as the pathogenic properties of a disease-producing
organism are determined by the inoculation of experiment
animals. The first two experiments which follow were designed
to decide this point.
It was regarded as important to conduct similar experiments
at two different establishments, in order to determine whether the
same results would be obtained under the somewhat different conditions
imposed by different methods of cure. The two experiments
which follow were carried out, therefore, at different establishments.
Experiment I.
In carrying out this experiment four tierces of hams were “put
down” or “packed”—that is, placed in cure. Two of the tierces
were given the fancy or mild cure and two the regular or stronger cure.
The hams in two of the tierces, one mild and one regular cure, were
injected with a culture suspension of the bacillus; the other two tierces
were not injected with culture and were put down to serve as checks on
the cure. Hams weighing from 12 to 14 pounds were used for the mild
cure, while for the regular cure hams weighing from 14 to 16 pounds
were used. This was in accordance with the general rule which prevails
in packing houses, the lighter hams being subjected to the mild
cure and the heavier hams to the regular cure. The only difference
between the mild and the regular cure in this experiment lay in the
pumping. The hams which were given the mild cure were pumped
in the shank only, while those given the regular cure were pumped
in the body as well as in the shank.
All of the hams had received the usual 48-hour chill. They were
all pumped with the same pumping pickle and cured in the same
curing pickle, and were in cure for the same length of time. The
pumping and curing pickles used were the regular pumping and
curing pickles of the establishment at which the experiment was
carried out, and the hams were cured in accordance with the fancy
and regular cures as practiced at this establishment.
The hams were packed in new tierces which had been thoroughly
scalded with boiling water. The tierces were held in a curing room
which was kept at an average temperature of from 34° to 36° F.,
the temperature occasionally going as high as 38° and 40° F., but
never above 40° F. The hams were left in cure for about 70
days, which is a little longer than the usual cure. The tierces were
rolled three times during the cure. At the end of the cure the hams
in all four tierces were carefully tested by an expert meat inspector,
who knew nothing of the treatment which the hams had received.
The hams in two of the tierces were inoculated with a culture
suspension prepared as follows: Ten tubes of egg-pork medium, each
tube containing approximately 10 cubic centimeters of the medium,
were inoculated with the bacillus and held at room temperature
(20° to 25° C.) for six days. The cultures were then filtered through
sterile gauze into a large sterile flask; this was done in order to
remove the particles of meat, which might otherwise have clogged
the syringes used in inoculating the hams. In transferring the contents
of the culture tubes to the filter the tubes were washed out
with sterile physiological salt solution (0.6 per cent sodium chlorid),
and the meat particles on the filter were afterwards washed with
the salt solution, a sufficient quantity of the latter being used to
bring the total volume of filtrate to 400 cubic centimeters. A
microscopic preparation from the filtrate showed the organisms in
large numbers, with an occasional rod showing a large terminal
spore. This suspension was used for the injection of 40 hams, each
ham being given 10 cubic centimeters, or the equivalent of 2.5 cubic
centimeters of the original culture. The hams were injected with the
culture suspension by means of a sterile syringe carrying a long 5-inch
needle. The needle was thrust well into the body of the ham at a
point near the upper end of the middle bone or femur, the latter
being used as a guide in inserting the needle and the injection being
made into the tissues just behind and a little to one side of the
upper end of the femur.
The details of the experiment were as follows:
Tierce No. 1 (fancy cure).—This tierce contained 20 hams weighing from 12 to 14
pounds each. These hams were pumped in the shank only. Immediately after
pumping they were injected with 10 cubic centimeters each of the liquid culture
or suspension described above. After injection the hams were immediately packed
in the tierce, which was then headed up, filled with the regular curing pickle, and
placed in cure.
Result: When tested at the end of the cure all of the hams in this tierce save one
were found to be sour. In 10 of them the souring was very marked throughout the
body of the ham and extended into the shank as well. In six the souring was very
marked in the body of the ham, but did not extend into the shank. In three there
was slight but well-marked souring in the body of the ham with no souring in the
shank, and one remained sweet. The probable explanation of the variation in
the degree and the extent of the souring will be discussed later. The bone marrow
of the femur or middle bone was tested in all of the hams and found to be sour in
18. In one of the hams which showed only slight souring in the body the souring
did not extend through to the bone marrow, and in the ham which remained sweet
the bone marrow was also sweet. The fact that one ham in this tierce remained
sweet was in all likelihood due to an oversight in making the inoculations. In making
the inoculations the hams were spread out in a row on a table by a packing-house
assistant, who removed the hams as soon as they were inoculated and placed them in
tierces; and it is more than probable that the assistant removed one of the hams before
it was inoculated in the interval when the writer was busy filling the syringe for
the next inoculation.
Tierce No. 2 (fancy cure).—This tierce contained 20 hams of the same average weight
as the preceding. They were pumped in the shank only, but were not injected with
culture, being put down to serve as checks on the hams in tierce No. 1. These hams,
therefore, were subjected to exactly the same cure and were held under exactly the
same conditions as those in tierce No. 1, the only difference being that the hams in
this tierce were not injected with culture.
Result: When tested at the end of the cure all of the hams in this tierce were found
to be perfectly sound and sweet, showing that the curing in this instance was properly
carried out and that the souring of the hams in tierce No. 1 was undoubtedly due to
the injections of culture which they received.
Tierce No. 3 (regular cure).—This tierce contained 20 hams weighing from 14 to
16 pounds each. These hams were pumped in the shank and also in the body. Immediately
after pumping they were each injected in the same manner as those in tierce
No. 1 with 10 cubic centimeters of culture. The hams were then packed in tierce and
placed in cure.
Result: At the end of the cure 9 of the hams were found to be sour, while 11
remained sweet. Of the 9 hams which became sour, 1 showed very pronounced souring
in the body and in the shank as well, 3 showed very pronounced souring in the
body, 1 showed pronounced souring in the body, and 4 slight souring in the body.
The bone marrow of the femur was tested in all of the sour hams and was found to be
sour in 7. In 2 of the sour hams which showed slight souring in the body the souring
noted in the meat had not extended through to the bone marrow.
Tierce No. 4 (regular cure).—This tierce contained 20 hams of the same average weight
as those in tierce No. 3, and, like the latter, were pumped in both shank and body, but
were not injected with culture. This tierce was put down to serve as a check on
tierce No. 3 and was held under exactly the same conditions, the only difference being
that these hams were not injected with culture.
Result: At the end of the cure the hams were carefully tested and all were found to
be perfectly sound and sweet.
Results of Experiment I.
| No. of tierce. |
Number
of hams. |
Average
weight of hams
Pounds. |
Cure. |
How pumped. |
Treatment. |
Condition at end of cure. |
| Number of sour hams |
Percentage of sour hams |
| 1 |
20 |
12-14 |
Fancy |
Shank only |
Each ham injected
with 10 c. c. of culture. |
19 |
95 |
| 2 |
20 |
12-14 |
do |
do |
Not injected with culture;
check on tierce 1. |
0 |
0 |
| 3 |
20 |
14-16 |
Regular |
Shank and body |
Each ham injected
with 10 c. c. of culture. |
9 |
45 |
| 4 |
20 |
14-16 |
do |
do |
Not injected with culture;
check on tierce 3. |
0 |
0 |
Three hams from each tierce were selected for bacteriological and
histological examination. From tierces 1 and 3, which contained
the injected hams, three of the most pronounced “sours” were
selected from each tierce. In examining the hams bacteriologically
the following method was adopted: The hams were sectioned near
the center of the body and the larger or butt end turned up so as to
expose the cut surface. A cross section of a ham thus cut is shown
in figure 3.
Cultures were taken at the points indicated by the numbers and
from the exposed bone marrow of the femur by first searing the surface,
and then taking out plugs of the meat or marrow by means of
sterile instruments. The plugs of meat or marrow were dropped
into tubes containing egg-pork medium and pushed to the bottom of
the tubes by means of a sterile platinum wire. In the cultures made
from the sour hams from tierces 1 and 3, which were injected with
culture, the bacillus with which these hams were injected was found
in practically every culture, although it was sometimes absent in
the cultures taken at points near the skinned surfaces of the hams
(i. e., at points 1, 4, and 5 in fig. 3). In the cultures taken from the
meat, the bacillus was not always present in pure culture, but this is
not to be wondered at when we remember that the pickling fluids
often contain large numbers of bacteria of various kinds, and these,
of course, find their way into the hams in the pickling fluids. Especially
is this true of the hams which are pumped in the body, where
bacteria are actually pumped into the bodies of the hams in the
pumping pickle. In the case of hams which are not pumped in
the body, the pickle bacteria do not appear to penetrate the body of
the ham to any great depth.
In figure 3 the plus signs after the figures represent the distribution
of the sour-ham bacillus in one of the hams from tierce 1, and this
may be taken as a typical example of the other sour hams which were
examined in this experiment. It should be explained that the
shaded areas are not intended to represent the actual limits of souring,
but simply the areas in which the sour odor was most pronounced
and from which it could be readily obtained with the trier. In
comparing the regular and mild cure hams, it was found that the
areas of souring as defined with the trier were more restricted in the
regular cure hams, and this was undoubtedly due to the additional
pumping which these hams received, whereby the growth of the
bacillus was partially inhibited.
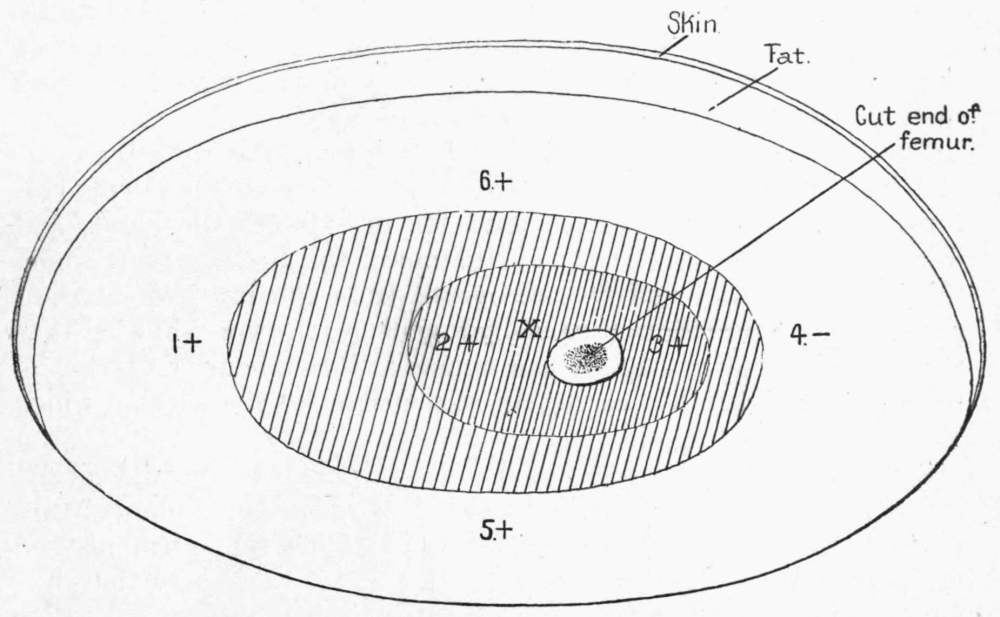
Fig. 3.—Cross section through body of artificially soured ham, showing sour areas and points at which
cultures were taken. Darker shading indicates sour area in hams pumped in body and shank; light
shading indicates sour area in hams pumped in shank only; figures indicate points at which cultures
were taken; plus signs indicate presence of bacillus; minus sign indicates absence of bacillus; X indicates
point of inoculation.
It will be noticed that the sour-ham bacillus was present in cultures
taken at points outside the shaded areas, indicating that the
organism had extended generally throughout the bodies of the hams.
As the hams were inoculated at a point just to one side of and a
little behind the femur (i. e., at the point X in the figure), the presence
of the bacillus generally throughout the hams would indicate
a very extensive multiplication of the original bacilli with which the
hams were injected. In view of the fact that the bacillus in question
is nonmotile, the spread of the bacilli throughout the hams must
result simply from subdivision and growth by extension, and in
spreading throughout the hams the bacilli appear to follow along the
connective tissue bands which afford paths of least resistance. In the
cultures made from the bone marrow the bacillus was recovered in
pure culture from each of the hams examined, and it is probable that
the bacillus finds its way into the bone marrow from the meat by
following along the small arteries which pass through the bone. The
fact that the bacillus was found in pure culture (i. e., uncontaminated)
in the cultures made from the bone marrow is explained probably
by its capacity for growth by extension, and also by the fact that the
pickling solutions probably do not reach the bone marrow until late
in the curing and then only to a limited extent. The bacteria which
ordinarily occur in pickling fluids are not strict anaerobes and are not
placed under the most suitable conditions for growth when they
reach the interior of the ham, for it seems probable that in the interior
of hams which are totally submerged in pickling fluids the amount
of available oxygen must be extremely small. The ordinary pickle
bacteria, therefore, would not multiply as rapidly in the interior of
the hams and would not find their way into the bone marrow as
soon as would a strictly anaerobic organism.
Pure cultures of the sour-ham bacillus, recovered from the meat
and bone marrow of the injected hams, were compared with cultures
of the original bacillus used for inoculating the hams, and
were found to be identical. Furthermore, the bacillus with which
the hams were injected was recovered from the injected hams at
points far removed from the original point of injection, showing that
the organism had multiplied and extended throughout the bodies of
the hams and that it was clearly responsible for the souring which
the hams had undergone.
Sound hams from tierces 2 and 4 were examined bacteriologically
in the same manner as the injected hams, and some of the cultures
showed the ordinary pickle bacteria, but in not a single instance did
egg-pork cultures yield a sour odor, and in no case could the sour-ham
bacillus be demonstrated in any of these hams.
Microscopic sections and teased preparations of the muscle fibers
in salt solution were prepared from several of the sour hams in this
experiment, and these preparations showed the same histological
changes and the same distribution of bacilli as noted in the natural
sours.
In Plate III, figures 1 and 2, sections are shown of artificially soured
hams, that is, hams which were artificially soured by injections of culture;
and if these figures be compared with the sections made from
hams which had undergone spontaneous souring (see Pl. II, figs. 1 and
2) the similarity in the form and distribution of the bacilli will be at
once apparent.
Bul. 132, Bureau of Animal Industry, U. S. Dept. of Agriculture. Plate III.
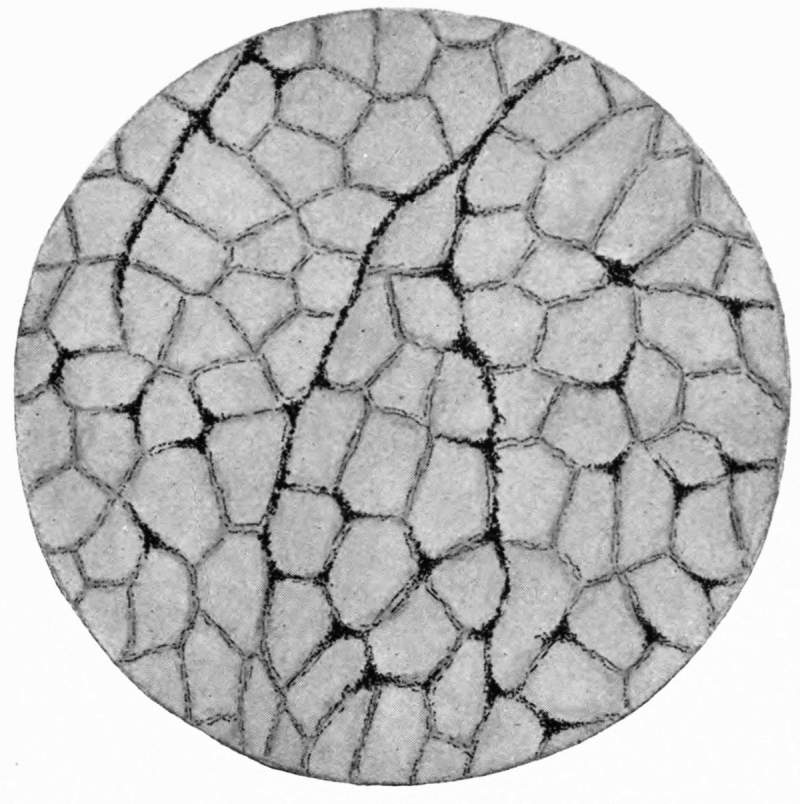
Fig. 1.—Section Through Muscular Tissue of Artificially Soured
Ham, Showing Distribution of Bacilli Between the Muscle
Fibers, which are Shown in Cross Section. The Dark Lines and
Masses Between the Muscle Fibers Represent Clumps of
Bacilli.
(Pen-and-ink drawing made with camera lucida from section stained by
the Gram-Weigert method to show bacteria. × 85.)
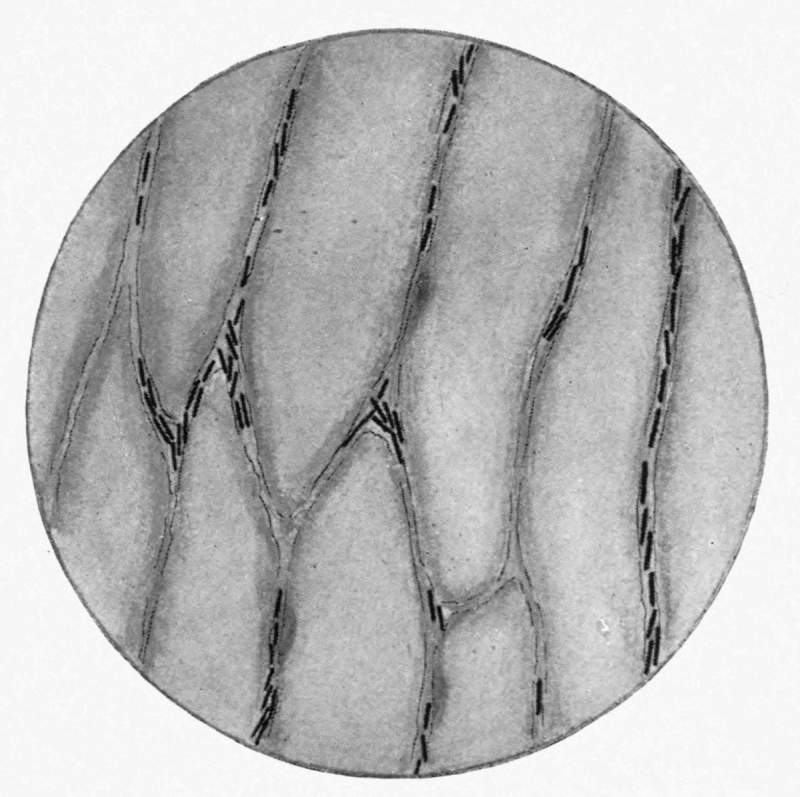
Fig. 2.—Section Through Muscular Tissue of Artificially Soured
Ham, Showing Individual Bacilli Between the Muscle Fibers,
which are Cut Longitudinally.
(Pen-and-ink drawing made with camera lucida from section stained by
the Gram-Weigert method to show bacteria. × 320.)]
Summary and discussion of Experiment I.—Comparing tierces 1
and 2, where the hams were pumped in the shank only, the only
difference being that the hams in tierce 1 were inoculated with culture
while those in tierce 2 were not, we find that in tierce 1 nineteen out
of twenty, or 95 per cent, of the hams became sour, whereas in tierce 2
all of the hams remained sweet. In view of the fact that these tierces
were held under exactly the same conditions, we must conclude that
the souring of the hams in tierce 1 was due to the injection of culture
which they received.
Comparing tierces 3 and 4, where the hams were pumped in both
shank and body, the hams in tierce 3 being injected with culture
while those in tierce 4 were not, we find that in tierce 3 nine out of
twenty, or 45 per cent, of the hams became sour, whereas in tierce 4 all
of the hams remained sweet. As the conditions of cure were the same
for all four tierces, we must again conclude that the souring of the
hams in tierce 3 was directly attributable to the injections of culture
which they received.
If now we compare tierces 1 and 3, the two tierces which were
injected with culture, we find that in the case of tierce 1, where the
hams were pumped in the shank only, 95 per cent became sour;
whereas in the case of tierce 3, where the hams were pumped in both
shank and body, only 45 per cent became sour. In other words, the
percentage of souring in those hams which were pumped in the body
as well as in the shank was 50 percent less than in those hams which
were pumped in the shank only. Inasmuch as the only difference
in the treatment accorded tierces 1 and 3 lay in the additional
pumping given the hams in tierce 3, we must conclude that the
marked diminution in the percentage of souring in the case of tierce
3 was undoubtedly due to the additional pumping which these hams
received, the hams being saturated at the start with the pumping
pickle. It will be shown later that both sodium chlorid and potassium
nitrate exert an inhibitory effect upon the bacillus with which the
hams were injected, which directly bears out the foregoing conclusion.
In tierces 2 and 4, the two check tierces which were not injected
with culture, all of the hams were sweet at the end of the cure, showing
that the conditions under which the experiment was carried out were
entirely favorable to a successful cure.
The sour odor obtained from the artificially soured hams in this
experiment was pronounced by the meat inspector who tested the
hams, and who was entirely unaware of the treatment they had
received, to be identical with the usual sour odor which characterizes
hams that have undergone spontaneous souring; in other words,
there was no difference in odor between these artificially soured hams
and natural sours.
With regard to the variation in the degree and the extent of the
souring exhibited by the individual hams in the two inoculated
tierces, where some of the hams showed pronounced souring throughout
the body and shank, while others which had been injected with
the same amount of culture showed only slight souring in the body,
several factors must be considered, viz:(1) Differences in the reaction
of the meat of the individual hams which may have exerted an influence
on the growth of the bacteria with which the hams were injected.
(2) Variations in the texture of the muscle fibers and connective
tissue of the individual hams, permitting in some cases a more rapid
and thorough penetration of the pickling fluids to the interior of the
hams, whereby the inhibitory effect of the sodium chlorid and the
potassium nitrate on the bacteria would come into play earlier.
(3) Variations in pumping, whereby more of the pickling solution was
forced into some of the hams than into others. Probably all three of
these factors would have to be taken into account in explaining the
variation in the degree and extent of the souring exhibited by the
injected hams.
With regard to the souring of the bone marrow, we find that of
nineteen sour hams in tierce 1 eighteen showed sour marrows, while
in tierce 3 nine sour hams showed seven sour marrows. The high
proportion of marrow sours is not surprising when it is recalled that
of the nineteen sour hams in tierce 1 the meat was markedly sour in
sixteen, while of the nine sour hams in tierce 3 the meat was markedly
sour in five. In the case of the four sour hams in tierce 3
which showed slight souring in the body, two of these showed sour
marrows, while in two the marrows were sweet. In this experiment
the percentage of sour hams showing sour marrows corresponds
with the percentage of marrow-sour hams found in the packing
house, where, as has been pointed out before, a ham which is markedly
sour in the body will practically always show sour marrow,
while in hams which show only slight souring in the body the marrow
is involved in about 50 per cent of the cases.
Experiment II.
This experiment was essentially a repetition of Experiment I, but
was carried out at a different packing establishment and under somewhat
different conditions.
Two lots of hams were injected with a culture suspension of the
bacillus at different stages of the cure, or rather at different stages in
the preparation for cure, i. e.,(1) on the hanging floor, previous to
chilling, and (2) after chilling and pumping and immediately before
packing. Three tierces, each containing 20 hams, were put down.
Two of the tierces contained the hams injected with culture, while
the third tierce contained check hams which had not been treated
with culture. Half of the hams in each tierce were pumped
in the shank, while the other half were pumped in both body and
shank. The same pumping and curing pickles were used for all three
tierces, and were the regular pumping and regular curing pickles of
the establishment at which the experiment was carried out. The
hams used were all 14 to 16 pounds in weight and were subjected to
the usual 48-hour chill with an additional chill of 48 hours after they
were cut from the carcass. They were packed in tierces which had
been thoroughly scrubbed and cleaned with boiling water. The
tierces were held in a pickling room at a temperature of 33° to 36° F.,
the temperature never rising above 36° F., and were rolled three
times during the curing period. The hams were in cure for about
eighty days. At the end of the cure the hams were carefully tested by
a trained meat inspector, who knew nothing of the treatment they
had received.
The culture suspension was prepared from 20 tubes of egg-pork
medium in the same manner as that used in Experiment I, the cultures
being diluted with sufficient salt solution to give 400 cubic centimeters
of suspension. The cultures from which the suspension was prepared
had grown at room temperature for ten days. The suspension was
examined microscopically and showed large numbers of the bacilli in
the form of filaments or long chains, with many of the individual
organisms showing large terminal spores. The hams were injected
with the culture suspension in the same manner as those in Experiment
I.
The details of the experiment were as follows:
Tierce No. 1.—Contained 20 hams, each ham being injected with 20 cubic centimeters
of the suspension or the equivalent of 10 cubic centimeters of the original
culture. The hams were injected while on the hanging floor, before they had been
cut from the carcasses and previous to chilling. The carcasses were still quite warm—that
is, had lost but little of their body heat when the injections were made. The
carcasses, which had been carefully tagged, were then run into coolers and given
the usual 48-hour chill, after which the hams were severed from the carcasses and
given an additional 48-hour chill in accordance with the custom of the packing
house at which the experiment was carried out. The hams were next pumped with
regular pumping pickle, 10 being pumped in both body and shank and 10 in shank
only. They were finally packed in a tierce, which was then headed up, filled with
regular curing pickle, and placed in cure.
Result: When tested at the end of the cure it was found that the 10 hams which
were pumped in the shank only were all sour. In each of them the souring extended
throughout the entire ham, in the shank as well as in the body, and was very pronounced,
so much so that they were characterized as “stinkers” by the meat inspector
who assisted in testing them. The bone marrow of the femur or middle bone was
sour in all of these hams. Of the 10 hams which were pumped in both body and
shank 7 showed well-marked souring throughout the body, but the souring did not
extend into the shank. The bone marrow of the femur was found to be sour in 6 of
these hams, while in 1 the souring had not extended through to the bone marrow.
Tierce No. 2.—Contained 20 hams which were chilled and pumped in exactly the
same manner as those in tierce No. 1. These hams were injected with culture after
they had been chilled and pumped, or just before they were placed in cure. The
hams in this tierce, therefore, were injected with culture four days later than those
in tierce 1. The hams were injected with a bacterial suspension prepared in the
same manner as that used for tierce 1, except that the egg-pork cultures from which
the suspension was prepared were 7 days instead of 10 days old. Each ham was
injected with 20 cubic centimeters of the suspension or the equivalent of 10 cubic
centimeters of the original culture. The hams were injected in the same manner as
those in tierce 1.
Result: When tested at the end of the cure, it was found that of the 10 hams which
were pumped in the shank all were sour; in 8 of these the souring was very marked
throughout the body of the ham and extended into the shank; in all of these hams
the souring had extended through to the bone marrow of the middle bone or femur.
Of the 10 hams which were pumped in both body and shank 6 were sour in the body.
These hams were classed by the meat inspector who examined them as “light body
sours,” and in none of them did the souring extend into the shank or through the
bone into the bone marrow of the femur.
Tierce No. 3.—Contained 20 hams which were chilled and pumped in the same
manner as those in the two preceding tierces. These hams were not injected with
culture and were put down to serve as checks on the cure. In other words, they
were pumped with the same pickling fluids, were subjected to exactly the same cure,
and were held under precisely the same conditions as those in the preceding tierces,
the only difference being that the hams in this tierce were not injected with culture.
Result: When tested at the end of the cure, all of the hams in this tierce were found
to be perfectly sound and sweet.
Results of Experiment II.
| No. of tierce. |
Number of hams. |
Average weight
of hams.
Pounds. |
How pumped. |
Treatment. |
Condition at end of cure. |
Number of
sour hams. |
Percentage of
sour hams. |
| 1 |
20 |
14-16 |
10 in shank |
Each ham injected with 20
c. c. of culture prior to chilling and pumping. |
10 |
100 |
| 10 in body and shank |
do |
7 |
70 |
| 2 |
20 |
14-16 |
10 in shank |
Each ham injected with 20
c. c. of culture subsequent to chilling and pumping. |
10 |
100 |
| 10 in body and shank |
do |
6 |
60 |
| 3 |
20 |
14-16 |
10 in shank |
Not injected with culture |
0 |
0 |
| 10 in body and shank |
do |
0 |
0 |
Four hams were selected from each tierce for bacteriological and
histological examination. From tierces 1 and 2, in which the hams
were injected with culture, 4 of the sourest hams were selected from
each tierce. Cultures were made from these hams in the same
manner as described under Experiment I and with the same result—that
is, the sour-ham bacillus was found throughout the bodies of
the hams. Microscopic sections were also prepared from these hams
and showed the same histological changes and the same distribution
of bacilli as noted for the hams in Experiment I.
Summary and discussion of Experiment II.—Comparing tierces 1
and 2, in which the hams were injected with culture, with tierce 3,
where the hams were not injected with culture, we find that in tierce
1 seventeen hams (85 per cent) became sour and in tierce 2 sixteen
hams (80 per cent) became sour, whereas in tierce 3 all of the hams
were sweet. The fact that all of the hams in tierce 3, the check
tierce, were sweet indicates that the conditions were favorable for a
successful cure; and as all three tierces were cured under exactly the
same conditions, the only difference being that the hams in tierces
1 and 2 were injected with culture, whereas those in tierce 3 were not
injected with culture, we must conclude that the souring of the hams
in tierces 1 and 2 was due to the injections of culture which they
received.
Comparing tierce 1 with tierce 2, we find that the hams in tierce 1
showed more extensive souring than did those in tierce 2, this being
especially noticeable in the case of the hams which were pumped in
both body and shank. This difference in the extent or degree of souring
was probably due to the fact that the hams in tierce 1 were
injected while they were still warm and before they had lost their
animal heat, the bacterial suspension thus having a better chance to
become disseminated through the meat. The hams in tierce 2 were
injected with culture after they had been chilled, when the tissues
were more or less contracted and the conditions less favorable for the
dissemination of the suspension throughout the meat. The hams in
tierce 1 were also injected four days earlier than those in tierce 2,
and prior to pumping; and this would explain the greater difference
in the extent of the souring in the case of the hams which were
pumped in both body and shank, as in tierce 1 the bacteria had four
days in which to develop before coming in contact with the pickling
fluids, whereas in tierce 2 the bacteria were injected after the hams
were pumped with pickle and were thus brought into immediate
contact with the pickling fluids, which, as will be shown later, have a
distinct inhibitory action upon the bacillus in question. In the case
of the hams which were pumped in the shank but not in the body
there was not this difference, as in these hams the pickling fluids
must penetrate into the bodies of the hams from the outside. As it
requires some time for the pickling fluids to reach the interior of a
ham, the bacteria were thus afforded quite an interval in which to
develop before being exposed to the inhibitory action of the pickling
fluids. A chemical study of the processes involved in ham curing
has been carried out in the Biochemic Division and the approximate
rate of penetration of the curing pickle determined, and it was found
that it required about four weeks for the interior of a 10-pound ham
which had not been pumped to acquire its maximum percentage of
sodium chlorid.
To recapitulate: In this experiment 40 hams were injected with
culture, half of this number being pumped in the shank only and
half in both body and shank. Of the 20 which were pumped in the
shank only, every ham without exception, or 100 per cent, became
sour. Of those which were pumped in both body and shank, 13, or
65 per cent, became sour. The reduction in the percentage of sours
in the last lot was clearly due to the additional pumping which these
hams received.
If now we compare tierce 2 in this experiment with tierces 1 and 3
in Experiment I—these three tierces being comparable, as they were
all injected with culture at the same stage in their preparation for
cure, that is, subsequent to chilling and pumping—we find, in the
case of the hams pumped in both body and shank, 65 per cent of
sours in Experiment II as against 45 per cent in Experiment I, and
this difference is undoubtedly due to the heavier dose of culture
used in Experiment II, where the hams were given the equivalent
of 10 cubic centimeters of egg-pork culture as against 2-1/2 cubic centimeters
in Experiment I. In the case of the hams which were
pumped in the shank but not in the body, the percentage of sours
was practically the same in the two experiments—in Experiment I
all but one of these hams became sour, while in Experiment II all of
them became sour. The degree or extent of the souring in these last
hams, however, was greater in Experiment II, a result of the heavier
injections of culture which they received.
Summary of Experiments I and II.
Summarizing the results obtained in Experiments I and II, we find
that culture suspensions of the anaerobic bacillus isolated from sour
hams caused souring with great uniformity when injected into the
bodies of sound hams which were pumped in the shank only. In
the two experiments, 40 sound hams which were pumped in the
shank only were injected with culture suspensions of the bacillus,
with the result that 39, or 97.5 per cent, became sour during the
process of cure; and it is quite probable, as we have pointed out
before, that one of these hams was overlooked in making the inoculations,
otherwise the entire lot would have become sour.
The inhibitory action of the pickling fluids upon the bacillus is
well shown in the case of those hams which were pumped in both
body and shank. Out of 40 hams which were pumped in both body
and shank, 22, or 55 per cent, became sour in the process of curing.
Inasmuch as these hams were cured under precisely the same conditions
as the hams which were pumped in the shank only, we must
conclude that the diminution in souring in these hams was undoubtedly
due to the additional pumping which they received, whereby
the bacteria with which these hams were injected were brought into
immediate contact with the strong pumping pickle and their development
thereby inhibited.
In these two experiments it was proven beyond doubt that the
anaerobic bacillus isolated from sour hams was capable of producing
souring when introduced into the bodies of sound hams; and in view
of the fact that this bacillus was constantly present in hams which
had undergone spontaneous or natural souring, and was the only
organism that could be isolated from such hams that was capable of
producing in egg-pork cultures the characteristic sour-ham odor, the
conclusion seems justifiable that this bacillus is an undoubted cause
of the ham souring which occurs in the packing house; and the
results thus far obtained indicate that it is an important, if not the
only, factor concerned in ham souring.
Having established the etiological relation of the bacillus isolated
from sour hams with ham souring, the next point to be considered
was the manner in which this bacillus finds its way into the bodies of
the hams.
Regarding the question of the probable method by which the ham-souring
bacillus enters hams, there were three possibilities to be taken
into consideration:(1) That the bacillus is present in the flesh of
hogs at the time of slaughter,(2) that the bacillus gains entrance
through the pickling fluids,(3) that the bacillus is introduced into
the bodies of the hams in the handling or manipulation which the
hams undergo in preparation for, or during, the process of curing.
In order to throw some light upon this point, a number of fresh
hams—that is, hams which had been chilled but not pumped or subjected
to any other manipulation—were examined bacteriologically,
but in no case could the anaerobic bacillus which was isolated from
sour hams be detected in any of them. The fact that in certain
of the smaller packing establishments which cure their hams without
pumping the percentage of souring is extremely low would also
seem to negative this possibility, for if the bacillus which causes
souring were present in the hams at the time of slaughter, sour hams
would be as frequent at such establishments as at those establishments
which make a practice of pumping. Furthermore, a laboratory
study, biological and chemical, of the bacillus isolated from
sour hams shows that this organism belongs to the class of putrefactive
bacteria, and while such bacteria may be present in the
intestines of healthy animals, as, for example, the bacillus of Bienstock
(Bacillus putrificus), these bacteria do not invade the organs
and tissues of the body until after the death of the animal, and the
packing-house practice of rapidly eviscerating the hogs immediately
after slaughter would certainly preclude this possibility.
With regard to the second possibility, that the bacillus finds its
way into the hams in the curing pickles, it was determined by laboratory
experiment that the addition of 3 per cent of sodium chlorid or
3 per cent of potassium nitrate to laboratory media completely
inhibits the growth of the bacillus. As the pickling solutions always
contain considerably more than these percentages of sodium chlorid
and potassium nitrate, it would be impossible for the bacillus to
multiply in the pickles. Additional laboratory experiments demonstrated,
however, that the bacillus or its spores may remain alive in
the curing pickles for at least thirty days, and it seemed possible that
the curing pickles might become contaminated at times with the
bacilli, and that the bacilli, although incapable of multiplying in the
pickles, might find their way into the bodies of the hams in the
pickling fluids. In order to throw some light upon this point, the
following experiment was carried out:
EXPERIMENT TO SHOW WHETHER INFECTION TAKES PLACE FROM THE CURING PICKLE.
In this experiment two tierces were put down, each containing
20 hams. The hams weighed from 14 to 16 pounds and had received
the usual 48-hour chilling. The pickling solutions employed were
the regular curing pickles of the establishment at which the experiment
was carried out. The curing pickle in one tierce was inoculated
with 400 cubic centimeters of a culture suspension of the bacillus,
prepared in the same manner as that used for the injection of the
hams in tierce 2 in Experiment II. A microscopic preparation made
from a small drop of the culture suspension before adding it to the
pickle showed the bacilli in large numbers, and in the 400 cubic
centimeters of the suspension there were millions of the bacteria.
The curing pickle in the other tierce was left untreated, the hams
in this tierce serving as a check. The tierces used in this experiment,
as in all of the experiments, were thoroughly cleaned with boiling
water before the hams were placed in them. The experiment was
conducted in a pickling room which was held at 33° to 36° F., and
the tierces were rolled three times during the cure. The details of
the experiment are as follows:
Tierce 1.—Contained 20 hams, half of which were pumped in both body and shank
and half in the shank only. As soon as they were pumped the hams were packed in
the tierce. Sufficient curing pickle to fill the tierce was then measured out in a clean
barrel and to it was added the culture suspension. The culture was thoroughly mixed
with the pickle and the latter was then run into the tierce containing the hams.
Result: When tested at the end of the cure, two of the hams which had been
pumped in the shank only showed slight souring in the body. The rest of the hams
were sweet.
Tierce 2.—Contained 20 hams which were pumped in the same manner as those in
tierce 1. The curing pickle was the same as that used for tierce 1, but without the
addition of culture. This tierce was put down as a check on tierce 1, the hams being
cured under exactly the same conditions, but without the addition of culture to the
curing pickle.
Result: One of the hams which was pumped in the shank only developed slight
souring in the body. The remainder of the hams were sweet.
Comparing tierce 1, which contained the inoculated pickle, with
tierce 2, the check tierce which contained uninoculated pickle, we
find there was practically no difference in the final result. In tierce
1 two of the hams developed slight souring, while in tierce 2 one of
the hams became slightly sour. All of these hams had been pumped
in the shank only. The fact that one of the hams in the check tierce
developed slight souring was undoubtedly due to bacterial contamination
in pumping or in the handling which the hams underwent prior
to pickling, and the slight souring of the two hams in tierce 1 must
also be attributed to the same cause or causes, for had the souring
in these last hams resulted from the penetration of the bacteria from
the pickling solution a higher percentage should have become sour.
Furthermore, if the souring of the two hams in tierce 1 had resulted
from the penetration of the bacteria from the curing pickle, the souring
should have been general throughout the bodies of these hams,
whereas the souring was only evident around the bone and was slight
in degree.
From this experiment the conclusion would seem justified that the
bacillus which causes ham souring does not usually find its way into
the bodies of the hams from the curing pickle, although it would be
going too far, perhaps, to say that infection never takes place from
the curing pickle. The experiment, however, indicates clearly that
the curing pickles are certainly not the main channel through which
the hams become infected. In referring to the curing pickles, it
should be understood that we refer here to the pickling solutions in
which the hams are immersed, and not to the pumping pickles. The
possibility of infection through the pumping pickle will be discussed
later.
There are at least three possible ways in which hams may become
infected from the handling which they receive in preparation for, or
during the process of curing, viz: From the thermometers used in
taking the inside temperatures of the hams, from the pumping
needles, and from the billhooks used in lifting the hams.
INFECTION FROM HAM THERMOMETERS.
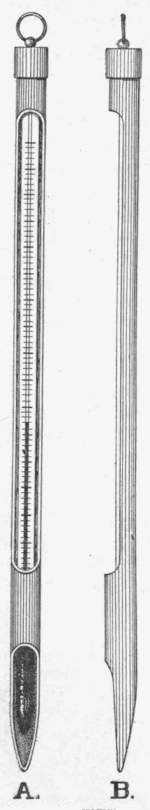
Fig. 4.—Diagrammatic views showing
construction of ham thermometer. A, front view, showing open space
between metal point and mercury bulb, which becomes filled with
particles of meat, grease, and dirt; B, side view.
The packing-house method of taking the temperatures of hams by
means of a pointed, metal-capped thermometer which is thrust deep
into the bodies of the hams has already been referred to, but deserves
to be described somewhat more in detail, as it will be at once apparent
that this manipulation furnishes a ready means
whereby hams may become infected with putrefactive
bacteria. The construction of a ham thermometer
is shown in figure 4.
The instrument consists of a glass thermometer
inclosed in a metal case, the front portions of the
case being cut away so as to expose the scale above
and the mercury bulb below. As was explained
before, the thermometer is thrust deep into the
body of the ham so that the pointed end containing
the mercury bulb rests beside or a little behind
the upper portion of the femur, the bone being
used as a guide in introducing the thermometer.
Ham temperatures are taken at three stages in
the preparation for cure—(1) on the hanging floor,
just before the hams go to the chill rooms, in order
to determine the amount of heat lost prior to chilling;
(2) on leaving the chill rooms, in order to determine
the thoroughness of the chill;(3) on the
packing floor, just before the hams are placed in
pickle, as a further check on the thoroughness of
the chilling.
In taking the temperatures of hams which have
been chilled—and most of the temperatures are
taken subsequent to chilling—it is customary for
the packing-house attendant who has this matter
in charge to warm the thermometer by holding the
pointed or bulb end in his hand, so as to force the
mercury column up to about 60° F., or well above
the temperature of hams. The thermometer is
then thrust into the ham and allowed to remain
for several minutes, by which time the mercury
column will have fallen to the temperature of the
ham. The thermometer is then slowly withdrawn
so as to expose the top of the mercury column, and
an accurate reading is thus obtained of the inside
temperature of the ham. The thermometer is
warmed by the hand before each ham is tested, and
this undoubtedly insures more accurate readings
than would result were the thermometer removed
from one ham and plunged immediately into
another, but the procedure is open to certain
objections, for the open space between the
metal point of the thermometer and the mercury
bulb soon becomes filled with particles of meat and with grease and
dirt from the attendant’s hands, and it is at once apparent that a
thermometer in this condition would furnish a ready means whereby
extraneous matter might be introduced into the bodies of the hams.
In other words, a contaminated thermometer would furnish an excellent
means whereby hams could be inoculated with putrefactive
bacteria.
In order to determine whether hams actually become inoculated in
this manner, the following experiment was carried out:
EXPERIMENT TO SHOW WHETHER HAMS BECOME INFECTED FROM HAM THERMOMETERS.
This experiment was designed to show (1) whether the usual
packing-house method of taking ham temperatures was apt to induce
souring in the hams thus tested, and (2) whether souring would result
in hams which were tested with a thermometer purposely contaminated
with the bacillus isolated from sour hams.
The experiment was carried out as follows: Thirty hog carcasses
were selected as they entered the hanging floor from the killing floor.
They had been cleaned, eviscerated, and split, and were of the same
average weight and of sufficient size to yield hams weighing from 12
to 14 pounds. They were divided into three lots of 10 each and were
allowed to remain on the hanging floor for two hours, after which they
were given the usual 48-hour chilling.
Lot 1.—The hams in this lot were tested with an ordinary ham thermometer as they
entered the hanging floor, as they left the hanging floor, and as they left the coolers.
The thermometer used was borrowed from one of the plant attendants and was used in
the condition in which it was received from him; that is, it was not cleaned or disinfected
prior to use.
Lot 2.—The hams in this lot were tested as they entered the hanging floor with a
thermometer which had been previously cleaned and disinfected and then dipped in
a culture suspension of the meat-souring bacillus which was isolated from sour hams.
The thermometer was dipped in the culture suspension before each ham was tested.
No further temperatures were taken of these hams. The thermometer was carefully
cleaned and disinfected before it was returned to the attendant from whom it was
borrowed.
Lot 3.—The hams in this lot were not tested at all, and were intended as checks on
the cure.
The three lots of carcasses were carefully tagged and were chilled in
a special cooler to themselves. Upon leaving the cooler the hams
were cut from the carcasses and trimmed. The three lots of hams
were then cured in separate tierces. All of the hams were subjected to
exactly the same cure.
The pickles used were the regular pumping and regular curing
pickles of the establishment at which the experiment was carried out.
The hams in lot 3 were pumped first and those in lot 1 were
pumped next. The needle was then removed and a fresh, clean
needle was used for lot 2. This was done in order to prevent the
possibility of carrying over bacteria from one lot of hams to another
on the pumping needle. The tierces were thoroughly cleaned with
boiling water before being used. The curing was carried out in a
pickling cellar which was held at 33° to 36° F., the temperature never
rising above the latter figure. The tierces were rolled three times
during the curing. The details and results were as follows:
Tierce 1.—Contained 20 hams, half of which were pumped in both body and shank
and half in the shank only. These hams were taken from the carcasses in lot 1 and had
been tested several times with a ham thermometer, as already described.
Result: At the end of the cure it was found that of the 10 hams which were pumped
in the shank, 5 showed well-marked souring in the body, while of the 10 hams which
were pumped in both body and shank, 2 showed slight souring in the body.
Tierce 2.—Contained 20 hams, which were pumped in the same manner as those in
tierce 1. These hams were taken from the carcasses in lot 2 and had been tested once
with a thermometer which was dipped in a culture suspension of the bacillus isolated
from sour hams.
Result: The 10 hams which were pumped in the shank only all became sour. When
they were tried out at the end of the cure, they showed pronounced souring throughout
the entire body and were classed as “stinkers” by the meat inspector who examined
them. The souring extended through to the bone marrow of the femur in all of these
hams. Of the 10 hams which were pumped in both body and shank, 7 showed
well-marked souring in the body, but not as pronounced as in those pumped in the
shank only; in five of these hams the souring extended through to the bone marrow of
the femur, while in 2 the bone marrow remained sweet.
Tierce 3.—Contained 20 hams, which were pumped in the same manner as those in
the two preceding tierces. These hams were not tested with a thermometer, and were
put down as a check on the cure. They were pumped with the same pumping pickle,
subjected to the same cure, and held under precisely the same conditions as the hams
in the two preceding tierces.
Result: When tested at the end of the cure, all of these hams were found to be
perfectly sound and sweet.
Results of experiment to show whether hams become infected from ham thermometers.
| No. of tierce. |
Number of hams. |
Average weight of hams.
Pounds. |
How pumped. |
Treatment. |
Condition at end of cure. |
| Number of sour hams. |
Percentage of sour hams. |
| 1 |
20 |
12-14 |
10 in shank |
Tested in several stages in preparation for cure
which had not been cleaned. |
5 |
50 |
| 10 in body and shank |
do |
2 |
20 |
| 2 |
20 |
14-16 |
10 in shank |
Tested once with ham thermometer dipped
in culture suspension of anaerobic bacillus isolated
from sour hams. |
10 |
100 |
| 10 in body and shank |
do |
7 |
70 |
| 3 |
20 |
14-16 |
10 in shank |
Not tested with thermometer. |
0 |
0 |
| 10 in body and shank |
do |
0 |
0 |
Several hams from each tierce were examined bacteriologically.
cultures being taken from the meat near the bone and from the bone
marrow of the femur.
In the sour hams from tierce 1 cultures taken from the meat near
the bone showed the same anaerobic bacillus noted in other sour
hams (i. e., the same bacillus which caused souring in Experiments I
and II), but these cultures were contaminated with other bacteria
which were probably introduced on the thermometer along with the
ham-souring bacillus. None of the contaminating bacteria were
capable, however, of producing a sour-meat odor when grown on the
egg-pork medium. Pure cultures of the ham-souring bacillus were
obtained from the bone marrow of some of these hams, showing that
this bacillus had penetrated through to the bone marrow while the
other bacteria had not.
From the sour hams in tierce 2 the ham-souring bacillus was
recovered readily, and often in pure culture, from the hams which
had been pumped in the shank only, whereas it was usually contaminated
with pickle bacteria in the hams which had been pumped
in both body and shank.
In the case of the sound hams in tierce 3, cultures taken from the
meat near the bone and from the bone marrow of the femur were
negative in the hams which had been pumped in the shank only,
while cultures taken from corresponding points in the hams pumped
in both body and shank showed ordinary pickle bacteria, which had
evidently been introduced into the bodies of these hams in the pumping
pickles. None of these hams exhibited the slightest sour odor.
Summary of experiment.—In this experiment 20 hams (tierce 1)
were tested with an ordinary ham thermometer in the usual packing-house
manner. Half of these hams were subjected to the mild cure
and half were given the regular cure, with the result that 50 per cent
of those receiving the mild cure and 20 per cent of those receiving the
regular cure became sour.
A second lot of 20 hams (tierce 2) were tested with a thermometer
which had been purposely contaminated with a culture suspension of
the ham-souring bacillus. These hams were cured in the same manner
as the first lot, with the result that all of those receiving the mild
cure and 70 per cent of those receiving the regular cure became sour.
A third lot of 20 hams (tierce 3) which had not been tested at all
were cured in the same manner as the two preceding lots, as a check
on the cure. All of these hams were sweet at the end of the cure.
Inasmuch as the three lots of hams were cured under precisely the
same conditions and were handled in the same manner prior to pickling,
the only difference being that the hams in tierces 1 and 2 were
tested with the ham thermometer while those in tierce 3 were not,
we must conclude that the souring of the hams in tierces 1 and 2
resulted from the testing which these hams received. In the case
of tierce 1 the hams became infected from a thermometer which, in
the ordinary routine use of the packing house, had become accidentally
contaminated with the ham-souring bacillus. In the case
of tierce 2 the hams became infected from a thermometer which
had been artificially contaminated with the bacillus. The high
percentage of sours in this last lot is due to the fact that these
hams were heavily infected with the ham-souring bacillus, for owing
to the construction of the ham thermometer many thousands of the
bacilli were unquestionably introduced into each ham on the point
of the thermometer. In the ordinary routine of ham testing, where
hams become infected from foreign matter introduced on the thermometer,
the percentage of souring, as shown in tierce 1, would be
less, for it is not to be supposed that ham thermometers are always
contaminated with the ham-souring bacillus, but that they only
become so at times, and that probably only a few of the bacilli
are then introduced.
This experiment, we think, proves conclusively (1) that the ham-souring
bacillus may be introduced into the bodies of hams on the
thermometers used in testing the hams, and (2) that the packing-house
method of taking ham temperatures by means of a thermometer
which is thrust deep into the bodies of the hams may cause souring
in the hams thus tested.
As a further proof that hams may become contaminated in this
manner, a series of cultures were made from scrapings taken from
ham thermometers. The scrapings consisted of the accumulations
of bits of meat, grease, and dirt that collect on the thermometers,
and were taken from the thermometers while the latter were in
ordinary routine use in the packing house. In a series of six cultures
which were made from such scrapings at different times, the same
bacillus which was isolated from sour hams and shown to cause meat
souring was found three times. In other words, the ham-souring
bacillus was present in 50 per cent of the cultures made from thermometer
scrapings, and many hams undoubtedly become infected
from the thermometers. Souring would be almost certain to result
in mild-cure hams if these hams were tested with a thermometer
which had become accidentally contaminated with the ham-souring
bacillus, as the bacillus would have time to develop within the bodies
of the hams before being inhibited by the curing pickle, which penetrates
slowly into the bodies of these hams. In the case of regular
cure hams—that is, hams which are pumped in both body and shank—souring
would be much less apt to occur after the use of a contaminated
thermometer, as these hams are more or less saturated with a
strong pumping pickle at the beginning of the cure, which would
tend to inhibit the growth of any bacteria that might be introduced
on the thermometers.
The fact that souring may result in hams from the use of a contaminated
thermometer would explain the occurrence of several sours in
one vat, for in testing hams just before they go into cure several hams
are usually tested in succession, and these would in all likelihood go
into the same vat. Supposing the thermometer to have been contaminated
with the ham-souring bacillus at the time these hams were
tested, this would explain a fact which has been often noted, namely,
the occurrence of several sours in one vat while other vats containing
the same run of hams show no sours.
If souring resulted in all of the hams which are subjected to a thermometer
test in the daily routine of the packing house, this manipulation
alone might account for nearly all of the sours which occur, but
the experiment which has been just described shows that all of these
hams do not become sour. In tierce 1, where each ham was subjected
to three thermometer tests at different times, souring resulted in 35
percent (this includes both mild and regular cure) of the hams thus
tested, and in actual practice the percentage of sours in hams which
have been subjected to the thermometer test would probably be
somewhat less. Quite a large percentage of sour hams are thus left
unaccounted for by the thermometer test, and we believe that these
are chiefly the result of contamination carried in on the pumping
needles or in the pumping pickles.
INFECTION FROM PUMPING NEEDLES.
In view of the results obtained in the last experiment, in which it
was shown that hams may become infected from the use of ham thermometers,
it seemed not improbable that hams might also become
infected from the pumping needles, which, like the thermometers,
are thrust deep into the bodies of the hams beside the bone. In order
to throw some light upon this point, cultures were taken from the
grease and dirt that accumulate on the shields at the bases of the
pumping needles, as such material must undoubtedly be carried into
the hams at times on the needles. The ham-souring bacillus was
found several times in these cultures, and hence it is fair to infer that
hams may also become infected at times from the pumping needles,
just as they become infected from the thermometers. Bits of contaminated
meat and grease and particles of dirt carried in on the
pumping needles would be forced out into the hams by the pumping
pickle, which passes out through small openings or fenestræ in the
needles, and this probably affords one explanation as to why so many
more body sours occur in the mild-cure hams. In the mild-cure hams,
which are pumped in the shank only, the pumping needle is introduced
near the femorotibial articulation, and the shank is saturated
at the start with a strong brine solution, while the body of the ham is
not. If the ham-souring bacillus were carried into these hams on
the pumping needle, the growth of the bacillus in the shank would be
inhibited by the strong brine solution with which the shank is saturated,
but there would be nothing to prevent the bacillus from growing
upward into the body of the ham, which has not been pumped and is
free from pickle. This would also explain the fact that the souring
often starts at the knee joint and extends upward into the body of
the ham. In the case of the regular cure hams, where the ham is
pumped in both body and shank, the entire ham is more or less saturated
at the start with the strong brine of the pumping pickle, which
tends to inhibit the growth of the ham-souring bacillus even if this
bacillus should find its way into these hams on the pumping needles.
It is in the mild-cure or partly pumped hams, where the body of the
ham is left unpumped, that the ham-souring bacillus finds its best
opportunity for development, and the greater proportion of the sours
that occur in the packing house are found in these hams.
As regards the possibility of infection from the pumping pickle
itself, it does not seem probable that this would often occur, for the
pumping and curing pickles are always prepared on an upper floor of
the pickling houses and are delivered to the pickle cellars in closed
pipes, so the chances for the accidental contamination of these solutions
from floating dust or dirt would not be great. Furthermore,
the strong brine of the pumping pickle would completely inhibit the
growth of the ham-souring bacillus, and the bacillus would be incapable
of multiplying, even if it found its way into the pickle. On the
other hand, laboratory experiments show that the bacillus or its
spores may remain alive for a considerable length of time in the pumping
pickle, so the possibility of infection from this source can not be
overlooked.
INFECTION FROM BILLHOOKS.
After the hams are cut from the carcasses they are handled entirely
by means of billhooks. In handling the hams the hooks are inserted
beneath the skin of the shank at a point just above the tibio-femoral
articulation. The hooks should be inserted in the connective tissue
beneath the skin and should not penetrate the muscular tissue to
any depth. When the hams lie in the right position, with the butt
or large portion away from and the shank toward the operator, it is
an easy matter to pick them up in the proper manner; but when
they lie at different angles and are being rapidly handled it is almost
impossible to prevent the hook from penetrating the muscular tissues,
and if the hook should penetrate to the bone it might carry in foreign
matter contaminated with the meat-souring bacillus. It is not probable
that many hams become contaminated in this way, as the men
who handle the hams are very skillful in manipulating their hooks;
but the possibility that hams may become contaminated in this
manner should not be entirely overlooked.
The most favorable medium for the growth of the organism was
found to be the modified egg-meat mixture of Rettger, which has
been previously described. In this medium the organism develops
rapidly at a temperature of 20° to 25° C., giving rise to the characteristic
sour-meat odor. Like the bacillus described by Klein, it also
grows readily on pork-agar and pork-bouillon containing glucose,
but differs from Klein’s bacillus in that it will grow, though less luxuriantly,
on ordinary nutrient media—agar, gelatin, and bouillon—without
the addition of glucose.
The optimum temperature for growth is 20° to 25° C. The organism
does not grow at incubator temperature (37.5° C.). At ice-box
temperature (8° to 10° C.) it develops readily, although the growth
is less rapid than at 20° to 25° C. That the organism will develop at
even lower temperatures was shown in the inoculation experiments
with hams, where it developed and multiplied extensively in the
bodies of the hams at the temperature of the pickling cellars, which
are held usually at 34° to 36° F.(1° to 2° C.).
The organism develops best in a neutral or slightly alkaline
medium.
Growth on egg-pork medium.—At a temperature of 20° to 25° C.
the cultures show a slight but distinct sour odor in from two to three
days. This odor, as before stated, closely resembles the odor of a
sour ham. Egg-pork cultures from three to five days old were given
to a trained meat inspector, who knew nothing whatever as to the
contents of the tubes, and he was asked to describe the odor; he
described it as that of a sour ham.
At one week the albumins of the medium are gelatinized or partly
coagulated and the odor is more pronounced. At ten days the
albumins are completely coagulated except at the surface, where
there is no apparent growth; the odor is more putrefactive in nature,
and the reaction of the medium is slightly acid. At three weeks the
coagulated albumin splits up into fragments and appears to undergo
a slow digestion, gas bubbles form in the lower portion of the culture,
and the odor becomes distinctly putrefactive in character. The slow
digestion of the albumin is probably due to a proteolytic enzyme
elaborated by the bacillus.
At the end of a week a dark zone usually appears at the surface of
the coagulated albumin and gradually darkens until it becomes
almost black. This zone is probably due to a pigment elaborated by
the bacillus.
At ice-box temperature (8° to 10° C.) the same changes and the
same odor were noted, but were somewhat slower in developing.
Glucose-pork-agar.—This medium was prepared from pork in the
same manner as beef-agar, and contained 1 per cent of glucose. The
organism grows readily on this medium and may be conveniently
cultivated in deep stab cultures. The medium was always thoroughly
boiled and then rapidly cooled in order to expel the inclosed
air. The growth of the organism was found to vary considerably
with the reaction.
When the reaction was +1.5, deep stab cultures at three days (20°
to 25° C.) showed a well-marked arborescent growth, appearing as
delicate filaments extending outward from the line of stab. The
growth stopped within one-fourth or one-half inch of the surface of
the agar on account of the presence of oxygen in the upper part of
the culture medium. As the growth extended toward the walls of
the test tube the agar became clouded, and there were sometimes gas
bubbles in the depth of the agar, but the gas formation was not
extensive.
When the reaction of the agar is neutral or slightly alkaline, extensive
gas formation occurs and the agar is often much broken up.
The cultures developed a disagreeable, somewhat putrefactive
odor, but did not give the characteristic sour-ham odor obtained from
the egg-pork cultures.
The organism was also grown on anaerobic agar plates by Zinsser’s
method, which is said to give absolutely anaerobic conditions. The
colonies on agar have a cottony or woolly appearance at first, and
spread slowly, with slightly irregular margins.
In glucose-pork-agar to which azolitmin was added the azolitmin
in the lower portion of deep stab cultures was completely decolorized
in five days at room temperature (20° to 25° C).
In glucose-pork-agar containing neutral red the red color in the
lower portion of the tube was changed to yellow with the development
of fluorescence.
Neutral gelatin.—Tubes of ordinary neutral gelatin without the
addition of glucose were inoculated and held at ice-box temperature
(8° to 10° C). At five days a delicate white growth appeared along
the line of stab in the lower portion of the tube. At seven days the
growth showed fine radial striæ, presenting an arborescent or tree-like
appearance, and extended halfway from the line of stab to the
walls of the test tube. At two weeks the growth had caused a delicate
clouding of the medium in the lower portion of the tube. At
three weeks the gelatin in the lower portion of the tube had become
liquefied and the growth had settled to the bottom as a white precipitate.
In gelatin containing glucose, gas bubbles are formed in the depth
of the medium through the splitting up of the glucose, and the
characteristic arborescent growth is obscured.
Glucose-pork-bouillon.—This medium was prepared from pork
instead of beef and contained 1 per cent of glucose. The best results
were obtained when the reaction of the medium was neutral or
slightly alkaline.
Culture tubes, which had been previously boiled to expel the contained
air and then inoculated, were held in a Novy jar, in an atmosphere
of hydrogen at a temperature of 20° to 25° C. At three days
the tubes showed well-marked clouding. At one week the growth
appeared as a heavy, white, flocculent, cottony precipitate in the
bottom of the tubes with a slight flocculent precipitate above.
When the culture was removed from the jar and shaken, the heavy,
flocculent precipitate at the bottom of the tube broke up without
much difficulty, giving rise to a heavy uniform clouding with some
small floating masses, which soon settled to the bottom. On shaking
the tube some evolution of gas in the form of very fine bubbles was
noticed.
In Smith fermentation tubes containing neutral glucose-pork-bouillon
the closed arm of the tube shows well-marked clouding with gas
formation at three days at room temperature (20° to 25° C). The
growth has a tufted, cottony appearance, and there are many filaments
and threads. The growth settles to the bottom of the closed
arm as a cottony, white precipitate (see Pl. IV). The organism
splits the glucose vigorously, and at 10 days the tubes show from
40 to 50 per cent of gas. The bouillon in the open arm of the tube
remains unclouded. The maximum gas production at room temperature
is reached in from 10 to 14 days, by which time the growth in the
closed arm has completely settled into the bend of the tube, leaving
the bouillon in the closed arm clear. The gas formula, as determined
by Smith’s method, was H/CO₂= 5/1. The reaction of the bouillon becomes
acid to phenolphthalein.
The organism will grow on ordinary neutral bouillon without the
addition of glucose, and in Smith tubes containing this medium a
small amount of gas was formed, due to the splitting of the muscle
sugar.
The bacillus also grows in a sugar-free broth—that is, a broth free
from muscle sugar—and from cultures grown in this medium a well-marked
indol test was obtained.
Litmus-milk.—The organism was grown in litmus-milk in Smith
fermentation tubes at 20° to 25° C. At seven days the litmus in the
lower portion of the closed arm had assumed a brownish-buff color.
At two weeks the litmus in the closed arm had been reduced to a
brownish-buff color except at the top of the tube, where a pale,
bluish tinge remained, and the litmus in the open arm showed very
slight reddening as compared with a check tube. At three weeks the
litmus in the closed arm was entirely reduced to a light, brownish-buff
color, and the litmus in the open arm showed a slight but distinct
reddening as compared with the check. The reddening of the
litmus in the open arm was evidently due to the transfusion of acids
formed by the growth of the bacillus in the closed arm. After several
weeks the milk
is slowly peptonized,
probably as a result
of enzyme action.
The organism is a large bacillus having an average size of 4 to 8 μ
in length by 0.5 to 0.7 μ in thickness, but there are many longer forms
measuring from 10 to 20 μ in length. It develops in long, irregular
chains or filaments, which at times show a slightly spiral form.
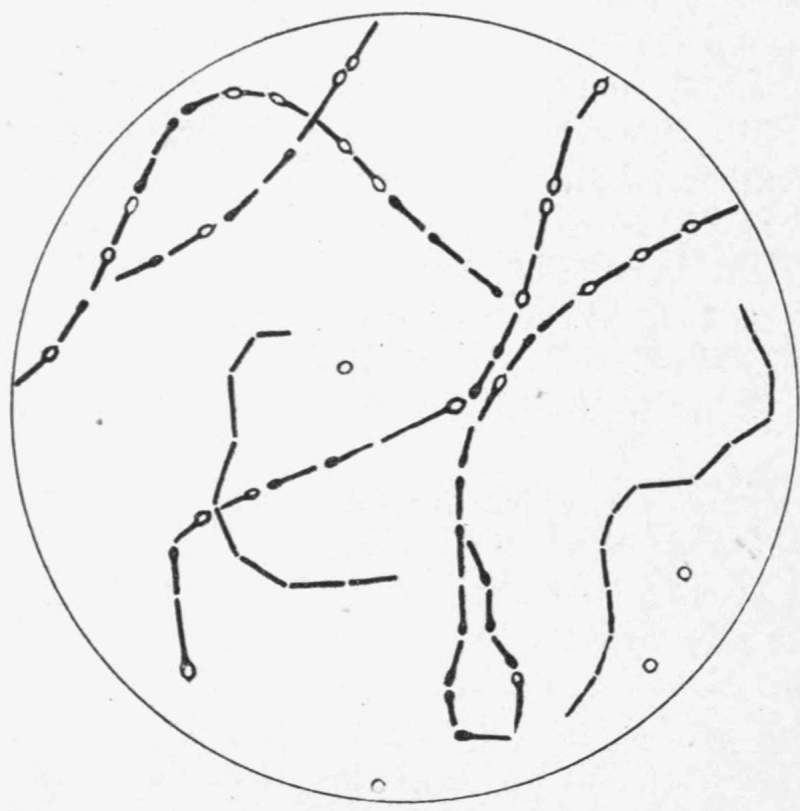
Fig. 5.—Ham-souring bacillus
(Bacillus putrefaciens) grown on egg-pork
medium, showing tendency to form chains. Partly developed and
fully developed spores are shown at ends of rods; also free spores.
(Pen-and-ink drawing made with camera lucida from preparation
stained by Gram’s method.× 640.)
The individual organisms show at times a widely open, slightly
spiral form, which was more apparent in hanging-drop preparations made
from bouillon cultures, where the organisms had been comparatively
undisturbed. This appearance was also noted at times in the stained
sections of soured muscular tissue, where the organisms were stained in
place. The organism possesses no motility. It stains with the ordinary
aniline dyes and by Gram’s method.
The organism develops large, terminal spores, which are at first
oval, but when fully developed are perfectly round and measure
from 1.5 to 2 μ in diameter.
Spores develop rapidly in the egg-pork medium at 20° to 25° C.,
fully developed spores being noted in from five to seven days. At
ice-box temperature (8° to 10° C.) partly developed spores were
noted in the egg-pork medium at 10 days and fully developed
spores at 2 weeks.
Occasional spores were noted in old agar and gelatin cultures,
but abundant spore formation was seen only in the egg-pork medium.
No spores were noted in bouillon cultures, even at 10 weeks.
In its vegetative form the bacillus is killed at 55° C. in 10 minutes.
The spores survive a temperature of 80° C. for 20 minutes, but are
killed at 100° C. in 10 minutes.
When sodium chlorid and potassium nitrate were added to glucose-pork
broth in varying amounts, it was found that 3 per cent of
sodium chlorid or 3 per cent of potassium nitrate was sufficient to
inhibit completely the growth of the bacillus at room temperature
(20° to 25° C.).
While the growth of the bacillus was inhibited by sodium chlorid
and potassium nitrate as just stated, it was found that very much
stronger solutions of the two salts failed to destroy the bacillus.
Thus it was found that the bacillus or its spores retained their vitality
after an exposure of 30 days in a solution containing 23 per cent of
sodium chlorid and 6 per cent of potassium nitrate.
The organism splits glucose, but not lactose or saccharose. That
it possesses the power of splitting muscle sugar was shown by the
formation of gas in Smith fermentation tubes containing ordinary
neutral bouillon without the addition of any sugar.
The formation of gas in glucose bouillon varies considerably with
the reaction of the medium. The largest amount of gas was formed
when the broth was neutral or slightly alkaline. When the reaction
of the broth was distinctly acid or distinctly alkaline the amount
of gas was diminished. The gas which is formed in bouillon cultures
consists chiefly of hydrogen and carbon dioxide. In order to collect
a sufficient amount of the gas for analysis, two large fermentation
tubes capable of holding 150 cubic centimeters each were constructed.
These tubes were filled with pork-bouillon and inoculated
with the bacillus. After 20 days at room temperature (20° to 25° C.)
the gas was collected and the carbon dioxide and hydrogen determined,
with the following result:
|
Cubic centimeters. |
| Total amount of gas collected |
37.7 |
| Carbon dioxide, by absorption with NaOH |
6.2 |
| Hydrogen, by difference |
31.5 |
This analysis gives an approximate gas formula of H/CO2= 5/1, which
agrees with the gas formula as determined in the small fermentation
tubes by Smith’s method.
In hams which had undergone spontaneous souring and in hams
which had been artificially soured by inoculation, hydrogen-sulphid
was often noted when the sour portions of the meat were tested
with lead-acetate paper, but no distinct odor of the gas could be
obtained. Hydrogen sulphid was also noted in egg-pork cultures of
the bacillus.
In glucose-bouillon, butyric and lactic acids are formed and the
reaction of the medium becomes distinctly acid. Butyric and lactic
acids were also noted in the egg-pork cultures.
A series of Smith fermentation tubes containing 10 c. c. each of
glucose-pork broth medium was inoculated with the bacillus and
held at room temperature (20° to 25° C.). These cultures were
titrated against [N/40]NaOH, with phenolphthalein as an indicator at
intervals of two days up to nineteen days, and then at two-week
intervals up to sixty-one days. Three of the cultures were titrated
each time so as to give a fair average of the acidity of the cultures,
and an uninoculated check tube was also titrated each time to see
if there was any change in the reaction of the medium. The results
of the titrations are shown in the following table:
Acidity determinations in glucose-pork broth cultures.
Age of culture
(days). |
Culture
A. |
Culture
B. |
Culture
C. |
Average. |
Medium. |
Acidity of
culture. |
|
|
|
|
|
|
Per cent. |
| 2 |
0.038 |
0.030 |
0.040 |
0.036 |
0.009 |
0.027 |
| 4 |
.105 |
.100 |
.102 |
.102 |
.009 |
.093 |
| 6 |
.106 |
.110 |
.109 |
.108 |
.009 |
.099 |
| 8 |
.124 |
.115 |
.117 |
.119 |
.009 |
.110 |
| 10 |
.128 |
.130 |
.126 |
.128 |
.009 |
.119 |
| 12 |
.129 |
.120 |
.129 |
.126 |
.009 |
.117 |
| 19 |
.126 |
.125 |
.125 |
.125 |
.009 |
.116 |
| 33 |
.125 |
.123 |
.125 |
.124 |
.009 |
.115 |
| 47 |
.122 |
.120 |
.121 |
.121 |
.009 |
.112 |
| 61 |
.121 |
.116 |
.119 |
.118 |
.009 |
.109 |
From the above table it will be seen that the maximum acidity
was reached at ten days, after which there was a gradual reduction
in the acidity, due probably to the formation of ammonia compounds.
Rabbits, guinea pigs, and white mice were inoculated and fed with
cultures of the bacillus without effect, from which it would appear
that the bacillus possesses no pathogenic or disease-producing
properties.
The bacillus is essentially a saprogenic bacterium with zymogenic
properties. A preliminary study of the chemical changes which take
place in sour hams shows that these changes are of a putrefactive
nature. Hams which had undergone spontaneous souring were compared
with hams which had been artificially soured by inoculation,
and the chemical changes were found to be identical. A chemical
study was also made of the changes taking place in egg-pork cultures
of the bacillus at different stages of growth, and these changes were
found to be of a putrefactive nature and similar in character to the
changes which occur in sour hams. Among the putrefactive products
formed by the growth of the bacillus in the egg-pork medium were
indol, skatol, volatile fatty acids, skatol-carbonic acid, and hydrogen
sulphid.[4]
Bul. 132, Bureau of Animal Industry, U. S. Dept. of Agriculture. Plate IV.
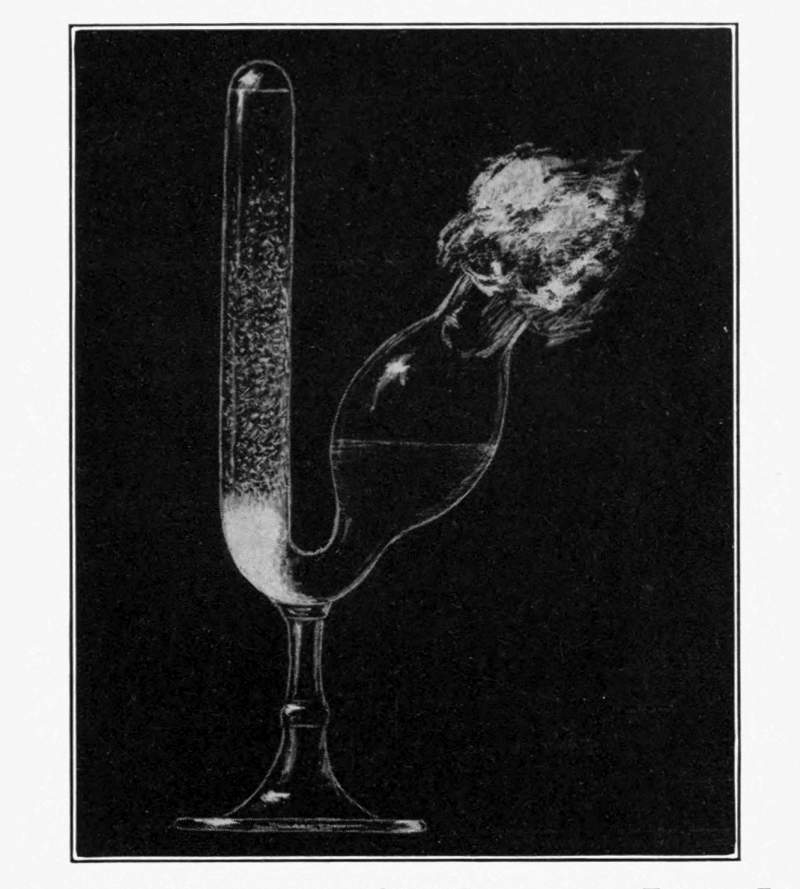
Glucose Bouillon Culture in Smith Fermentation Tube at Four
Days. Culture Grown at Room Temperature (20° to 25° C.).
Growth Confined Entirely to Closed Arm, with Gas Collecting
at Top.
A more extended study is now being carried on in the Biochemic
Division of the chemical changes which take place in hams during
the process of souring, together with a further study of the chemical
changes which result from the growth of the bacillus in the egg-pork
medium. The results of this investigation will be given in a later
paper.
The bacillus described in this paper belongs to the class of putrefactive
anaerobes, which are widely distributed in nature in dust, soil,
and excrementitious matters. This group of bacteria contains both
pathogenic and nonpathogenic forms. The former have received
considerable attention, but the latter have never been thoroughly
cleared up. The bacillus isolated from sour hams belongs in the latter
category, being possessed of no pathogenic or disease-producing properties.
It occurs in the dust and dirt of the packing house and finds
its way into the hams in the various manipulations to which the hams
are subjected.
The bacillus described in this paper does not seem to correspond
with any forms heretofore described. It differs from Klei bacillus
(Bacillus fœdans) in the following important particulars:(1) It forms
large terminal spores, whereas Klein’s bacillus formed no spores;(2) it
will grow at a temperature of 34° F., while Klei bacillus did not grow
below 50° F.;(3) it produces an acid reaction in culture media, while
Klei bacillus gave a distinctly alkaline reaction;(4) it will grow on
the ordinary nutrient media—gelatin, agar, and broth—without the
addition of glucose, while Klein’s bacillus did not;(5) it peptonizes
the casein in milk, whereas Klein’s bacillus had no action on milk;
(6) it liquefies gelatin more rapidly, causing complete liquefaction
after three weeks at 8° to 10° C., whereas Klein’s bacillus caused only
partial liquefaction after eight weeks at 20° C.;(7) it can be conveyed
from turbid broth cultures to new culture material by means of the
platinum loop, whereas Klein’s bacillus could not be thus conveyed.
For the bacillus described in the present paper the following name
is proposed:Bacillus putrefaciens.
As it has been shown that souring in hams results from the growth
of a bacterium which is introduced into the bodies of the hams in the
various manipulations which the hams undergo, the only way to eliminate
souring in hams, as they are cured in the larger packing establishments,
would be to cure the hams under aseptic or sterile conditions,
which would, of course, be a physical impossibility.
While it will probably be impossible, therefore, to eliminate souring
entirely under the methods of ham curing which are at present employed
in the larger packing establishments, much can undoubtedly
be done toward reducing the percentage of sours. In the matter of
taking ham temperatures, for instance, if the thermometers used were
thoroughly cleaned and disinfected and the surfaces of the hams
seared at the point where the thermometer is introduced, infection
from this source could be entirely prevented; or it might be possible
so to regulate the temperature of the chill rooms that the taking of
ham temperatures could be discontinued.
The elimination of the souring that results from the introduction
of foreign matter on the pumping needles could be effected in two
ways only,(1) by not pumping the hams at all, or (2) by pumping
them under sterile or aseptic conditions. As has been stated before,
some of the smaller packing establishments cure their hams without
pumping, and in these establishments the percentage of sours runs
very low. When hams are cured without pumping, however, the
period of curing has to be materially lengthened in order to give the
curing pickles sufficient time to penetrate thoroughly, and this is
what the larger plants wish to avoid because of the greater space and
greater number of vats which would be necessitated. The object of
pumping in the larger plants, where the number of hams handled
daily runs into the thousands, is to hasten the cure and thus prevent
the accumulation of a great number of hams at one time. It is
doubtful, therefore, whether the larger packing houses could conveniently
discontinue pumping.
To pump the hams under aseptic conditions would necessitate a
technique far too elaborate for routine use in the packing house; in
fact, anything like complete asepsis would be out of the question.
Certain measures might be adopted, however, that would tend to
prevent the possible introduction of ham-souring bacilli in the process
of pumping. It would undoubtedly be safer, for instance, to
boil the pumping pickle before use, and the chances of carrying in
contaminated foreign matter on the pumping needles could be lessened
by sterilizing the pumps and needles with boiling water and by frequently
dipping the needles, while in use, in boiling water. If the
hams were sprayed with clean water just prior to pumping, there
would be less likelihood of carrying in foreign matter on the needles.
The danger of introducing contaminated foreign matter on the needles
might be further obviated by searing the surfaces of the hams at
the points where the needles are introduced; but such a procedure
would be hardly practicable in the larger packing houses, where the
great number of hams cured necessitates rapid handling.
While the danger of possible contamination in pumping, through
the introduction of contaminated foreign matter on the pumping
needles, can not well be avoided, this danger is partly counterbalanced
by the inhibitory action of the pumping pickle, which is strikingly
shown in the experiments which have been described. In these
experiments, 100 hams received large doses of the ham-souring bacillus,
half of these hams being subjected to the mild cure and half to the
regular cure, with the following result: In the case of the mild-cure
hams, which were pumped in the shank only, the percentage
of sours was practically 100 per cent, every ham with possibly one
exception becoming sour; whereas in the regular-cure hams, which
were pumped in both body and shank, only 58 per cent of the hams
became sour. In other words, the additional pumping which the
regular-cure hams received served to prevent souring in 42 per cent
of these hams. In these experiments the number of bacteria introduced
into the hams was very great, thousands and even millions of
the bacilli being introduced into each ham, whereas in the routine of
the packing house it is not likely that more than a few of the bacilli
are ever introduced at one time on the thermometers and pumping
needles. In view of these results it is safe to say that in the larger
packing houses, where pumping seems to be necessary, the number
of sours could be reduced fully 50 per cent if all hams were pumped in
the body as well as in the shank.
At present the usual procedure is to pump all hams, both mild and
regular cure, with the same pumping pickle, the mild-cure hams
being pumped in the shank only and the regular-cure hams at two
additional points in the body. The experiments quoted above
show that the additional pumping which the regular-cure hams
receive undoubtedly tends to prevent the development of souring
in these hams, and this result is unquestionably due to the inhibitory
action of the salts contained in the pumping pickle, as it was found
by laboratory experiment that the addition of 3 per cent of sodium
chlorid to culture media is sufficient to inhibit the growth of the
ham-souring bacillus. The pumping pickles consist of strong brine
solutions and always contain considerably more than 3 per cent of
sodium chlorid. If, therefore, the pumping of regular-cure hams
were made more thorough than at present, and all of the deeper portions
of the ham were thoroughly saturated with the strong brine
solution, souring could be largely eliminated, if not entirely prevented,
in these hams, as an unfavorable medium or soil would thus be
created in which the ham-souring bacillus could not develop. The
ham-souring bacillus is able to develop within the bodies of the
regular-cure hams because the pumping of these hams is not always
thorough and there are certain areas in the inner or deeper portions
of the hams in which the tissues are not thoroughly saturated with
the pumping pickle.
Under the present methods of curing, the greater proportion of
the sours occur among the partly pumped or mild-cure hams. These
hams are pumped in the shank only, and the growth of the ham-souring
bacillus within the bodies of these hams is not interfered
with until the curing pickle has penetrated from the outside. As
it requires several weeks for the curing pickle to penetrate thoroughly
into the deeper portions of these hams, the bacillus is thus
afforded a considerable interval in which to develop before it is
exposed to the inhibitory action of the pickle. If these hams
could be thoroughly pumped in the body at the beginning of the cure
in the same manner as the regular-cure hams, the chief loss from
ham souring would be eliminated. It would not do, however, to
pump these hams in the body with the same pumping pickle used in
the regular cure, as the meat would be rendered too salty and the
mild flavor of the ham would be lost. There is undoubtedly a demand
for mild-cure hams, otherwise they would not be on the market; and
the question then arises how to pump these hams and still retain a
mild cure. This might be accomplished by pumping these hams
with their own curing pickle, which is usually a milder pickle than
that employed in the regular cure, or an even milder pumping pickle
might be used. If mild-cure hams were pumped in this way, the
percentage of souring in these hams could undoubtedly be greatly
diminished without materially affecting the flavor of the ham.
To recapitulate briefly, the prevention of ham souring is to be
sought in two ways:(1) Through greater care in handling the
hams and the adoption of precautionary measures to prevent the introduction
of the ham-souring bacillus into the bodies of the hams,
and (2) through more thorough pumping of the deeper or inner portions
of the hams, so as to create an unfavorable soil or medium in
which the ham-souring bacillus can not develop even if it should
gain entrance into the bodies of the hams.
From what has been said it will be apparent that ham souring
can probably never be entirely eliminated from the packing house
under the present methods of curing, but the adoption of precautionary
measures in testing and pumping hams, together with a more
thorough pumping of all hams in ways similar to those suggested,
would unquestionably reduce very materially the losses from this
source.
1. In this paper it has been shown that ham souring, as encountered
in the wet cure where the hams are entirely submerged in pickling
fluids, is due to the growth of an anaerobic bacillus within the bodies of
the hams. This bacillus (B. putrefaciens) was found in sour hams
obtained from four different packing establishments. It was isolated
and grown in various laboratory media, in one of which, the egg-pork
medium, it gave rise to the characteristic sour-ham odor.
This bacillus was the only organism that could be isolated from sour
hams that was capable of producing the characteristic sour-ham odor
in the egg-pork medium.
2. When injected into the bodies of sound hams, the bacillus
caused these hams to sour in the process of curing. In hams which
had been inoculated with the bacillus and thus artificially soured, the
bacillus was recovered in cultures taken at points far removed,
relatively speaking, from the point of inoculation, indicating that
the bacillus had multiplied and progressed by extension throughout
the bodies of the hams.
3. The bacillus possesses no motility, and its extension throughout
the bodies of the hams is a result of multiplication. In its growth
it follows along the connective-tissue bands between the muscle
bundles, which are composed of comparatively loose tissue and
afford paths of least resistance. When it invades the muscle tissue
proper, it follows along the sarcolemma sheaths between the muscle
fibers. As a result of this growth the muscular tissue becomes softer
and tends to break more easily.
4. The bacillus belongs to the class of putrefactive anaerobes
which are widely distributed in nature in dust, soil, and excrementitious
matters. The bacillus or its spores is present in the dust and
dirt of packing houses and finds its way into the hams in the various
manipulations to which they are subjected.
5. The bacillus or its spores may be introduced into hams on the
thermometers used in testing the hams, on the pumping needles,
and possibly on the billhooks used in handling the hams. It may
also be carried into the hams in the pumping pickle, and may even
find its way into the hams from the curing pickle, although infection
through the latter channel probably does not often occur.
6. The bacillus develops in the deeper portions of the ham because
of the anaerobic conditions there prevailing, and souring is most
often encountered, therefore, in the deeper portions of the ham
near the bone.
7. A preliminary study of the chemical changes which take place
in the process of souring shows that these changes are of a putrefactive
nature, and ham souring, as ordinarily encountered, is to be
regarded as an incipient putrefaction. Hams which had been
artificially soured by injections of culture were compared with sour
hams obtained from the packing house, and the putrefactive changes
were found to be identical.
8. Hams which have once become sour can never be restored to a
sound condition, because of the chemical changes which result from
the growth of the bacillus. In other words, the tissues of the ham
undergo certain chemical changes in the process of souring, and
when these changes have once taken place the tissues can never be
restored to a sound condition. The repumping of slightly soured
hams with a strong pumping pickle will check further souring, by
inhibiting the growth of the bacillus, but will not restore to a sound
condition those portions of the ham which have become sour.
9. The salts of the pickling fluids have a marked inhibitory action
on the ham-souring bacillus, and sours occur less frequently in regular-cure
hams.
10. In regular-cure hams the growth of the ham-souring bacillus
is restricted and often completely inhibited as a result of the additional
pumping which these hams receive, whereby they are more
or less saturated with pickle at the beginning of the cure.
11. If the pumping of regular-cure hams were more thorough and
all of the deeper portions of the ham were thoroughly saturated
with the pumping pickle, souring could be largely eliminated if not
entirely prevented in the hams, as an unfavorable medium or soil
would thus be created, in which the ham-souring bacillus could not
develop. The reason that souring does develop in regular-cure hams
is because the pumping is not always thorough and there are certain
areas in the deeper portions of these hams which are not saturated
with the pumping pickle.
12. Under the present methods of curing, the partly pumped or
mild-cure hams furnish the greater proportion of the sours, as these
hams are not pumped in the body and the growth of the ham-souring
bacillus within the bodies of these hams is not interfered
with until the curing pickle has penetrated from the outside. As
it requires several weeks for the curing pickle to penetrate thoroughly
into the deeper portions of these hams, the bacillus is thus afforded
a considerable interval in which to develop.
13. The percentage of souring in the mild-cure hams could be
greatly reduced without materially affecting the cure by pumping
these hams with their own curing pickle, which is usually a milder
pickle than that employed in the regular cure; and if the pumping
were thorough the number of sours in these hams could be reduced
to a small figure.
14. The only way by which ham souring could be entirely eliminated
from the larger packing establishments under the present methods
of curing would be to handle the hams throughout under aseptic
conditions, and this, for obvious reasons, would be an impossibility.
The losses from ham souring may be materially reduced, however, by
greater care in handling the hams and the adoption of precautionary
measures designed to prevent the introduction of contaminated
foreign matter into the bodies of the hams, together with more
thorough methods of pumping.
In conclusion, the writer desires to express his obligations to Dr.
S. E. Bennett, of the Inspection Division, inspector in charge at
Chicago, for the assignment of trained meat inspectors to assist in
the work, as well as for kind assistance in obtaining data and material
for laboratory study, and to Dr. L. E. Day, of the Pathological
Division, who kindly prepared the sections which are figured and
described in the present article.